Q9ASW1
Gene name |
GALT3 |
Protein name |
Hydroxyproline O-galactosyltransferase GALT3 |
Names |
Beta-1,3-galactosyltransferase 16 |
Species |
Arabidopsis thaliana (Mouse-ear cress) |
KEGG Pathway |
ath:AT3G06440 |
EC number |
|
Protein Class |
|
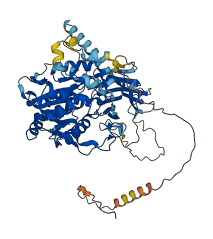
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q9ASW1
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q9ASW1-F1 | Predicted | AlphaFoldDB |
68 variants for Q9ASW1
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| tmp_3_1975248_T_C | 9 | R>G | No | 1000Genomes | |
| tmp_3_1975152_G_C | 41 | Q>E | No | 1000Genomes | |
| ENSVATH05783857 | 45 | T>N | No | 1000Genomes | |
| ENSVATH05783856 | 48 | V>M | No | 1000Genomes | |
| tmp_3_1975089_C_A | 62 | A>S | No | 1000Genomes | |
| ENSVATH00309428 | 65 | P>S | No | 1000Genomes | |
| ENSVATH05783855 | 66 | H>Q | No | 1000Genomes | |
| tmp_3_1975068_T_A | 69 | T>S | No | 1000Genomes | |
| tmp_3_1975059_C_G | 72 | D>H | No | 1000Genomes | |
| tmp_3_1975030_G_T | 81 | S>R | No | 1000Genomes | |
| tmp_3_1975029_A_G | 82 | F>L | No | 1000Genomes | |
| ENSVATH05783854 | 88 | V>L | No | 1000Genomes | |
| ENSVATH10526430 | 93 | L>F | No | 1000Genomes | |
| ENSVATH10526429 | 94 | V>I | No | 1000Genomes | |
| tmp_3_1974883_A_C | 130 | N>K | No | 1000Genomes | |
| ENSVATH02118811 | 131 | R>K | No | 1000Genomes | |
| ENSVATH02118810 | 136 | Y>S | No | 1000Genomes | |
| ENSVATH02118809 | 139 | G>D | No | 1000Genomes | |
| ENSVATH00309426 | 148 | I>N | No | 1000Genomes | |
| ENSVATH02118808 | 156 | F>Y | No | 1000Genomes | |
| ENSVATH00309425 | 158 | K>T | No | 1000Genomes | |
| ENSVATH02118807 | 165 | H>N | No | 1000Genomes | |
| ENSVATH02118806 | 166 | V>L | No | 1000Genomes | |
| ENSVATH00309424 | 183 | V>A | No | 1000Genomes | |
| ENSVATH05783853 | 189 | H>L | No | 1000Genomes | |
| ENSVATH05783852 | 201 | G>A | No | 1000Genomes | |
| ENSVATH00309421 | 207 | R>C | No | 1000Genomes | |
| ENSVATH05783849 | 213 | R>H | No | 1000Genomes | |
| ENSVATH02118805 | 241 | Q>P | No | 1000Genomes | |
| ENSVATH05783846 | 262 | G>D | No | 1000Genomes | |
| ENSVATH05783844 | 269 | S>N | No | 1000Genomes | |
| ENSVATH05783843 | 271 | N>S | No | 1000Genomes | |
| ENSVATH00309416 | 276 | M>I | No | 1000Genomes | |
| ENSVATH02118804 | 290 | G>R | No | 1000Genomes | |
| tmp_3_1974319_A_C | 293 | F>V | No | 1000Genomes | |
| ENSVATH00309414 | 296 | A>T | No | 1000Genomes | |
| tmp_3_1974268_C_A | 310 | G>W | No | 1000Genomes | |
| ENSVATH05783839 | 323 | E>K | No | 1000Genomes | |
| ENSVATH10526425 | 328 | S>N | No | 1000Genomes | |
| tmp_3_1974127_G_A | 333 | S>L | No | 1000Genomes | |
| ENSVATH00309410 | 338 | I>M | No | 1000Genomes | |
| ENSVATH00309407 | 369 | T>A | No | 1000Genomes | |
| ENSVATH05783837 | 371 | I>L | No | 1000Genomes | |
| tmp_3_1973996_C_T | 377 | V>I | No | 1000Genomes | |
| ENSVATH05783833 | 398 | E>D | No | 1000Genomes | |
| ENSVATH10526343 | 419 | V>D | No | 1000Genomes | |
| ENSVATH10526342 | 420 | N>H | No | 1000Genomes | |
| ENSVATH00309399 | 420 | N>S | No | 1000Genomes | |
| ENSVATH00309398 | 427 | S>Y | No | 1000Genomes | |
| ENSVATH10526341 | 428 | K>T | No | 1000Genomes | |
| ENSVATH05783830 | 453 | C>F | No | 1000Genomes | |
| ENSVATH00309395 | 459 | V>L | No | 1000Genomes | |
| tmp_3_1973561_G_A | 461 | P>L | No | 1000Genomes | |
| tmp_3_1973547_T_G | 466 | M>L | No | 1000Genomes | |
| ENSVATH00309392 | 486 | R>K | No | 1000Genomes | |
| ENSVATH05783821 | 513 | P>H | No | 1000Genomes | |
| ENSVATH00309390 | 518 | P>H | No | 1000Genomes | |
| ENSVATH00309389 | 534 | S>A | No | 1000Genomes | |
| ENSVATH02118796 | 551 | G>R | No | 1000Genomes | |
| ENSVATH05783805 | 569 | Q>E | No | 1000Genomes | |
| tmp_3_1973026_G_A | 583 | H>Y | No | 1000Genomes | |
| tmp_3_1973020_T_A | 585 | S>C | No | 1000Genomes | |
| ENSVATH10526336 | 590 | N>K | No | 1000Genomes | |
| ENSVATH05783803 | 598 | T>N | No | 1000Genomes | |
| ENSVATH05783802 | 615 | S>T | No | 1000Genomes | |
| ENSVATH05783801 | 618 | C>R | No | 1000Genomes | |
| tmp_3_1972916_T_G | 619 | E>D | No | 1000Genomes | |
| ENSVATH05783800 | 620 | E>E | No | 1000Genomes |
No associated diseases with Q9ASW1
1 regional properties for Q9ASW1
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Galectin, carbohydrate recognition domain | 165 - 344 | IPR001079 |
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| Golgi apparatus | A membrane-bound cytoplasmic organelle of the endomembrane system that further processes the core oligosaccharides (e.g. N-glycans) added to proteins in the endoplasmic reticulum and packages them into membrane-bound vesicles. The Golgi apparatus operates at the intersection of the secretory, lysosomal, and endocytic pathways. |
| Golgi membrane | The lipid bilayer surrounding any of the compartments of the Golgi apparatus. |
| integral component of membrane | The component of a membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
4 GO annotations of molecular function
| Name | Definition |
|---|---|
| carbohydrate binding | Binding to a carbohydrate, which includes monosaccharides, oligosaccharides and polysaccharides as well as substances derived from monosaccharides by reduction of the carbonyl group (alditols), by oxidation of one or more hydroxy groups to afford the corresponding aldehydes, ketones, or carboxylic acids, or by replacement of one or more hydroxy group(s) by a hydrogen atom. Cyclitols are generally not regarded as carbohydrates. |
| galactosyltransferase activity | Catalysis of the transfer of a galactosyl group to an acceptor molecule, typically another carbohydrate or a lipid. |
| glycosyltransferase activity | Catalysis of the transfer of a glycosyl group from one compound (donor) to another (acceptor). |
| hydroxyproline O-galactosyltransferase activity | Catalysis of the transfer of galactose from UDP-galactose to hydroxyproline residues present in the peptide backbone. |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| arabinogalactan protein metabolic process | The chemical reactions and pathways involving a cell wall arabinogalactan II glycoprotein, which is composed of a group of core protein of highly varying length and domain complexity. These are O-glycosylated at one or more hydroxyproline residues by arabinogalactan (AG) type II groups, which consist of (1->3)-beta-galactan and (1->6)-beta-linked galactan chains connected to each other by (1->3,1->6)-linked branch points, O-3 and O-6 positions substituted with terminal arabinosyl residues. Also, rhamnose, fucose, glucuronic and galacturonic acid can be present in the glycan structures. |
| mucilage biosynthetic process involved in seed coat development | The chemical reactions and pathways resulting in the formation of mucilage that occur as part of seed coat development; mucilage is normally synthesized during seed coat development. |
| protein O-linked glycosylation via hydroxyproline | The glycosylation of proteins via 04 atom of hydroxyproline to form O4-glycosyl-L-hydroxyproline; the most common form is arabinofuranosyl-4-proline. |
| root hair cell development | The process whose specific outcome is the progression of a root hair cell over time, from its formation to the mature state. |
11 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| Q8BG28 | B3galnt2 | UDP-GalNAc:beta-1,3-N-acetylgalactosaminyltransferase 2 | Mus musculus (Mouse) | PR |
| Q864U6 | B3GALNT1 | UDP-GalNAc:beta-1,3-N-acetylgalactosaminyltransferase 1 | Sus scrofa (Pig) | PR |
| A7XDQ9 | GALT2 | Hydroxyproline O-galactosyltransferase GALT2 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q8GXG6 | GALT4 | Hydroxyproline O-galactosyltransferase GALT4 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q8L7F9 | GALT1 | Beta-1,3-galactosyltransferase GALT1 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q8RX55 | GALT5 | Hydroxyproline O-galactosyltransferase GALT5 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q9LV16 | GALT6 | Hydroxyproline O-galactosyltransferase GALT6 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q5XEZ1 | HPGT3 | Hydroxyproline O-galactosyltransferase HPGT3 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q94F27 | HPTG1 | Hydroxyproline O-galactosyltransferase HPGT1 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q6P3P5 | b3gnt5 | Lactosylceramide 1,3-N-acetyl-beta-D-glucosaminyltransferase | Xenopus tropicalis (Western clawed frog) (Silurana tropicalis) | PR |
| Q5M900 | b3galnt2 | UDP-GalNAc:beta-1,3-N-acetylgalactosaminyltransferase 2 | Xenopus tropicalis (Western clawed frog) (Silurana tropicalis) | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MKQFMSVVRF | KFGFTSVRMR | DWSVGVSIMV | LTLIFIIRYE | QSDHTHTVDD | SSIEGESVHE |
| 70 | 80 | 90 | 100 | 110 | 120 |
| PAKKPHFMTL | EDLDYLFSNK | SFFGEEEVSN | GMLVWSRMRP | FLERPDALPE | TAQGIEEATL |
| 130 | 140 | 150 | 160 | 170 | 180 |
| AMKGLVLEIN | REKRAYSSGM | VSKEIRRICP | DFVTAFDKDL | SGLSHVLLEL | PCGLIEDSSI |
| 190 | 200 | 210 | 220 | 230 | 240 |
| TLVGIPDEHS | SSFQIQLVGS | GLSGETRRPI | ILRYNVNFSK | PSIVQNTWTE | KLGWGNEERC |
| 250 | 260 | 270 | 280 | 290 | 300 |
| QYHGSLKNHL | VDELPLCNKQ | TGRIISEKSS | NDDATMELSL | SNANFPFLKG | SPFTAALWFG |
| 310 | 320 | 330 | 340 | 350 | 360 |
| LEGFHMTING | RHETSFAYRE | KLEPWLVSAV | KVSGGLKILS | VLATRLPIPD | DHASLIIEEK |
| 370 | 380 | 390 | 400 | 410 | 420 |
| LKAPSLSGTR | IELLVGVFST | GNNFKRRMAL | RRSWMQYEAV | RSGKVAVRFL | IGLHTNEKVN |
| 430 | 440 | 450 | 460 | 470 | 480 |
| LEMWRESKAY | GDIQFMPFVD | YYGLLSLKTV | ALCILGTKVI | PAKYIMKTDD | DAFVRIDELL |
| 490 | 500 | 510 | 520 | 530 | 540 |
| SSLEERPSSA | LLYGLISFDS | SPDREQGSKW | FIPKEEWPLD | SYPPWAHGPG | YIISHDIAKF |
| 550 | 560 | 570 | 580 | 590 | 600 |
| VVKGHRQRDL | GLFKLEDVAM | GIWIQQFNQT | IKRVKYINDK | RFHNSDCKSN | YILVHYQTPR |
| 610 | |||||
| LILCLWEKLQ | KENQSICCE |