P0A8N3
Gene name |
lysS (asuD, herC, b2890, JW2858) |
Protein name |
Lysine--tRNA ligase |
Names |
Lysyl-tRNA synthetase, LysRS |
Species |
Escherichia coli (strain K12) |
KEGG Pathway |
eco:b2890 |
EC number |
6.1.1.6: Ligases forming aminoacyl-tRNA and related compounds |
Protein Class |
|
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
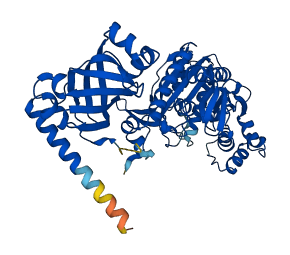
Autoinhibited structure

Activated structure
5 structures for P0A8N3
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| 1BBU | X-ray | 270 A | A | 2-505 | PDB |
| 1BBW | X-ray | 270 A | A | 2-505 | PDB |
| 1KRS | NMR | - | A | 31-149 | PDB |
| 1KRT | NMR | - | A | 31-149 | PDB |
| AF-P0A8N3-F1 | Predicted | AlphaFoldDB |
No variants for P0A8N3
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for P0A8N3 | |||||
No associated diseases with P0A8N3
5 regional properties for P0A8N3
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Aminoacyl-tRNA synthetase, class II (D/K/N) | 162 - 501 | IPR004364 |
| domain | OB-fold nucleic acid binding domain, AA-tRNA synthetase-type | 68 - 146 | IPR004365 |
| domain | Aminoacyl-tRNA synthetase, class II | 184 - 503 | IPR006195 |
| domain | Lysyl-tRNA synthetase, class II, C-terminal | 177 - 503 | IPR018149 |
| domain | Lysine-tRNA ligase, class II, N-terminal | 67 - 174 | IPR044136 |
Functions
| Description | ||
|---|---|---|
| EC Number | 6.1.1.6 | Ligases forming aminoacyl-tRNA and related compounds |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
2 GO annotations of cellular component
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ligase activity | Catalysis of the joining of two molecules, or two groups within a single molecule, using the energy from the hydrolysis of ATP, a similar triphosphate, or a pH gradient. |
| lysine-tRNA ligase activity | Catalysis of the reaction: ATP + L-lysine + tRNA(Lys) = AMP + diphosphate + L-lysyl-tRNA(Lys). |
| magnesium ion binding | Binding to a magnesium (Mg) ion. |
| tRNA binding | Binding to a transfer RNA. |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| lysyl-tRNA aminoacylation | The process of coupling lysine to lysyl-tRNA, catalyzed by lysyl-tRNA synthetase. The lysyl-tRNA synthetase is a class-II synthetase. The activated amino acid is transferred to the 3'-OH group of a lysine-accetping tRNA. |
| tRNA aminoacylation for protein translation | The synthesis of aminoacyl tRNA by the formation of an ester bond between the 3'-hydroxyl group of the most 3' adenosine of the tRNA and the alpha carboxylic acid group of an amino acid, to be used in ribosome-mediated polypeptide synthesis. |
7 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| P32048 | MSK1 | Lysine--tRNA ligase, mitochondrial | Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) | PR |
| P15180 | KRS1 | Lysine--tRNA ligase, cytoplasmic | Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) | PR |
| P0A8N5 | lysU | Lysine--tRNA ligase, heat inducible | Escherichia coli (strain K12) | PR |
| Q6F2U9 | Os03g0586800 | Lysine--tRNA ligase | Oryza sativa subsp japonica (Rice) | PR |
| Q22099 | kars-1 | Lysine--tRNA ligase | Caenorhabditis elegans | PR |
| Q9ZPI1 | At3g11710 | Lysine--tRNA ligase, cytoplasmic | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q43776 | LYSRS | Lysine--tRNA ligase | Solanum lycopersicum (Tomato) (Lycopersicon esculentum) | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSEQHAQGAD | AVVDLNNELK | TRREKLANLR | EQGIAFPNDF | RRDHTSDQLH | AEFDGKENEE |
| 70 | 80 | 90 | 100 | 110 | 120 |
| LEALNIEVAV | AGRMMTRRIM | GKASFVTLQD | VGGRIQLYVA | RDDLPEGVYN | EQFKKWDLGD |
| 130 | 140 | 150 | 160 | 170 | 180 |
| ILGAKGKLFK | TKTGELSIHC | TELRLLTKAL | RPLPDKFHGL | QDQEARYRQR | YLDLISNDES |
| 190 | 200 | 210 | 220 | 230 | 240 |
| RNTFKVRSQI | LSGIRQFMVN | RGFMEVETPM | MQVIPGGAAA | RPFITHHNAL | DLDMYLRIAP |
| 250 | 260 | 270 | 280 | 290 | 300 |
| ELYLKRLVVG | GFERVFEINR | NFRNEGISVR | HNPEFTMMEL | YMAYADYKDL | IELTESLFRT |
| 310 | 320 | 330 | 340 | 350 | 360 |
| LAQDILGKTE | VTYGDVTLDF | GKPFEKLTMR | EAIKKYRPET | DMADLDNFDS | AKAIAESIGI |
| 370 | 380 | 390 | 400 | 410 | 420 |
| HVEKSWGLGR | IVTEIFEEVA | EAHLIQPTFI | TEYPAEVSPL | ARRNDVNPEI | TDRFEFFIGG |
| 430 | 440 | 450 | 460 | 470 | 480 |
| REIGNGFSEL | NDAEDQAQRF | LDQVAAKDAG | DDEAMFYDED | YVTALEHGLP | PTAGLGIGID |
| 490 | 500 | ||||
| RMVMLFTNSH | TIRDVILFPA | MRPVK |