Q64511
Gene name |
Top2b |
Protein name |
DNA topoisomerase 2-beta |
Names |
DNA topoisomerase II, beta isozyme |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:21974 |
EC number |
5.6.2.2: Enzymes altering nucleic acid conformation |
Protein Class |
|
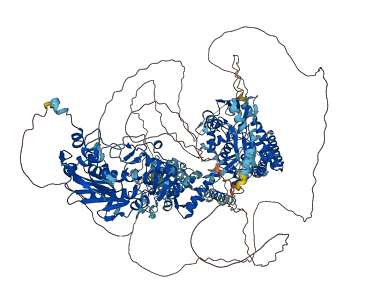
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q64511
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q64511-F1 | Predicted | AlphaFoldDB |
44 variants for Q64511
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs3404918274 | 19 | A>V | No | EVA | |
| rs231744053 | 32 | D>E | No | EVA | |
| rs3389321453 | 55 | R>L | No | EVA | |
| rs3389304272 | 64 | E>D | No | EVA | |
| rs3404918291 | 89 | G>D | No | EVA | |
| rs3389308826 | 104 | N>K | No | EVA | |
| rs3389279649 | 203 | W>C | No | EVA | |
| rs234127814 | 217 | H>Y | No | EVA | |
| rs49272973 | 252 | A>V | No | EVA | |
| rs3389304281 | 288 | L>M | No | EVA | |
| rs3389308707 | 305 | R>K | No | EVA | |
| rs3389233894 | 306 | W>* | No | EVA | |
| rs3389298712 | 326 | I>F | No | EVA | |
| rs3389289625 | 379 | N>S | No | EVA | |
| rs1132427678 | 391 | T>P | No | EVA | |
| rs1133021734 | 392 | L>M | No | EVA | |
| rs1134997830 | 396 | S>R | No | EVA | |
| rs3404534659 | 396 | S>T | No | EVA | |
| rs1131888896 | 398 | G>R | No | EVA | |
| rs1132945911 | 399 | S>Y | No | EVA | |
| rs3405061173 | 456 | A>S | No | EVA | |
| rs3389308634 | 477 | L>I | No | EVA | |
| rs3389270989 | 484 | V>L | No | EVA | |
| rs3389305399 | 494 | P>L | No | EVA | |
| rs3389312743 | 619 | I>L | No | EVA | |
| rs3389300846 | 756 | L>Q | No | EVA | |
| rs3389303452 | 766 | Y>H | No | EVA | |
| rs3389308825 | 868 | G>V | No | EVA | |
| rs3389312685 | 877 | D>V | No | EVA | |
| rs3389312690 | 888 | M>V | No | EVA | |
| rs3389232417 | 898 | L>R | No | EVA | |
| rs3389270977 | 900 | N>Y | No | EVA | |
| rs3389298683 | 925 | V>E | No | EVA | |
| rs3389298697 | 927 | R>S | No | EVA | |
| rs3389308674 | 1101 | E>K | No | EVA | |
| rs46976423 | 1168 | S>A | No | EVA | |
| rs3389308904 | 1188 | E>G | No | EVA | |
| rs3389305354 | 1191 | E>G | No | EVA | |
| rs3389305424 | 1209 | G>R | No | EVA | |
| rs3389316701 | 1262 | F>I | No | EVA | |
| rs13469722 | 1284 | P>H | No | EVA | |
| rs235426254 | 1503 | I>V | No | EVA | |
| rs3389312691 | 1550 | K>N | No | EVA | |
| rs3389232363 | 1551 | P>L | No | EVA |
No associated diseases with Q64511
5 regional properties for Q64511
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | TolB, N-terminal | 24 - 121 | IPR007195 |
| repeat | WD40-like beta propeller | 199 - 223 | IPR011659-1 |
| repeat | WD40-like beta propeller | 237 - 272 | IPR011659-2 |
| repeat | WD40-like beta propeller | 281 - 315 | IPR011659-3 |
| repeat | WD40-like beta propeller | 369 - 396 | IPR011659-4 |
Functions
| Description | ||
|---|---|---|
| EC Number | 5.6.2.2 | Enzymes altering nucleic acid conformation |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
6 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytosol | The part of the cytoplasm that does not contain organelles but which does contain other particulate matter, such as protein complexes. |
| heterochromatin | A compact and highly condensed form of chromatin that is refractory to transcription. |
| nucleolus | A small, dense body one or more of which are present in the nucleus of eukaryotic cells. It is rich in RNA and protein, is not bounded by a limiting membrane, and is not seen during mitosis. Its prime function is the transcription of the nucleolar DNA into 45S ribosomal-precursor RNA, the processing of this RNA into 5.8S, 18S, and 28S components of ribosomal RNA, and the association of these components with 5S RNA and proteins synthesized outside the nucleolus. This association results in the formation of ribonucleoprotein precursors; these pass into the cytoplasm and mature into the 40S and 60S subunits of the ribosome. |
| nucleoplasm | That part of the nuclear content other than the chromosomes or the nucleolus. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
| ribonucleoprotein complex | A macromolecular complex that contains both RNA and protein molecules. |
11 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| chromatin binding | Binding to chromatin, the network of fibers of DNA, protein, and sometimes RNA, that make up the chromosomes of the eukaryotic nucleus during interphase. |
| DNA binding | Any molecular function by which a gene product interacts selectively and non-covalently with DNA (deoxyribonucleic acid). |
| DNA topoisomerase activity | Catalysis of the transient cleavage and passage of individual DNA strands or double helices through one another, resulting a topological transformation in double-stranded DNA. |
| DNA topoisomerase type II (double strand cut, ATP-hydrolyzing) activity | Catalysis of a DNA topological transformation by transiently cleaving a pair of complementary DNA strands to form a gate through which a second double-stranded DNA segment is passed, after which the severed strands in the first DNA segment are rejoined, driven by ATP hydrolysis. The enzyme changes the linking number in multiples of 2. |
| enzyme binding | Binding to an enzyme, a protein with catalytic activity. |
| histone deacetylase binding | Binding to histone deacetylase. |
| metal ion binding | Binding to a metal ion. |
| protein C-terminus binding | Binding to a protein C-terminus, the end of a peptide chain at which the 1-carboxyl function of a constituent amino acid is not attached in peptide linkage to another amino-acid residue. |
| protein heterodimerization activity | Binding to a nonidentical protein to form a heterodimer. |
| protein kinase C binding | Binding to protein kinase C. |
8 GO annotations of biological process
| Name | Definition |
|---|---|
| axonogenesis | De novo generation of a long process of a neuron, including the terminal branched region. Refers to the morphogenesis or creation of shape or form of the developing axon, which carries efferent (outgoing) action potentials from the cell body towards target cells. |
| B cell differentiation | The process in which a precursor cell type acquires the specialized features of a B cell. A B cell is a lymphocyte of B lineage with the phenotype CD19-positive and capable of B cell mediated immunity. |
| DNA topological change | The process in which a transformation is induced in the topological structure of a double-stranded DNA helix, resulting in a change in linking number. |
| forebrain development | The process whose specific outcome is the progression of the forebrain over time, from its formation to the mature structure. The forebrain is the anterior of the three primary divisions of the developing chordate brain or the corresponding part of the adult brain (in vertebrates, includes especially the cerebral hemispheres, the thalamus, and the hypothalamus and especially in higher vertebrates is the main control center for sensory and associative information processing, visceral functions, and voluntary motor functions). |
| neuron migration | The characteristic movement of an immature neuron from germinal zones to specific positions where they will reside as they mature. |
| positive regulation of single stranded viral RNA replication via double stranded DNA intermediate | Any process that activates or increases the frequency, rate or extent of retroviral genome replication. |
| resolution of meiotic recombination intermediates | The cleavage and rejoining of intermediates, such as Holliday junctions, formed during meiotic recombination to produce two intact molecules in which genetic material has been exchanged. |
| sister chromatid segregation | The cell cycle process in which sister chromatids are organized and then physically separated and apportioned to two or more sets. |
6 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| P11388 | TOP2A | DNA topoisomerase 2-alpha | Homo sapiens (Human) | PR |
| Q02880 | TOP2B | DNA topoisomerase 2-beta | Homo sapiens (Human) | PR |
| Q01320 | Top2a | DNA topoisomerase 2-alpha | Mus musculus (Mouse) | PR |
| O46374 | TOP2A | DNA topoisomerase 2-alpha | Sus scrofa (Pig) | PR |
| P41516 | Top2a | DNA topoisomerase 2-alpha | Rattus norvegicus (Rat) | PR |
| Q23670 | top-2 | DNA topoisomerase 2 top-2 | Caenorhabditis elegans | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MAKSSLAGSD | GALTWVNNAT | KKEELETANK | NDSTKKLSVE | RVYQKKTQLE | HILLRPDTYI |
| 70 | 80 | 90 | 100 | 110 | 120 |
| GSVEPLTQLM | WVYDEDVGMN | CREVTFVPGL | YKIFDEILVN | AADNKQRDKN | MTCIKVSIDP |
| 130 | 140 | 150 | 160 | 170 | 180 |
| ESNIISIWNN | GKGIPVVEHK | VEKVYVPALI | FGQLLTSSNY | DDDEKKVTGG | RNGYGAKLCN |
| 190 | 200 | 210 | 220 | 230 | 240 |
| IFSTKFTVET | ACKEYKHSFK | QTWMNNMMKT | SEAKIKHFDG | EDYTCITFQP | DLSKFKMEKL |
| 250 | 260 | 270 | 280 | 290 | 300 |
| DKDIVALMTR | RAYDLAGSCK | GVKVMFNGKK | LPVNGFRSYV | DLYVKDKLDE | TGVALKVIHE |
| 310 | 320 | 330 | 340 | 350 | 360 |
| LANERWDVCL | TLSEKGFQQI | SFVNSIATTK | GGRHVDYVVD | QVVSKLIEVV | KKKNKAGVSV |
| 370 | 380 | 390 | 400 | 410 | 420 |
| KPFQVKNHIW | VFINCLIENP | TFDSQTKENM | TLQPKSFGSK | CQLSEKFFKA | ASNCGIVESI |
| 430 | 440 | 450 | 460 | 470 | 480 |
| LNWVKFKAQT | QLNKKCSSVK | YSKIKGIPKL | DDANDAGGKH | SLECTLILTE | GDSAKSLAVS |
| 490 | 500 | 510 | 520 | 530 | 540 |
| GLGVIGRDRY | GVFPLRGKIL | NVREASHKQI | MENAEINNII | KIVGLQYKKS | YDDAESLKTL |
| 550 | 560 | 570 | 580 | 590 | 600 |
| RYGKIMIMTD | QDQDGSHIKG | LLINFIHHNW | PSLLKHGFLE | EFITPIVKAS | KNKQELSFYS |
| 610 | 620 | 630 | 640 | 650 | 660 |
| IPEFDEWKKH | IENQKAWKIK | YYKGLGTSTA | KEAKEYFADM | ERHRILFRYA | GPEDDAAITL |
| 670 | 680 | 690 | 700 | 710 | 720 |
| AFSKKKIDDR | KEWLTNFMED | RRQRRLHGLP | EQFLYGTATK | HLTYNDFINK | ELILFSNSDN |
| 730 | 740 | 750 | 760 | 770 | 780 |
| ERSIPSLVDG | FKPGQRKVLF | TCFKRNDKRE | VKVAQLAGSV | AEMSAYHHGE | QALMMTIVNL |
| 790 | 800 | 810 | 820 | 830 | 840 |
| AQNFVGSNNI | NLLQPIGQFG | TRLHGGKDAA | SPRYIFTMLS | SLARLLFPAV | DDNLLKFLYD |
| 850 | 860 | 870 | 880 | 890 | 900 |
| DNQRVEPEWY | IPIIPMVLIN | GAEGIGTGWA | CKLPNYDARE | IVNNVRRMLE | GLDPHPMLPN |
| 910 | 920 | 930 | 940 | 950 | 960 |
| YKNFKGTIQE | LGQNQYAVSG | EIFVVDRNTV | EITELPVRTW | TQVYKEQVLE | PMLNGTDKTP |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| ALISDYKEYH | TDTTVKFVVK | MTEEKLAQAE | AAGLHKVFKL | QTTLTCNSMV | LFDHMGCLKK |
| 1030 | 1040 | 1050 | 1060 | 1070 | 1080 |
| YETVQDILKE | FFDLRLSYYG | LRKEWLVGML | GAESTKLNNQ | ARFILEKIQG | KITIENRSKK |
| 1090 | 1100 | 1110 | 1120 | 1130 | 1140 |
| DLIQMLVQRG | YESDPVKAWK | EAQEKAAEEE | DSQNQHDDSS | SDSGTPSGPD | FNYILNMSLW |
| 1150 | 1160 | 1170 | 1180 | 1190 | 1200 |
| SLTKEKVEEL | IKQRDTKGRE | VNDLKRKSPS | DLWKEDLAAF | VEELDKVEAQ | EREDILAGMS |
| 1210 | 1220 | 1230 | 1240 | 1250 | 1260 |
| GKAIKGKVGK | PKVKKLQLEE | TMPSPYGRRI | VPEITAMKAD | ASRKLLKKKK | GDPDTTVVKV |
| 1270 | 1280 | 1290 | 1300 | 1310 | 1320 |
| EFDEEFSGTP | AEGTGEETLT | PSAPVNKGPK | PKREKKEPGT | RVRKTPTSTG | KTNAKKVKKR |
| 1330 | 1340 | 1350 | 1360 | 1370 | 1380 |
| NPWSDDESKS | ESDLEEAEPV | VIPRDSLLRR | AAAERPKYTF | DFSEEEDDDA | AAADDSNDLE |
| 1390 | 1400 | 1410 | 1420 | 1430 | 1440 |
| ELKVKASPIT | NDGEDEFVPS | DGLDKDEYAF | SSGKSKATPE | KSSNDKKSQD | FGNLFSFPSY |
| 1450 | 1460 | 1470 | 1480 | 1490 | 1500 |
| SQKSEDDSAK | FDSNEEDTAS | VFAPSFGLKQ | TDKLPSKTVA | AKKGKPPSDT | APKAKRAPKQ |
| 1510 | 1520 | 1530 | 1540 | 1550 | 1560 |
| KKIVETINSD | SDSEFGIPKK | TTTPKGKGRG | AKKRKASGSE | NEGDYNPGRK | PSKTASKKPK |
| 1570 | 1580 | 1590 | 1600 | 1610 | |
| KTSFDQDSDV | DIFPSDFTSE | PPALPRTGRA | RKEVKYFAES | DEEEDVDFAM | FN |