Q5JLP4
Gene name |
CKX4 (Os01g0940000, LOC_Os01g71310, B1150F11.25) |
Protein name |
Cytokinin dehydrogenase 4 |
Names |
Cytokinin oxidase 4, OsCKX4 |
Species |
Oryza sativa subsp japonica (Rice) |
KEGG Pathway |
osa:4326515 |
EC number |
1.5.99.12: With other acceptors |
Protein Class |
|
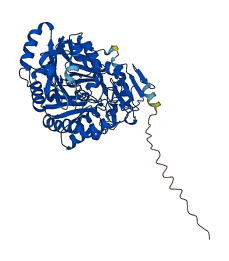
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q5JLP4
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q5JLP4-F1 | Predicted | AlphaFoldDB |
No variants for Q5JLP4
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q5JLP4 | |||||
No associated diseases with Q5JLP4
10 regional properties for Q5JLP4
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | UVR domain | 458 - 492 | IPR001943 |
| domain | AAA+ ATPase domain | 241 - 381 | IPR003593-1 |
| domain | AAA+ ATPase domain | 583 - 725 | IPR003593-2 |
| domain | ATPase, AAA-type, core | 246 - 362 | IPR003959-1 |
| domain | ATPase, AAA-type, core | 582 - 755 | IPR003959-2 |
| domain | Clp, repeat (R) domain | 42 - 184 | IPR004176 |
| conserved_site | ClpA/B, conserved site 1 | 336 - 348 | IPR018368 |
| domain | Clp ATPase, C-terminal | 762 - 852 | IPR019489 |
| conserved_site | ClpA/B, conserved site 2 | 617 - 635 | IPR028299 |
| domain | ClpA/ClpB, AAA lid domain | 384 - 482 | IPR041546 |
Functions
| Description | ||
|---|---|---|
| EC Number | 1.5.99.12 | With other acceptors |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| extracellular space | That part of a multicellular organism outside the cells proper, usually taken to be outside the plasma membranes, and occupied by fluid. |
3 GO annotations of molecular function
| Name | Definition |
|---|---|
| cytokinin dehydrogenase activity | Catalysis of the reaction: N6-dimethylallyladenine + acceptor + H2O = adenine + 3-methylbut-2-enal + reduced electron acceptor. |
| FAD binding | Binding to the oxidized form, FAD, of flavin-adenine dinucleotide, the coenzyme or the prosthetic group of various flavoprotein oxidoreductase enzymes. |
| oxidoreductase activity | Catalysis of an oxidation-reduction (redox) reaction, a reversible chemical reaction in which the oxidation state of an atom or atoms within a molecule is altered. One substrate acts as a hydrogen or electron donor and becomes oxidized, while the other acts as hydrogen or electron acceptor and becomes reduced. |
1 GO annotations of biological process
| Name | Definition |
|---|---|
| cytokinin metabolic process | The chemical reactions and pathways involving cytokinins, a class of adenine-derived compounds that can function in plants as growth regulators. |
8 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| A3AVP1 | CKX8 | Cytokinin dehydrogenase 8 | Oryza sativa subsp japonica (Rice) | PR |
| Q6YW51 | CKX6 | Cytokinin dehydrogenase 6 | Oryza sativa subsp japonica (Rice) | PR |
| Q8LNV6 | CKX3 | Cytokinin dehydrogenase 3 | Oryza sativa subsp japonica (Rice) | PR |
| Q6YW50 | CKX7 | Cytokinin dehydrogenase 7 | Oryza sativa subsp japonica (Rice) | PR |
| Q9FUJ2 | CKX4 | Cytokinin dehydrogenase 4 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q94AX4 | DLD | D-lactate dehydrogenase [cytochrome], mitochondrial | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q9LTS3 | CKX3 | Cytokinin dehydrogenase 3 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q9LY71 | CKX6 | Cytokinin dehydrogenase 6 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MRGAMKPSIV | HCLKLLMLLA | LGGVTMHVPD | EDDVVASLGA | LRLDGHFSFD | DAHAAARDFG |
| 70 | 80 | 90 | 100 | 110 | 120 |
| NRCSLLPAAV | LHPGSVSDVA | ATVRRVFQLG | RSSPLTVAAR | GHGHSLLGQS | QAAGGIVVKM |
| 130 | 140 | 150 | 160 | 170 | 180 |
| ESLAAAAARA | VRVHGGASPH | VDAPGGELWI | NVLHETLKHG | LAPRSWTDYL | HLTVGGTLSN |
| 190 | 200 | 210 | 220 | 230 | 240 |
| AGVSGQAFRH | GPQVSNVNQL | EIVTGRGEVV | TCSHEVNSDL | FYAALGGLGQ | FGIITRARIA |
| 250 | 260 | 270 | 280 | 290 | 300 |
| LEPAPKMVRW | IRVLYSDFET | FTEDQEKLIA | SEKTFDYIEG | FVIINRTGIL | NNWRTSFKPQ |
| 310 | 320 | 330 | 340 | 350 | 360 |
| DPVQASQFQS | DGRVLYCLEL | TMNFNHDEAD | IMEQEVGALL | SRLRYISSTL | FYTDVTYLEF |
| 370 | 380 | 390 | 400 | 410 | 420 |
| LDRVHTSELK | LRAQGLWEVP | HPWLNLLIPR | STVHKFAKEV | FGKILKDSNN | GPILLYPVNR |
| 430 | 440 | 450 | 460 | 470 | 480 |
| TKWDNRTSVV | IPDEEIFYLV | GFLSSAPSSS | GHGSVEHAMN | LNNKIVDFCE | KNGVGMKQYL |
| 490 | 500 | 510 | 520 | ||
| APYTTQKQWK | AHFGARWETF | ERRKHTYDPL | AILAPGQRIF | PKASLPMSL |