Q8MNV7
Gene name |
smrc-1 |
Protein name |
SWI/SNF-related matrix-associated actin-dependent regulator of chromatin subfamily A-like protein 1 homolog |
Names |
|
Species |
Caenorhabditis elegans |
KEGG Pathway |
cel:CELE_C16A3.1 |
EC number |
|
Protein Class |
|
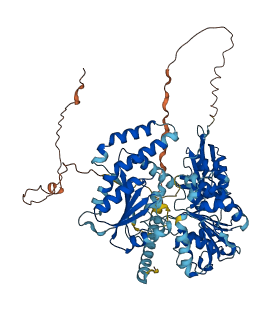
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q8MNV7
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q8MNV7-F1 | Predicted | AlphaFoldDB |
No variants for Q8MNV7
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q8MNV7 | |||||
No associated diseases with Q8MNV7
4 regional properties for Q8MNV7
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Signal transduction response regulator, receiver domain | 715 - 833 | IPR001789 |
| domain | GAF domain | 269 - 423 | IPR003018 |
| domain | Signal transduction histidine kinase, dimerisation/phosphoacceptor domain | 447 - 514 | IPR003661 |
| domain | Histidine kinase domain | 456 - 690 | IPR005467 |
2 GO annotations of cellular component
| Name | Definition |
|---|---|
| nuclear replication fork | The Y-shaped region of a nuclear replicating DNA molecule, resulting from the separation of the DNA strands and in which the synthesis of new strands takes place. Also includes associated protein complexes. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP-dependent chromatin remodeler activity | An activity, driven by ATP hydrolysis, that modulates the contacts between histones and DNA, resulting in a change in chromosome architecture within the nucleosomal array, leading to chromatin remodeling. |
| ATP-dependent DNA/DNA annealing activity | An ATP-dependent activity that facilitates the formation of a complementary double-stranded DNA molecule. |
| helicase activity | Catalysis of the reaction: ATP + H2O = ADP + phosphate, to drive the unwinding of a DNA or RNA helix. |
| hydrolase activity | Catalysis of the hydrolysis of various bonds, e.g. C-O, C-N, C-C, phosphoric anhydride bonds, etc. |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| DNA repair | The process of restoring DNA after damage. Genomes are subject to damage by chemical and physical agents in the environment (e.g. UV and ionizing radiations, chemical mutagens, fungal and bacterial toxins, etc.) and by free radicals or alkylating agents endogenously generated in metabolism. DNA is also damaged because of errors during its replication. A variety of different DNA repair pathways have been reported that include direct reversal, base excision repair, nucleotide excision repair, photoreactivation, bypass, double-strand break repair pathway, and mismatch repair pathway. |
| regulation of transcription by RNA polymerase II | Any process that modulates the frequency, rate or extent of transcription mediated by RNA polymerase II. |
| replication fork processing | The process in which a DNA replication fork that has stalled is restored to a functional state and replication is restarted. The stalling may be due to DNA damage, DNA secondary structure, bound proteins, dNTP shortage, or other causes. |
| replication fork protection | Any process that prevents the collapse of stalled replication forks. |
6 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| Q9TTA5 | SMARCAL1 | SWI/SNF-related matrix-associated actin-dependent regulator of chromatin subfamily A-like protein 1 | Bos taurus (Bovine) | PR |
| Q5FWF4 | ZRANB3 | DNA annealing helicase and endonuclease ZRANB3 | Homo sapiens (Human) | PR |
| Q9NZC9 | SMARCAL1 | SWI/SNF-related matrix-associated actin-dependent regulator of chromatin subfamily A-like protein 1 | Homo sapiens (Human) | PR |
| Q8BJL0 | Smarcal1 | SWI/SNF-related matrix-associated actin-dependent regulator of chromatin subfamily A-like protein 1 | Mus musculus (Mouse) | PR |
| B4F769 | Smarcal1 | SWI/SNF-related matrix-associated actin-dependent regulator of chromatin subfamily A-like protein 1 | Rattus norvegicus (Rat) | PR |
| B2ZFP3 | smarcal1 | SWI/SNF-related matrix-associated actin-dependent regulator of chromatin subfamily A-like protein 1 | Danio rerio (Zebrafish) (Brachydanio rerio) | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MVLTDEQRQA | IAKKREEAIR | RAAAYREREM | QAAANATAST | SSAAPPAPPK | PVIPVMFSQN |
| 70 | 80 | 90 | 100 | 110 | 120 |
| RQNFQPMKPT | MNNSTKQSTI | NNYIKQVQKP | EPTSLIKPTI | GVKLKLDIGD | RIKIEFYPFH |
| 130 | 140 | 150 | 160 | 170 | 180 |
| SAVIDLIKQV | PSRNYDPAKR | SWTVASSDHI | TISNILKNAT | AVKVELEPLP | QNIIGLTNFK |
| 190 | 200 | 210 | 220 | 230 | 240 |
| PKAAPSDLNT | VMDPSLIERL | FPYQKEGVIF | ALERDGRILL | ADEMGLGKSV | QALTIARYYK |
| 250 | 260 | 270 | 280 | 290 | 300 |
| ADWPLLIVCP | ASVKGAWKKQ | LNTFFPIIHR | IFIVDKSSDP | LPDVCTSNTV | AIMSYEQMVL |
| 310 | 320 | 330 | 340 | 350 | 360 |
| KHDILKKEKY | RTIIFDESHM | LKDGKARRTK | VATDLSKVAL | HVILLSGTPA | LSRPSELFTQ |
| 370 | 380 | 390 | 400 | 410 | 420 |
| IRLIDHKLFT | NFHEFAIRYC | DGKQGRFCFE | AKGCTNSEEL | AAIMFKRLMI | RRLKADVLKD |
| 430 | 440 | 450 | 460 | 470 | 480 |
| LPEKRREVVY | VSGPTIDARM | DDLQKARADY | EKVNSMERKH | ESLLEFYSLT | GIVKAAAVCE |
| 490 | 500 | 510 | 520 | 530 | 540 |
| HILENYFYPD | APPRKVLIFA | HHQIVLDTIQ | VEVNKRKLGS | IRIDGKTPSH | RRTALCDSFQ |
| 550 | 560 | 570 | 580 | 590 | 600 |
| TDDNIRVAVL | SITAAGVGIT | LTAASVVVFA | EIHFNPGYLV | QAEDRAHRVG | QKDSVFVQYL |
| 610 | 620 | 630 | 640 | 650 | 660 |
| IAKKTADDVM | WNMVQQKLDV | LGQVSLSSDT | FRTADKMHLR | FNDAAQPGIA | EYLKKTPDTT |
| 670 | 680 | ||||
| IDEWEDPVEE | KEDDDLEIIC | DSPAPKRIKN |