Q80YQ2
Gene name |
Med23 (Crsp3, Kiaa1216, Sur2) |
Protein name |
Mediator of RNA polymerase II transcription subunit 23 |
Names |
Cofactor required for Sp1 transcriptional activation subunit 3, CRSP complex subunit 3, Mediator complex subunit 23, Protein sur-2 homolog, mSur-2 |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:70208 |
EC number |
|
Protein Class |
|
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
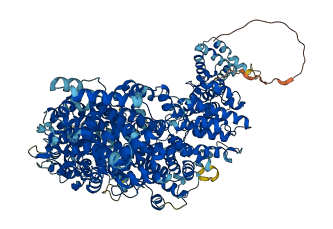
2 structures for Q80YQ2
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| 6W1S | EM | 402 A | R | 1-1367 | PDB |
| AF-Q80YQ2-F1 | Predicted | AlphaFoldDB |
57 variants for Q80YQ2
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs3400416885 | 33 | E>S | No | EVA | |
| rs3400976742 | 37 | L>I | No | EVA | |
| rs3389103027 | 98 | C>Y | No | EVA | |
| rs51990989 | 105 | D>A | No | EVA | |
| rs3389067557 | 108 | E>K | No | EVA | |
| rs3389094199 | 112 | T>R | No | EVA | |
| rs3389102481 | 125 | I>V | No | EVA | |
| rs3389080473 | 130 | D>V | No | EVA | |
| rs3389102470 | 144 | K>E | No | EVA | |
| rs3389060612 | 162 | A>T | No | EVA | |
| rs3389094203 | 228 | L>P | No | EVA | |
| rs3389090158 | 229 | P>A | No | EVA | |
| rs3389093208 | 246 | A>T | No | EVA | |
| rs3389102472 | 248 | L>M | No | EVA | |
| rs3389080508 | 254 | G>D | No | EVA | |
| rs3389097684 | 259 | D>V | No | EVA | |
| rs3389060601 | 312 | M>T | No | EVA | |
| rs3389060673 | 328 | Q>* | No | EVA | |
| rs3389093026 | 353 | V>A | No | EVA | |
| rs3389090162 | 386 | K>N | No | EVA | |
| rs3389084793 | 396 | M>L | No | EVA | |
| rs3389037129 | 442 | T>M | No | EVA | |
| rs3389103040 | 512 | T>M | No | EVA | |
| rs3401080296 | 532 | T>M | No | EVA | |
| rs3389093050 | 572 | V>L | No | EVA | |
| rs3389067632 | 608 | F>I | No | EVA | |
| rs3389102455 | 649 | A>V | No | EVA | |
| rs3389093036 | 662 | Q>K | No | EVA | |
| rs3389097710 | 737 | A>S | No | EVA | |
| rs3400978924 | 810 | V>A | No | EVA | |
| rs3400632681 | 818 | A>T | No | EVA | |
| rs3389060695 | 875 | E>* | No | EVA | |
| rs3389084870 | 883 | Y>H | No | EVA | |
| rs3389094195 | 899 | R>Q | No | EVA | |
| rs3389067626 | 902 | D>E | No | EVA | |
| rs3389037191 | 918 | H>R | No | EVA | |
| rs3389097716 | 919 | T>S | No | EVA | |
| rs3389097680 | 933 | Y>F | No | EVA | |
| rs3389097651 | 953 | P>H | No | EVA | |
| rs3389084807 | 954 | I>T | No | EVA | |
| rs3389037110 | 1009 | L>M | No | EVA | |
| rs3389093101 | 1021 | H>L | No | EVA | |
| rs3389102503 | 1043 | C>Y | No | EVA | |
| rs3389037171 | 1046 | D>Y | No | EVA | |
| rs3389103018 | 1059 | N>K | No | EVA | |
| rs3389094239 | 1076 | V>L | No | EVA | |
| rs3389093073 | 1081 | G>A | No | EVA | |
| rs49883787 | 1083 | S>C | No | EVA | |
| rs248216484 | 1130 | V>I | No | EVA | |
| rs3389060643 | 1175 | S>F | No | EVA | |
| rs3389093348 | 1211 | L>I | No | EVA | |
| rs3389060677 | 1226 | L>I | No | EVA | |
| rs50396942 | 1242 | E>Q | No | EVA | |
| rs3389090187 | 1299 | Y>* | No | EVA | |
| rs3389067630 | 1307 | G>D | No | EVA | |
| rs3389097711 | 1353 | A>V | No | EVA | |
| rs47512542 | 1361 | A>P | No | EVA |
No associated diseases with Q80YQ2
No regional properties for Q80YQ2
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| No domain, repeats, and functional sites for Q80YQ2 | |||
6 GO annotations of cellular component
| Name | Definition |
|---|---|
| core mediator complex | A protein complex that interacts with the carboxy-terminal domain of the largest subunit of RNA polymerase II and plays an active role in transducing the signal from a transcription factor to the transcriptional machinery. The core mediator complex has a stimulatory effect on basal transcription, and contains most of the same subdomains as the larger form of mediator complex -- a head domain comprising proteins known in Saccharomyces as Srb2, -4, and -5, Med6, -8, and -11, and Rox3 proteins; a middle domain comprising Med1, -4, and -7, Nut1 and -2, Cse2, Rgr1, Soh1, and Srb7 proteins; and a tail consisting of Gal11p, Med2p, Pgd1p, and Sin4p -- but lacks the regulatory subcomplex comprising Ssn2, -3, and -8, and Srb8 proteins. Metazoan core mediator complexes have similar modular structures and include homologs of yeast Srb and Med proteins. |
| mediator complex | A protein complex that interacts with the carboxy-terminal domain of the largest subunit of RNA polymerase II and plays an active role in transducing the signal from a transcription factor to the transcriptional machinery. The mediator complex is required for activation of transcription of most protein-coding genes, but can also act as a transcriptional corepressor. The Saccharomyces complex contains several identifiable subcomplexes: a head domain comprising Srb2, -4, and -5, Med6, -8, and -11, and Rox3 proteins; a middle domain comprising Med1, -4, and -7, Nut1 and -2, Cse2, Rgr1, Soh1, and Srb7 proteins; a tail consisting of Gal11p, Med2p, Pgd1p, and Sin4p; and a regulatory subcomplex comprising Ssn2, -3, and -8, and Srb8 proteins. Metazoan mediator complexes have similar modular structures and include homologs of yeast Srb and Med proteins. |
| nucleoplasm | That part of the nuclear content other than the chromosomes or the nucleolus. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
| transcription regulator complex | A protein complex that is capable of associating with DNA by direct binding, or via other DNA-binding proteins or complexes, and regulating transcription. |
| ubiquitin ligase complex | A protein complex that includes a ubiquitin-protein ligase and enables ubiquitin protein ligase activity. The complex also contains other proteins that may confer substrate specificity on the complex. |
1 GO annotations of molecular function
| Name | Definition |
|---|---|
| ubiquitin protein ligase activity | Catalysis of the transfer of ubiquitin to a substrate protein via the reaction X-ubiquitin + S -> X + S-ubiquitin, where X is either an E2 or E3 enzyme, the X-ubiquitin linkage is a thioester bond, and the S-ubiquitin linkage is an amide bond: an isopeptide bond between the C-terminal glycine of ubiquitin and the epsilon-amino group of lysine residues in the substrate or, in the linear extension of ubiquitin chains, a peptide bond the between the C-terminal glycine and N-terminal methionine of ubiquitin residues. |
8 GO annotations of biological process
| Name | Definition |
|---|---|
| positive regulation of gene expression | Any process that increases the frequency, rate or extent of gene expression. Gene expression is the process in which a gene's coding sequence is converted into a mature gene product (protein or RNA). |
| positive regulation of T cell extravasation | Any process that activates or increases the frequency, rate or extent of T cell extravasation. |
| positive regulation of transcription elongation by RNA polymerase II | Any process that activates or increases the frequency, rate or extent of transcription elongation, the extension of an RNA molecule after transcription initiation and promoter clearance by the addition of ribonucleotides, catalyzed by RNA polymerase II. |
| positive regulation of transcription initiation by RNA polymerase II | Any process that increases the rate, frequency or extent of a process involved in starting transcription from an RNA polymerase II promoter. |
| protein ubiquitination | The process in which one or more ubiquitin groups are added to a protein. |
| regulation of DNA-templated transcription | Any process that modulates the frequency, rate or extent of cellular DNA-templated transcription. |
| regulation of transcription by RNA polymerase II | Any process that modulates the frequency, rate or extent of transcription mediated by RNA polymerase II. |
| RNA polymerase II preinitiation complex assembly | The aggregation, arrangement and bonding together of proteins on an RNA polymerase II promoter DNA to form the transcriptional preinitiation complex (PIC), the formation of which is a prerequisite for transcription by RNA polymerase. |
4 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| Q9W1X7 | MED23 | Mediator of RNA polymerase II transcription subunit 23 | Drosophila melanogaster (Fruit fly) | PR |
| Q9ULK4 | MED23 | Mediator of RNA polymerase II transcription subunit 23 | Homo sapiens (Human) | PR |
| Q5EB59 | Med23 | Mediator of RNA polymerase II transcription subunit 23 | Rattus norvegicus (Rat) | PR |
| Q10669 | sur-2 | Mediator of RNA polymerase II transcription subunit 23 | Caenorhabditis elegans | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| METQLQSIFE | EVVKTEIIEE | AFPGMFMDTP | EDEKTKLISC | LAAFRQFWSG | LSQESHEQCV |
| 70 | 80 | 90 | 100 | 110 | 120 |
| QWIVKFIHGQ | HSPKRISFLY | DCLAMAVETG | LLPPRMVCES | LINSDSLEWE | RTQLWALTFK |
| 130 | 140 | 150 | 160 | 170 | 180 |
| LVRKIIGGVD | YKGVRDLLKA | ILEKILTIPN | TVSSAVVQQL | LAAREVIAYI | LERNACLLPA |
| 190 | 200 | 210 | 220 | 230 | 240 |
| YFAVTEIRKL | YPEGKLPHWL | LGNLVSDFVD | TFRPTARINS | ICGRCSLLPV | VNNSGAICNS |
| 250 | 260 | 270 | 280 | 290 | 300 |
| WKLDPATLRF | PLKGLLPYDK | DLFEPQTALL | RYVLEQPYSR | DMVCNMLGLN | KQHKQRCPVL |
| 310 | 320 | 330 | 340 | 350 | 360 |
| EDQLVDLVVY | AMERSETEEK | FDDGGTSQLL | WQHLSSQLIF | FVLFQFASFP | HMVLSLHQKL |
| 370 | 380 | 390 | 400 | 410 | 420 |
| AGRGLIKGRD | HLMWVLLQFI | SGSIQKNALA | DFLPVMKLFD | LLYPEKECIP | VPDINKPQST |
| 430 | 440 | 450 | 460 | 470 | 480 |
| HAFAMTCIWI | HLNRKAQNGD | STLQIPIPHS | LKLHHEFLQQ | SLRNKSLQMN | DYKIALLCNA |
| 490 | 500 | 510 | 520 | 530 | 540 |
| YSTNSECFTL | PMGALVETIY | GNGIMRVPLP | GTSCLASASV | TPLPMNLLDS | LTVHAKMSLI |
| 550 | 560 | 570 | 580 | 590 | 600 |
| HSIATRVIKL | AHTKSSVALA | PALVETYSRL | LVYMEIESLG | IKGFISQLLP | TVFKSHAWGI |
| 610 | 620 | 630 | 640 | 650 | 660 |
| LHTLLEMFSH | RMHHIQPHYR | VQLLSHLHTL | AAVAQTNQNQ | LHLCVESTAL | RLITALGSSE |
| 670 | 680 | 690 | 700 | 710 | 720 |
| VQPQFTRFLN | DPKTVLSAES | EELNRALILT | LARATHVTDF | FTGSDSIQGT | WCKDILQTIM |
| 730 | 740 | 750 | 760 | 770 | 780 |
| NFTPHNWASH | TLSCFPAPLQ | AFFKQNNVPQ | ESRFNLKKNV | EEEYRKWKSM | TDENEIITQF |
| 790 | 800 | 810 | 820 | 830 | 840 |
| SVQGFPPLFL | CLLWKMLLET | DHISQIGYKV | LERIGARALV | AHVRTFADFL | VYEFSTSAGG |
| 850 | 860 | 870 | 880 | 890 | 900 |
| QQLNKCIEIL | NDMVWKYNIV | TLDRLILCLA | MRSHEGNEAQ | VCYFIIQLLL | LKPNDFRNRV |
| 910 | 920 | 930 | 940 | 950 | 960 |
| SDFVKENSPE | HWLQSDWHTK | HMSYHKKYPE | KLYFEGLAEQ | VDPPVPIQSP | YLPIYFGNVC |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| LRFLPVFDIV | IHRFLELLPV | SKSLETLLDH | LGGLYKFHDR | PVTYLYNTLH | YYEMCLRNRD |
| 1030 | 1040 | 1050 | 1060 | 1070 | 1080 |
| HLKRKLVHAI | IGSLKDNRPQ | GWCLSDTYLK | HAMNAREDNP | WVPEDSYYCK | LIGRLVDTMA |
| 1090 | 1100 | 1110 | 1120 | 1130 | 1140 |
| GKSPGPFPNC | DWRFNEFPNP | AAHALHVTCV | ELMALAVPGK | DVGNALLNVV | LKSQPLVPRE |
| 1150 | 1160 | 1170 | 1180 | 1190 | 1200 |
| NITAWMNAIG | LIITALPEPY | WIVLHDRIVN | VISSSSLTSE | TEWVGYPFRL | FDFTACHQSY |
| 1210 | 1220 | 1230 | 1240 | 1250 | 1260 |
| SEMSCSYTLA | LAHAVWHHSS | IGQLSLIPKF | LTEALLPVVK | TEFQLLYVYH | LVGPFLQRFQ |
| 1270 | 1280 | 1290 | 1300 | 1310 | 1320 |
| QERTRCMIEI | GVAFYDMLLN | VDQCSTHLNY | MDPICDFLYH | MKYMFTGDSV | KEQVEKIICN |
| 1330 | 1340 | 1350 | 1360 | ||
| LKPALKLRLR | FITHISKMEP | AVPPQALNSG | SPAPQSNQVP | ASLPVTQ |