Q5NCE8
Gene name |
Mrs2 (Gm902, Mrs2l) |
Protein name |
Magnesium transporter MRS2 homolog, mitochondrial |
Names |
MRS2-like protein |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:380836 |
EC number |
|
Protein Class |
|
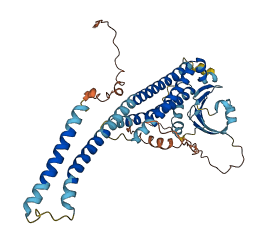
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q5NCE8
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q5NCE8-F1 | Predicted | AlphaFoldDB |
21 variants for Q5NCE8
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs226446155 | 42 | S>Y | No | EVA | |
| rs244367321 | 48 | S>* | No | EVA | |
| rs3389290745 | 88 | V>A | No | EVA | |
| rs46423077 | 106 | A>P | No | EVA | |
| rs3389204796 | 115 | M>K | No | EVA | |
| rs3389271835 | 144 | D>V | No | EVA | |
| rs3404157102 | 162 | L>P | No | EVA | |
| rs3403755921 | 180 | I>V | No | EVA | |
| rs215039156 | 194 | R>K | No | EVA | |
| rs255339834 | 197 | V>I | No | EVA | |
| rs3403963809 | 223 | H>Y | No | EVA | |
| rs3389271866 | 320 | D>Y | No | EVA | |
| rs3389290838 | 331 | L>H | No | EVA | |
| rs3389275319 | 348 | V>D | No | EVA | |
| rs3389283661 | 350 | F>S | No | EVA | |
| rs3389274902 | 357 | S>Y | No | EVA | |
| rs3389275337 | 373 | F>* | No | EVA | |
| rs3389270327 | 383 | L>M | No | EVA | |
| rs29971816 | 400 | T>A | No | EVA | |
| rs3412778551 | 405 | K>R | No | EVA | |
| rs29971033 | 410 | N>D | No | EVA |
No associated diseases with Q5NCE8
No regional properties for Q5NCE8
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| No domain, repeats, and functional sites for Q5NCE8 | |||
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| integral component of membrane | The component of a membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
| mitochondrial inner membrane | The inner, i.e. lumen-facing, lipid bilayer of the mitochondrial envelope. It is highly folded to form cristae. |
| mitochondrion | A semiautonomous, self replicating organelle that occurs in varying numbers, shapes, and sizes in the cytoplasm of virtually all eukaryotic cells. It is notably the site of tissue respiration. |
1 GO annotations of molecular function
| Name | Definition |
|---|---|
| magnesium ion transmembrane transporter activity | Enables the transfer of magnesium (Mg) ions from one side of a membrane to the other. |
3 GO annotations of biological process
| Name | Definition |
|---|---|
| lactate metabolic process | The chemical reactions and pathways involving lactate, the anion of lactic acid. |
| magnesium ion transport | The directed movement of magnesium (Mg) ions into, out of or within a cell, or between cells, by means of some agent such as a transporter or pore. |
| mitochondrial magnesium ion transmembrane transport | The process in which a magnesium ion (Mg2+) is transported across a mitochondrial membrane, into or out of the mitochondrion. |
6 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| Q9HD23 | MRS2 | Magnesium transporter MRS2 homolog, mitochondrial | Homo sapiens (Human) | PR |
| Q9ET09 | Mrs2 | Magnesium transporter MRS2 homolog, mitochondrial | Rattus norvegicus (Rat) | PR |
| Q10S25 | MRS2-H | Putative magnesium transporter MRS2-H | Oryza sativa subsp japonica (Rice) | PR |
| Q9AUK4 | MRS2-A | Magnesium transporter MRS2-A, chloroplastic | Oryza sativa subsp japonica (Rice) | PR |
| Q304A0 | MRS2-7 | Magnesium transporter MRS2-7 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| Q9FLG2 | MRS2-2 | Magnesium transporter MRS2-2 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MECLRCLPGL | LPRAAQPRRA | LWTAVARLSL | AACGGRATPL | RSRSPKASST | ARAAGDVLRF |
| 70 | 80 | 90 | 100 | 110 | 120 |
| RTSDASQATL | ASVAQVFAVT | KFDKEGNVTS | FERKKTELYH | ELALQARDLR | FQHVMSITTR |
| 130 | 140 | 150 | 160 | 170 | 180 |
| NNRIIMRMEY | LKAVITPECL | LILDYRNLNL | EHWLFRELPS | QLAGEGQLVT | YPLPFEFRAI |
| 190 | 200 | 210 | 220 | 230 | 240 |
| EALLQYWIST | LRGRLSVLQP | LILETLDALV | DPKHSSVDRS | KLHVLLQNGK | SLSELETDIK |
| 250 | 260 | 270 | 280 | 290 | 300 |
| IFKESILELL | DEEEMLEELC | LTKWSDPHVF | EKSSTGIDHA | EEMELLLENY | YRLAEDLSNE |
| 310 | 320 | 330 | 340 | 350 | 360 |
| ARELRVLIDD | SQSIIFINLD | SHRNVMMRLN | LQLTMGTFSL | SLFGLMGVAF | GMNLESSLEE |
| 370 | 380 | 390 | 400 | 410 | 420 |
| DHRVFWLVTG | IMFMGSGLIW | RRLLSFLGRQ | LEAPVPPVMT | SLPKKTLLAN | RRMDVKNSLR |
| 430 | |||||
| PEGLGASRTI | LASR |