Q9V3D6
Gene name |
Cpsf100 (CG1957) |
Protein name |
Probable cleavage and polyadenylation specificity factor subunit 2 |
Names |
Cleavage and polyadenylation specificity factor 100 kDa subunit, CPSF 100 kDa subunit |
Species |
Drosophila melanogaster (Fruit fly) |
KEGG Pathway |
dme:Dmel_CG1957 |
EC number |
|
Protein Class |
|
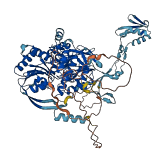
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q9V3D6
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q9V3D6-F1 | Predicted | AlphaFoldDB |
No variants for Q9V3D6
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q9V3D6 | |||||
No associated diseases with Q9V3D6
6 regional properties for Q9V3D6
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Metallo-beta-lactamase | 17 - 223 | IPR001279 |
| domain | Zn-dependent metallo-hydrolase, RNA specificity domain | 539 - 600 | IPR011108 |
| domain | Beta-Casp domain | 243 - 369 | IPR022712 |
| domain | Cleavage and polyadenylation specificity factor 2, C-terminal | 617 - 655 | IPR025069-1 |
| domain | Cleavage and polyadenylation specificity factor 2, C-terminal | 660 - 753 | IPR025069-2 |
| domain | CPSF2, metallo-hydrolase domain | 7 - 204 | IPR035639 |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| mRNA cleavage and polyadenylation specificity factor complex | A multisubunit complex that binds to the canonical AAUAAA hexamer and to U-rich upstream sequence elements on the pre-mRNA, thereby stimulating the otherwise weakly active and nonspecific polymerase to elongate efficiently RNAs containing a poly(A) signal. |
1 GO annotations of molecular function
| Name | Definition |
|---|---|
| RNA binding | Binding to an RNA molecule or a portion thereof. |
3 GO annotations of biological process
| Name | Definition |
|---|---|
| mRNA 3'-end processing by stem-loop binding and cleavage | Any mRNA 3'-end processing that involves the binding to and cleavage of a stem-loop structure. For example, histone mRNAs contain a highly conserved stem-loop sequence at the 3' end of the mRNA with a 6 base pairs (bp) stem and a 4-nt loop. The mRNA is cleaved between these two elements, after the fourth or fifth nucleotide, which is typically an adenosine. |
| mRNA polyadenylation | The enzymatic addition of a sequence of 40-200 adenylyl residues at the 3' end of a eukaryotic mRNA primary transcript. |
| pre-mRNA cleavage required for polyadenylation | The targeted, endonucleolytic cleavage of a pre-mRNA, required for polyadenylation of the 3' end. This cleavage is directed by binding sites near the 3' end of the mRNA and leaves a 3' hydoxyl end which then becomes a target for adenylation. |
4 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| Q12102 | CFT2 | Cleavage factor two protein 2 | Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) | PR |
| Q9P2I0 | CPSF2 | Cleavage and polyadenylation specificity factor subunit 2 | Homo sapiens (Human) | PR |
| O35218 | Cpsf2 | Cleavage and polyadenylation specificity factor subunit 2 | Mus musculus (Mouse) | PR |
| O17403 | cpsf-2 | Probable cleavage and polyadenylation specificity factor subunit 2 | Caenorhabditis elegans | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MTSIIKLHTI | SGAMDESPPC | YILQIDDVRI | LLDCGWDEKF | DANFIKELKR | QVHTLDAVLL |
| 70 | 80 | 90 | 100 | 110 | 120 |
| SHPDAYHLGA | LPYLVGKLGL | NCPIYATIPV | FKMGQMFMYD | LYMSHFNMGD | FDLFSLDDVD |
| 130 | 140 | 150 | 160 | 170 | 180 |
| TAFEKITQLK | YNQTVSLKDK | GYGISITPLN | AGHMIGGTIW | KIVKVGEEDI | VYATDFNHKK |
| 190 | 200 | 210 | 220 | 230 | 240 |
| ERHLSGCELD | RLQRPSLLIT | DAYNAQYQQA | RRRARDEKLM | TNILQTVRNN | GNVLIAVDTA |
| 250 | 260 | 270 | 280 | 290 | 300 |
| GRVLELAHML | DQLWKNKESG | LMAYSLALLN | NVSYNVIEFA | KSQIEWMSDK | LTKAFEGARN |
| 310 | 320 | 330 | 340 | 350 | 360 |
| NPFQFKHIQL | CHSLADVYKL | PAGPKVVLAS | TPDLESGFTR | DLFVQWASNA | NNSIILTTRT |
| 370 | 380 | 390 | 400 | 410 | 420 |
| SPGTLAMELV | ENCAPGKQIE | LDVRRRVDLE | GAELEEYLRT | QGEKLNPLIV | KPDVEEESSS |
| 430 | 440 | 450 | 460 | 470 | 480 |
| ESEDDIEMSV | ITGKHDIVVR | PEGRHHSGFF | KSNKRHHVMF | PYHEEKVKCD | EYGEIINLDD |
| 490 | 500 | 510 | 520 | 530 | 540 |
| YRIADATGYE | FVPMEEQNKE | NVKKEEPGIG | AEQQANGGIV | DNDVQLLEKP | TKLISQRKTI |
| 550 | 560 | 570 | 580 | 590 | 600 |
| EVNAQVQRID | FEGRSDGESM | LKILSQLRPR | RVIVIHGTAE | GTQVVARHCE | QNVGARVFTP |
| 610 | 620 | 630 | 640 | 650 | 660 |
| QKGEIIDVTS | EIHIYQVRLT | EGLVSQLQFQ | KGKDAEVAWV | DGRLGMRVKA | IEAPMDVTVE |
| 670 | 680 | 690 | 700 | 710 | 720 |
| QDASVQEGKT | LTLETLADDE | IPIHNSVLIN | ELKLSDFKQT | LMRNNINSEF | SGGVLWCSNG |
| 730 | 740 | 750 | |||
| TLALRRVDAG | KVAMEGCLSE | EYYKIRELLY | EQYAIV |