O17403
Gene name |
cpsf-2 (F09G2.4) |
Protein name |
Probable cleavage and polyadenylation specificity factor subunit 2 |
Names |
Cleavage and polyadenylation specificity factor 100 kDa subunit, CPSF 100 kDa subunit |
Species |
Caenorhabditis elegans |
KEGG Pathway |
cel:CELE_F09G2.4 |
EC number |
|
Protein Class |
|
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
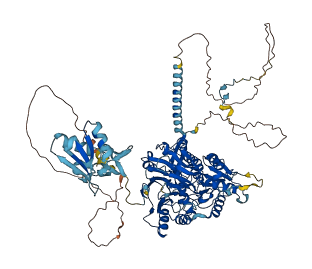
1 structures for O17403
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-O17403-F1 | Predicted | AlphaFoldDB |
No variants for O17403
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for O17403 | |||||
No associated diseases with O17403
5 regional properties for O17403
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Metallo-beta-lactamase | 17 - 222 | IPR001279 |
| domain | Zn-dependent metallo-hydrolase, RNA specificity domain | 563 - 619 | IPR011108 |
| domain | Beta-Casp domain | 242 - 368 | IPR022712 |
| domain | Cleavage and polyadenylation specificity factor 2, C-terminal | 642 - 840 | IPR025069 |
| domain | CPSF2, metallo-hydrolase domain | 10 - 203 | IPR035639 |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| mRNA cleavage and polyadenylation specificity factor complex | A multisubunit complex that binds to the canonical AAUAAA hexamer and to U-rich upstream sequence elements on the pre-mRNA, thereby stimulating the otherwise weakly active and nonspecific polymerase to elongate efficiently RNAs containing a poly(A) signal. |
1 GO annotations of molecular function
| Name | Definition |
|---|---|
| RNA binding | Binding to an RNA molecule or a portion thereof. |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| mRNA 3'-end processing | Any process involved in forming the mature 3' end of an mRNA molecule. |
| mRNA 3'-end processing by stem-loop binding and cleavage | Any mRNA 3'-end processing that involves the binding to and cleavage of a stem-loop structure. For example, histone mRNAs contain a highly conserved stem-loop sequence at the 3' end of the mRNA with a 6 base pairs (bp) stem and a 4-nt loop. The mRNA is cleaved between these two elements, after the fourth or fifth nucleotide, which is typically an adenosine. |
| mRNA polyadenylation | The enzymatic addition of a sequence of 40-200 adenylyl residues at the 3' end of a eukaryotic mRNA primary transcript. |
| pre-mRNA cleavage required for polyadenylation | The targeted, endonucleolytic cleavage of a pre-mRNA, required for polyadenylation of the 3' end. This cleavage is directed by binding sites near the 3' end of the mRNA and leaves a 3' hydoxyl end which then becomes a target for adenylation. |
4 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| Q12102 | CFT2 | Cleavage factor two protein 2 | Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) | PR |
| Q9V3D6 | Cpsf100 | Probable cleavage and polyadenylation specificity factor subunit 2 | Drosophila melanogaster (Fruit fly) | PR |
| Q9P2I0 | CPSF2 | Cleavage and polyadenylation specificity factor subunit 2 | Homo sapiens (Human) | PR |
| O35218 | Cpsf2 | Cleavage and polyadenylation specificity factor subunit 2 | Mus musculus (Mouse) | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MTSIIKLKVF | SGAKDEGPLC | YLLQVDGDYI | LLDCGWDERF | GLQYFEELKP | FIPKISAVLI |
| 70 | 80 | 90 | 100 | 110 | 120 |
| SHPDPLHLGG | LPYLVSKCGL | TAPVYATVPV | YKMGQMFIYD | MVYSHLDVEE | FEHYTLDDVD |
| 130 | 140 | 150 | 160 | 170 | 180 |
| TAFEKVEQVK | YNQTVVLKGD | SGVHFTALPA | GHMLGGSIWR | ICRVTGEDIV | YCVDFNHKKE |
| 190 | 200 | 210 | 220 | 230 | 240 |
| RHLNGCSFDN | FNRPHLLITG | AHHISLPQMR | RKDRDEQLVT | KILRTVRQKG | DCMIVIDTAG |
| 250 | 260 | 270 | 280 | 290 | 300 |
| RVLELAHLLD | QLWSNADAGL | STYNLVMMSH | VASSVVQFAK | SQLEWMNEKL | FKYDSSSARY |
| 310 | 320 | 330 | 340 | 350 | 360 |
| NPFTLKHVTL | CHSHQELMRV | RSPKVVLCSS | QDMESGFSRE | LFLDWCSDPR | NGVILTARPA |
| 370 | 380 | 390 | 400 | 410 | 420 |
| SFTLAAKLVN | MAERANDGVL | KHEDRLISLV | VKKRVALEGE | ELLEYKRRKA | ERDAEETRLR |
| 430 | 440 | 450 | 460 | 470 | 480 |
| MERARRQAQA | NESDDSDDDD | IAAPIVPRHS | EKDFRSFDGS | ENDAHTFDIM | AKWDNQQKAS |
| 490 | 500 | 510 | 520 | 530 | 540 |
| FFKTTKKSFP | MFPYIEEKVK | WDDYGEVIKP | EDYTVISKID | LRKGQNKDEP | VVVKKREEEE |
| 550 | 560 | 570 | 580 | 590 | 600 |
| EVYNPNDHVE | EMPTKCVEFK | NRVEVSCRIE | FIEYEGISDG | ESTKKLLAGL | LPRQIIVVHG |
| 610 | 620 | 630 | 640 | 650 | 660 |
| SRDDTRDLVA | YFADSGFDTT | MLKAPEAGAL | VDASVESFIY | QVALSDALLA | DIQFKEVSEG |
| 670 | 680 | 690 | 700 | 710 | 720 |
| NSLAWIDARV | MEKEAIDNML | AVGTSNLMID | DKNREEDVND | QEENGATEGE | GNAEPMEIGE |
| 730 | 740 | 750 | 760 | 770 | 780 |
| NGSQESLAIS | ESGKEVENGH | TNDSRTKKGT | KGKIRGNLIL | DPLPKRLIPI | HQAVFVNDPK |
| 790 | 800 | 810 | 820 | 830 | 840 |
| LSDFKNLLTD | KGYKAEFLSG | TLLINGGNCS | IRRNDTGVFQ | MEGAFTKDYY | KLRRLFYDQF |
| AVL |