Q8BJ71
Gene name |
Nup93 (Cip4, Kiaa0095) |
Protein name |
Nuclear pore complex protein Nup93 |
Names |
93 kDa nucleoporin, CBP-interacting protein 4, Nucleoporin Nup93 |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:71805 |
EC number |
|
Protein Class |
|
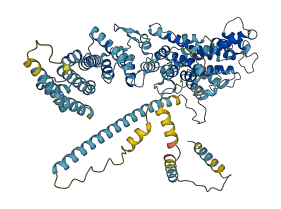
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q8BJ71
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q8BJ71-F1 | Predicted | AlphaFoldDB |
35 variants for Q8BJ71
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs3388997625 | 10 | L>H | No | EVA | |
| rs3388994918 | 21 | E>V | No | EVA | |
| rs3389006236 | 25 | E>V | No | EVA | |
| rs3389005392 | 50 | R>L | No | EVA | |
| rs3388989633 | 113 | A>V | No | EVA | |
| rs3388998678 | 117 | S>T | No | EVA | |
| rs3399447150 | 124 | M>K | No | EVA | |
| rs3389005356 | 131 | E>G | No | EVA | |
| rs3388993760 | 160 | Q>P | No | EVA | |
| rs3398546651 | 166 | Y>N | No | EVA | |
| rs3399005770 | 169 | D>Y | No | EVA | |
| rs3399394538 | 170 | V>E | No | EVA | |
| rs3399696765 | 170 | V>M | No | EVA | |
| rs3389002338 | 236 | T>I | No | EVA | |
| rs3388977857 | 257 | Q>E | No | EVA | |
| rs3388989651 | 305 | S>P | No | EVA | |
| rs3389006803 | 360 | D>Y | No | EVA | |
| rs3399394553 | 373 | L>P | No | EVA | |
| rs3388977900 | 393 | I>T | No | EVA | |
| rs3389001836 | 577 | S>G | No | EVA | |
| rs3399549109 | 615 | V>L | No | EVA | |
| rs3388970141 | 624 | E>* | No | EVA | |
| rs3388951479 | 625 | A>V | No | EVA | |
| rs3389005357 | 628 | L>F | No | EVA | |
| rs3389006792 | 654 | S>C | No | EVA | |
| rs3389002599 | 667 | A>G | No | EVA | |
| rs3388999910 | 689 | F>I | No | EVA | |
| rs3389005397 | 692 | L>I | No | EVA | |
| rs3389000153 | 708 | D>A | No | EVA | |
| rs3388952666 | 710 | A>D | No | EVA | |
| rs3389002357 | 736 | N>I | No | EVA | |
| rs3388995001 | 744 | N>Y | No | EVA | |
| rs3388994962 | 764 | K>I | No | EVA | |
| rs3389002609 | 809 | A>D | No | EVA | |
| rs3388952649 | 818 | M>I | No | EVA |
No associated diseases with Q8BJ71
No regional properties for Q8BJ71
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| No domain, repeats, and functional sites for Q8BJ71 | |||
Functions
5 GO annotations of cellular component
| Name | Definition |
|---|---|
| centrosome | A structure comprised of a core structure (in most organisms, a pair of centrioles) and peripheral material from which a microtubule-based structure, such as a spindle apparatus, is organized. Centrosomes occur close to the nucleus during interphase in many eukaryotic cells, though in animal cells it changes continually during the cell-division cycle. |
| nuclear envelope | The double lipid bilayer enclosing the nucleus and separating its contents from the rest of the cytoplasm; includes the intermembrane space, a gap of width 20-40 nm (also called the perinuclear space). |
| nuclear membrane | Either of the lipid bilayers that surround the nucleus and form the nuclear envelope; excludes the intermembrane space. |
| nuclear periphery | The portion of the nuclear lumen proximal to the inner nuclear membrane. |
| nuclear pore | A protein complex providing a discrete opening in the nuclear envelope of a eukaryotic cell, where the inner and outer nuclear membranes are joined. |
1 GO annotations of molecular function
| Name | Definition |
|---|---|
| structural constituent of nuclear pore | The action of a molecule that contributes to the structural integrity of the nuclear pore complex, a protein-lined channel in the nuclear envelope that allows the transfer of macromolecules. |
7 GO annotations of biological process
| Name | Definition |
|---|---|
| nuclear envelope organization | A process that is carried out at the cellular level which results in the assembly, arrangement of constituent parts, or disassembly of the nuclear envelope. |
| nuclear pore complex assembly | The aggregation, arrangement and bonding together of a set of components to form a nuclear pore complex. |
| nucleocytoplasmic transport | The directed movement of molecules between the nucleus and the cytoplasm. |
| poly(A)+ mRNA export from nucleus | The directed movement of poly(A)+ mRNA out of the nucleus into the cytoplasm. |
| positive regulation of SMAD protein signal transduction | Any process that increases the rate, frequency or extent of SMAD protein signal transduction. Pathway-restricted SMAD proteins and common-partner SMAD proteins are involved in the transforming growth factor beta receptor signaling pathways. |
| protein import into nucleus | The directed movement of a protein from the cytoplasm to the nucleus. |
| SMAD protein signal transduction | The cascade of processes by which a signal interacts with a receptor, causing a change in the activity of a SMAD protein, and ultimately effecting a change in the functioning of the cell. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MDTEGFGELL | QQAEQLAAET | EGISELPHVE | RNLQEIQQAG | ERLRSRTLTR | TSQETADVKA |
| 70 | 80 | 90 | 100 | 110 | 120 |
| SVLLGSRGLD | ISHISQRLES | LSAATTFEPL | EPVKDTDIQG | FLKNEKDNAL | LSAIEESRKR |
| 130 | 140 | 150 | 160 | 170 | 180 |
| TFGMAEEYHR | ESMLVEWEQV | KQRILHTLLA | SGEDALDFTQ | ESEPSYIGDV | NPPGRSSLDS |
| 190 | 200 | 210 | 220 | 230 | 240 |
| IEMAYARQIY | IYNEKIVSGH | LQPNLVDLCA | SVAELDDKSI | SDMWAMVKQM | TDVVLTPATD |
| 250 | 260 | 270 | 280 | 290 | 300 |
| ALKSRSSVEV | RMDFVKQALG | YLEQSYKNYT | LVTVFGNLHQ | AQLGGVPGTY | QLVRSFLNIK |
| 310 | 320 | 330 | 340 | 350 | 360 |
| LPAPSPGLQD | GEVEGHPVWA | LIYYCMRCGD | LLAASQVVSR | AQHQLGEFKT | WFQEYMNSKD |
| 370 | 380 | 390 | 400 | 410 | 420 |
| RRLSPATENK | LRLHYRRALR | NNTDPYKRAV | YCIIGRCDIT | DNQSEVADKT | EDYLWLKLNQ |
| 430 | 440 | 450 | 460 | 470 | 480 |
| VCFDDDGTSS | PQDRLTLSQF | QKQLLEDYGE | SHFTVNQQPF | LYFQVLFLTA | QFEAAIAFLF |
| 490 | 500 | 510 | 520 | 530 | 540 |
| RMERLRCHAV | HVALVLFELK | LLLKSSGQSA | QLLSHEPGDP | PCMRRLNFVR | LLMLYTRKFE |
| 550 | 560 | 570 | 580 | 590 | 600 |
| STDPREALQY | FYFLRDEKDS | QGENMFLRCV | SELVIESREF | DMILGKLEND | GSRKPGVIDK |
| 610 | 620 | 630 | 640 | 650 | 660 |
| FTSDTKPIIN | KVASVAENKG | LFEEAAKLYD | LAKNADKVLE | LMNKLLSPVV | PQISAPQSNK |
| 670 | 680 | 690 | 700 | 710 | 720 |
| ERLKNMALSI | AERYRAQGIS | ANKFVDSTFY | LLLDLITFFD | EYHSGHIDRA | FDIIDRLKLV |
| 730 | 740 | 750 | 760 | 770 | 780 |
| PLNQESVEER | VAAFRNFSDE | IRHNLSEVLL | ATMNILFTQF | KRLKGTSPSS | ATRPQRVIED |
| 790 | 800 | 810 | |||
| RDSQLRSQAR | ALITFAGMIP | YRTSGDTNAR | LVQMEVLMN |