Q80ZX8
Gene name |
Spag1 (Tpis) |
Protein name |
Sperm-associated antigen 1 |
Names |
Infertility-related sperm protein Spag-1, TPR-containing protein involved in spermatogenesis, TPIS |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:26942 |
EC number |
|
Protein Class |
|
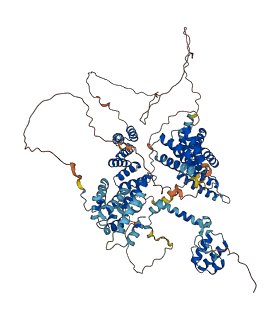
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q80ZX8
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q80ZX8-F1 | Predicted | AlphaFoldDB |
56 variants for Q80ZX8
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs3389359983 | 82 | P>H | No | EVA | |
| rs31774710 | 115 | C>R | No | EVA | |
| rs3389347519 | 146 | T>S | No | EVA | |
| rs216088357 | 148 | S>C | No | EVA | |
| rs240004463 | 157 | I>V | No | EVA | |
| rs247671738 | 160 | D>E | No | EVA | |
| rs3389347498 | 162 | A>T | No | EVA | |
| rs3389358707 | 164 | W>* | No | EVA | |
| rs3389372861 | 176 | I>F | No | EVA | |
| rs3389372855 | 179 | D>G | No | EVA | |
| rs3405153791 | 204 | L>Q | No | EVA | |
| rs3389372804 | 264 | S>T | No | EVA | |
| rs3389356829 | 305 | K>M | No | EVA | |
| rs3405485197 | 347 | E>D | No | EVA | |
| rs221428825 | 351 | S>L | No | EVA | |
| rs38088457 | 364 | E>A | No | EVA | |
| rs3389367528 | 375 | N>S | No | EVA | |
| rs3389320337 | 377 | Q>E | No | EVA | |
| rs3389328204 | 378 | K>T | No | EVA | |
| rs3389328242 | 421 | P>T | No | EVA | |
| rs3389367460 | 425 | R>* | No | EVA | |
| rs3389309506 | 441 | F>I | No | EVA | |
| rs3389354345 | 455 | V>M | No | EVA | |
| rs3389359939 | 456 | A>S | No | EVA | |
| rs3389278628 | 477 | N>H | No | EVA | |
| rs3389364166 | 488 | C>S | No | EVA | |
| rs3389372848 | 489 | R>W | No | EVA | |
| rs3389351400 | 498 | A>T | No | EVA | |
| rs3389320340 | 520 | E>K | No | EVA | |
| rs3389372877 | 540 | Q>H | No | EVA | |
| rs3389347545 | 560 | K>N | No | EVA | |
| rs3389352534 | 620 | K>R | No | EVA | |
| rs3389367507 | 636 | N>D | No | EVA | |
| rs36634162 | 664 | E>D | No | EVA | |
| rs253331252 | 664 | E>Q | No | EVA | |
| rs238147575 | 672 | E>K | No | EVA | |
| rs3389351387 | 689 | N>Y | No | EVA | |
| rs229698019 | 694 | G>R | No | EVA | |
| rs3406028330 | 701 | L>F | No | EVA | |
| rs236226673 | 706 | S>P | No | EVA | |
| rs32124828 | 711 | R>Q | No | EVA | |
| rs3389360581 | 730 | R>G | No | EVA | |
| rs256730961 | 741 | D>G | No | EVA | |
| rs3389367534 | 748 | A>E | No | EVA | |
| rs219481081 | 755 | A>T | No | EVA | |
| rs263197019 | 775 | V>F | No | EVA | |
| rs3389360659 | 786 | Q>E | No | EVA | |
| rs3405936060 | 789 | S>G | No | EVA | |
| rs235173091 | 793 | A>T | No | EVA | |
| rs3389328187 | 802 | H>Q | No | EVA | |
| rs3389354350 | 840 | D>V | No | EVA | |
| rs3389356813 | 844 | V>L | No | EVA | |
| rs3389367525 | 873 | A>V | No | EVA | |
| rs3389338928 | 881 | D>N | No | EVA | |
| rs3389347448 | 894 | A>D | No | EVA | |
| rs37851570 | 898 | Q>R | No | EVA |
No associated diseases with Q80ZX8
11 regional properties for Q80ZX8
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| repeat | Tetratricopeptide repeat 1 | 246 - 279 | IPR001440-1 |
| repeat | Tetratricopeptide repeat 1 | 642 - 672 | IPR001440-2 |
| repeat | Tetratricopeptide repeat | 213 - 246 | IPR019734-1 |
| repeat | Tetratricopeptide repeat | 246 - 279 | IPR019734-2 |
| repeat | Tetratricopeptide repeat | 280 - 313 | IPR019734-3 |
| repeat | Tetratricopeptide repeat | 430 - 463 | IPR019734-4 |
| repeat | Tetratricopeptide repeat | 472 - 505 | IPR019734-5 |
| repeat | Tetratricopeptide repeat | 506 - 539 | IPR019734-6 |
| repeat | Tetratricopeptide repeat | 606 - 639 | IPR019734-7 |
| repeat | Tetratricopeptide repeat | 640 - 673 | IPR019734-8 |
| domain | RNA-polymerase II-associated protein 3-like, C-terminal domain | 777 - 869 | IPR025986 |
4 GO annotations of cellular component
| Name | Definition |
|---|---|
| chaperone complex | A protein complex required for the non-covalent folding or unfolding, maturation, stabilization or assembly or disassembly of macromolecular structures. Usually active during or immediately after completion of translation. Many chaperone complexes contain heat shock proteins. |
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
| cytosol | The part of the cytoplasm that does not contain organelles but which does contain other particulate matter, such as protein complexes. |
| dynein axonemal particle | An aggregation of axonemal dyneins, their specific assembly factors, and broadly-acting chaperones that is located in the cytoplasm. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| GTP binding | Binding to GTP, guanosine triphosphate. |
| hydrolase activity | Catalysis of the hydrolysis of various bonds, e.g. C-O, C-N, C-C, phosphoric anhydride bonds, etc. |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| axonemal dynein complex assembly | The aggregation, arrangement and bonding together of a set of components to form an axonemal dynein complex, a dynein complex found in eukaryotic cilia and flagella, in which the motor domain heads interact with adjacent microtubules to generate a sliding force which is converted to a bending motion. |
| single fertilization | The union of male and female gametes to form a zygote. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MTAKAKDCPS | LWGFGTTKTF | KIPIEHLDFK | YIENCSDVKH | LEKILYVLRS | GEEGYYPELT |
| 70 | 80 | 90 | 100 | 110 | 120 |
| EFCEKCLTNL | APKSRALRKD | KPAETASSFS | AEEWEKIDSD | LKSWVSEIKR | EENTCHFHDP |
| 130 | 140 | 150 | 160 | 170 | 180 |
| ENHPGVEDPL | PPVRGSTCCP | HSGKETYSKS | KTAKKRIPRD | YAEWDKFDVE | KECSKIDEDY |
| 190 | 200 | 210 | 220 | 230 | 240 |
| KEKTVINNKA | HLSKIETKIE | TAGLTEKEKS | FLANREKGKG | NEAFYSGDYE | EAVMYYTRSL |
| 250 | 260 | 270 | 280 | 290 | 300 |
| SALPTAIAYN | NRAQAEIKLQ | RWSSALEDCE | KALELDPGNV | KALLRRATTY | KHQNKLQEAV |
| 310 | 320 | 330 | 340 | 350 | 360 |
| DDLRKVLQVE | PDNDLAKKTL | SEVERDLKNS | EPVSELQTKG | KRMVIEEVEN | SGDEGGKGSA |
| 370 | 380 | 390 | 400 | 410 | 420 |
| DEREDGGSDE | AAMGNIQKKL | MVRRSEGGRR | SRRGRTPGPR | AEQQGGLRET | ATASTGDSHY |
| 430 | 440 | 450 | 460 | 470 | 480 |
| PEEPRAADNP | SGLKRRGNEL | FRGGQFAEAA | AQYSVAIAQL | EPTGSANADE | LSILYSNRAA |
| 490 | 500 | 510 | 520 | 530 | 540 |
| CYLKEGNCRD | CIQDCNRALE | LHPFSVKPLL | RRAMAYETLE | QYRNAYVDYK | TVLQIDCGIQ |
| 550 | 560 | 570 | 580 | 590 | 600 |
| LASDSANRIA | RILTELDGSK | WRERLPPIPA | VPTSEPLRVW | LPAAETPDQD | PCPNNCMPSI |
| 610 | 620 | 630 | 640 | 650 | 660 |
| TDEKMFQALK | EEGNQLVKDK | NYKDAISKYN | ECLKINSKAC | AIYTNRALCY | LKLGQFEEAK |
| 670 | 680 | 690 | 700 | 710 | 720 |
| LDCEQALQID | GENVKASHRL | ALAQKGLENC | RESGVDPSQV | LLSPDSSEAA | RHLDTKNDTA |
| 730 | 740 | 750 | 760 | 770 | 780 |
| PPSKGRERRR | IQVQEVDGSS | DEEPERPAEA | SATSAPARDG | VEDGGSAEPA | EKLDVSKPTN |
| 790 | 800 | 810 | 820 | 830 | 840 |
| AYEFGQVLST | ISARKDEEAC | AHLLAITAPK | DLPLLLSNKL | EGDTFLLLIQ | SLKSHLVAKD |
| 850 | 860 | 870 | 880 | 890 | 900 |
| PSLVYEHLLY | LSKAERFKTM | LTLINKGQKE | QMAQLFDGLS | DTQSDGLTAE | DVQALRRQYE |
| L |