Q67EU8
Gene name |
RAD51A |
Protein name |
DNA repair protein RAD51 homolog A |
Names |
Rad51-like protein A, RAD51A, ZmRAD51a |
Species |
Zea mays (Maize) |
KEGG Pathway |
zma:541709 |
EC number |
|
Protein Class |
|
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
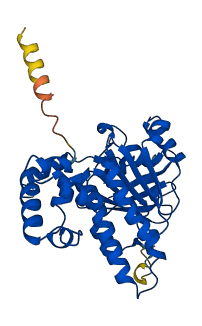
Autoinhibited structure

Activated structure
1 structures for Q67EU8
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q67EU8-F1 | Predicted | AlphaFoldDB |
No variants for Q67EU8
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q67EU8 | |||||
No associated diseases with Q67EU8
4 regional properties for Q67EU8
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | AAA+ ATPase domain | 120 - 307 | IPR003593 |
| domain | DNA recombination and repair protein Rad51-like, C-terminal | 85 - 337 | IPR013632 |
| domain | DNA recombination and repair protein RecA, monomer-monomer interface | 277 - 340 | IPR020587 |
| domain | DNA recombination and repair protein RecA-like, ATP-binding domain | 99 - 270 | IPR020588 |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| condensed nuclear chromosome | A highly compacted molecule of DNA and associated proteins resulting in a cytologically distinct nuclear chromosome. |
6 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP-dependent activity, acting on DNA | Catalytic activity that acts to modify DNA, driven by ATP hydrolysis. |
| ATP-dependent DNA damage sensor activity | A molecule that recognises toxic DNA structures, and initiates a signalling response, driven by ATP hydrolysis. |
| DNA strand exchange activity | Catalysis of the identification and base-pairing of homologous sequences between single-stranded DNA and double-stranded DNA. |
| double-stranded DNA binding | Binding to double-stranded DNA. |
| single-stranded DNA binding | Binding to single-stranded DNA. |
6 GO annotations of biological process
| Name | Definition |
|---|---|
| chromosome organization involved in meiotic cell cycle | A process of chromosome organization that is involved in a meiotic cell cycle. |
| DNA recombinase assembly | The aggregation, arrangement and bonding together of strand exchange proteins (recombinases) into higher order oligomers on single-stranded DNA. |
| mitotic recombination | The exchange, reciprocal or nonreciprocal, of genetic material between one DNA molecule and a homologous DNA region that occurs during mitotic cell cycles. |
| mitotic recombination-dependent replication fork processing | Replication fork processing that includes recombination between DNA near the arrested fork and homologous sequences. Proteins involved in homologous recombination are required for replication restart. |
| reciprocal meiotic recombination | The cell cycle process in which double strand breaks are formed and repaired through a single or double Holliday junction intermediate. This results in the equal exchange of genetic material between non-sister chromatids in a pair of homologous chromosomes. These reciprocal recombinant products ensure the proper segregation of homologous chromosomes during meiosis I and create genetic diversity. |
| strand invasion | The process in which the nucleoprotein complex (composed of the broken single-strand DNA and the recombinase) searches and identifies a region of homology in intact duplex DNA. The broken single-strand DNA displaces the like strand and forms Watson-Crick base pairs with its complement, forming a duplex in which each strand is from one of the two recombining DNA molecules. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSSAAQQQQK | AAAAEQEEVE | HGPFPIEQLQ | ASGIAALDVK | KLKDSGLHTV | EAVAYTPRKD |
| 70 | 80 | 90 | 100 | 110 | 120 |
| LLQIKGISEA | KADKIIEAAS | KIVPLGFTSA | SQLHAQRLEI | IQVTTGSREL | DKILEGGIET |
| 130 | 140 | 150 | 160 | 170 | 180 |
| GSITEIYGEF | RSGKTQLCHT | PCVTCQLPLD | QGGGEGKALY | IDAEGTFRPQ | RLLQIADRFG |
| 190 | 200 | 210 | 220 | 230 | 240 |
| LNGADVLENV | AYARAYNTDH | QSRLLLEAAS | MMIETRFALM | VVDSATALYR | TDFSGRGELS |
| 250 | 260 | 270 | 280 | 290 | 300 |
| ARQMHMAKFL | RSLQKLADEF | GVAVVITNQV | VAQVDGSAMF | AGPQFKPIGG | NIMAHASTTR |
| 310 | 320 | 330 | |||
| LALRKGRGEE | RICKVISSPC | LAEAEARFQL | ASEGIADVKD |