Q06411
Gene name |
SPP382 (CCF8, NTR1, YLR424W) |
Protein name |
Pre-mRNA-splicing factor SPP382 |
Names |
CLF1 complex factor 8, Nineteen complex-related protein 1, NTC-related protein 1, Suppressor of PRP38 protein 2 |
Species |
Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) |
KEGG Pathway |
sce:YLR424W |
EC number |
|
Protein Class |
|
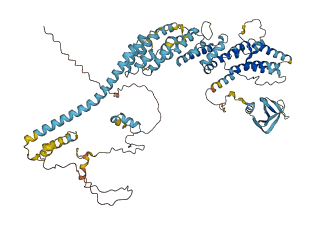
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
2 structures for Q06411
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| 5Y88 | EM | 370 A | U | 1-708 | PDB |
| AF-Q06411-F1 | Predicted | AlphaFoldDB |
26 variants for Q06411
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| s12-973494 | 35 | N>D | No | SGRP | |
| s12-973753 | 121 | Y>F | No | SGRP | |
| s12-973767 | 126 | D>N | No | SGRP | |
| s12-973881 | 164 | E>K | No | SGRP | |
| s12-973899 | 170 | V>I | No | SGRP | |
| s12-973909 | 173 | P>R | No | SGRP | |
| s12-973969 | 193 | V>A | No | SGRP | |
| s12-974067 | 226 | Y>H | No | SGRP | |
| s12-974104 | 238 | T>I | No | SGRP | |
| s12-974149 | 253 | G>A | No | SGRP | |
| s12-974182 | 264 | I>T | No | SGRP | |
| s12-974461 | 357 | S>N | No | SGRP | |
| s12-974554 | 388 | D>G | No | SGRP | |
| s12-974571 | 394 | I>V | No | SGRP | |
| s12-974628 | 413 | D>N | No | SGRP | |
| s12-974638 | 416 | E>G | No | SGRP | |
| s12-974751 | 454 | I>V | No | SGRP | |
| s12-974772 | 461 | P>S | No | SGRP | |
| s12-974904 | 505 | T>A | No | SGRP | |
| s12-974942 | 517 | M>I | No | SGRP | |
| s12-974947 | 519 | G>E | No | SGRP | |
| s12-974970 | 527 | I>V | No | SGRP | |
| s12-975016 | 542 | K>R | No | SGRP | |
| s12-975133 | 581 | Y>C | No | SGRP | |
| s12-975431 | 680 | M>I | No | SGRP | |
| s12-975492 | 701 | I>V | No | SGRP |
No associated diseases with Q06411
1 regional properties for Q06411
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | G-patch domain | 59 - 108 | IPR000467 |
7 GO annotations of cellular component
| Name | Definition |
|---|---|
| chromosome, telomeric region | The end of a linear chromosome, required for the integrity and maintenance of the end. A chromosome telomere usually includes a region of telomerase-encoded repeats the length of which rarely exceeds 20 bp each and that permits the formation of a telomeric loop (T-loop). The telomeric repeat region is usually preceded by a sub-telomeric region that is gene-poor but rich in repetitive elements. Some telomeres only consist of the latter part (for eg. D. melanogaster telomeres). |
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
| mitochondrion | A semiautonomous, self replicating organelle that occurs in varying numbers, shapes, and sizes in the cytoplasm of virtually all eukaryotic cells. It is notably the site of tissue respiration. |
| nucleolus | A small, dense body one or more of which are present in the nucleus of eukaryotic cells. It is rich in RNA and protein, is not bounded by a limiting membrane, and is not seen during mitosis. Its prime function is the transcription of the nucleolar DNA into 45S ribosomal-precursor RNA, the processing of this RNA into 5.8S, 18S, and 28S components of ribosomal RNA, and the association of these components with 5S RNA and proteins synthesized outside the nucleolus. This association results in the formation of ribonucleoprotein precursors; these pass into the cytoplasm and mature into the 40S and 60S subunits of the ribosome. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
| spliceosomal complex | Any of a series of ribonucleoprotein complexes that contain snRNA(s) and small nuclear ribonucleoproteins (snRNPs), and are formed sequentially during the spliceosomal splicing of one or more substrate RNAs, and which also contain the RNA substrate(s) from the initial target RNAs of splicing, the splicing intermediate RNA(s), to the final RNA products. During cis-splicing, the initial target RNA is a single, contiguous RNA transcript, whether mRNA, snoRNA, etc., and the released products are a spliced RNA and an excised intron, generally as a lariat structure. During trans-splicing, there are two initial substrate RNAs, the spliced leader RNA and a pre-mRNA. |
| U2-type post-mRNA release spliceosomal complex | A spliceosomal complex that is formed following the release of the spliced product from the post-spliceosomal complex and contains the excised intron and the U2, U5 and U6 snRNPs. |
1 GO annotations of molecular function
| Name | Definition |
|---|---|
| nucleic acid binding | Binding to a nucleic acid. |
6 GO annotations of biological process
| Name | Definition |
|---|---|
| generation of catalytic spliceosome for first transesterification step | Formation of a catalytic spliceosome complex ready to perform the first splicing reaction. This occurs by an ATP-dependent conformational change of the pre-catalytic spliceosome. |
| negative regulation of DNA ligase activity | Any process that stops, prevents or reduces the frequency, rate or extent of DNA ligase activity. |
| negative regulation of double-strand break repair via nonhomologous end joining | Any process that stops, prevents or reduces the frequency, rate or extent of double-strand break repair via nonhomologous end joining. |
| negative regulation of protein binding | Any process that stops, prevents, or reduces the frequency, rate or extent of protein binding. |
| negative regulation of protein-containing complex assembly | Any process that stops, prevents, or reduces the frequency, rate or extent of protein complex assembly. |
| spliceosomal complex disassembly | Disassembly of a spliceosomal complex with the ATP-dependent release of the product RNAs, one of which is composed of the joined exons. In cis splicing, the other product is the excised sequence, often a single intron, in a lariat structure. |
3 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| Q9UBB9 | TFIP11 | Tuftelin-interacting protein 11 | Homo sapiens (Human) | PR |
| Q9ERA6 | Tfip11 | Tuftelin-interacting protein 11 | Mus musculus (Mouse) | PR |
| Q9SLC6 | STIPL2 | Septin and tuftelin-interacting protein 1 homolog 2 | Arabidopsis thaliana (Mouse-ear cress) | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MEDSDSNTDK | KFFFKKRRID | SYNYSDEEDN | NSSMNSDMTY | TNDALKTSSG | NAPTISKLTK |
| 70 | 80 | 90 | 100 | 110 | 120 |
| TYGIGAKLLS | SMGYVAGKGL | GKDGSGITTP | IETQSRPMHN | AGLGMFSNTN | SSNYHSENED |
| 130 | 140 | 150 | 160 | 170 | 180 |
| YLSSEDEVVE | GIEQVKFNKT | STEVLGEALL | NDSGDMTIVR | TLRELRLAGV | QLPESILKEL |
| 190 | 200 | 210 | 220 | 230 | 240 |
| DPLNAVPKPK | KDVVVEILQE | LLGIEKSLEA | IRQRTSPLEV | QVKEYYGQER | LLSELEVTLR |
| 250 | 260 | 270 | 280 | 290 | 300 |
| DESKHVSLYD | KIGAILKLSD | DELIDRLTSC | LLRKELLIEF | DLDHLEKPND | ILDELTQIIE |
| 310 | 320 | 330 | 340 | 350 | 360 |
| LLAYRMDTTS | KFLNRTQTTI | FKVIYPKLKK | FWEGFDMTKS | KIDSAITLLL | DFQQVLSFIG |
| 370 | 380 | 390 | 400 | 410 | 420 |
| CKEHIMEEFV | YPKLLQELDN | WELHDEVDHV | SPRIWVLDFM | VLIDDKIKDT | IVDKIEAKFF |
| 430 | 440 | 450 | 460 | 470 | 480 |
| AYCKNWYHRE | SFCITNSDII | FIKELICERR | YYKILCKEFL | PKFLDELWER | HNDPIYELED |
| 490 | 500 | 510 | 520 | 530 | 540 |
| WKEKQEWKEK | DSGFFYFMKK | LRSYTHYFHP | KQYELMMRGT | FNNINKILYQ | WHLYSTVEDL |
| 550 | 560 | 570 | 580 | 590 | 600 |
| HKSKWWLNWL | MNTVFEHSLP | TEIELSEIRK | SYNIFAMSHR | YHLDKSTLDE | DFDLRQGLRN |
| 610 | 620 | 630 | 640 | 650 | 660 |
| LMETQVIDDI | SQSEQEPTYT | VQNIPLGKVS | SSFKDVVEDY | CLEKGYLISK | IPNRYTQLPY |
| 670 | 680 | 690 | 700 | ||
| GRDQDCIVPL | FEIRNGKKKM | EVALKHDILW | VEDSSGTFKP | IYLWALDL |