Q06010
Gene name |
STE23 (YLR389C, L8084.12) |
Protein name |
A-factor-processing enzyme |
Names |
Insulin-degrading enzyme homolog |
Species |
Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) |
KEGG Pathway |
sce:YLR389C |
EC number |
|
Protein Class |
|
Descriptions
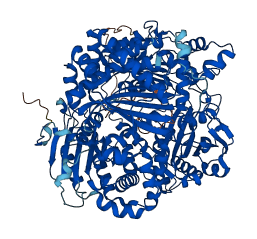
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q06010
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q06010-F1 | Predicted | AlphaFoldDB |
19 variants for Q06010
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| s12-902591 | 24 | L>F | No | SGRP | |
| s12-902330 | 111 | K>E | No | SGRP | |
| s12-901826 | 279 | D>N | No | SGRP | |
| s12-901778 | 295 | V>I | No | SGRP | |
| s12-901759 | 301 | P>L | No | SGRP | |
| s12-901752 | 303 | M>I | No | SGRP | |
| s12-901463 | 400 | V>I | No | SGRP | |
| s12-901058 | 535 | R>S | No | SGRP | |
| s12-901022 | 547 | D>H | No | SGRP | |
| s12-900850 | 604 | T>K | No | SGRP | |
| s12-900812 | 617 | V>L | No | SGRP | |
| s12-900451 | 737 | T>I | No | SGRP | |
| s12-900301 | 787 | E>G | No | SGRP | |
| s12-900280 | 794 | Q>R | No | SGRP | |
| s12-900124 | 846 | S>N | No | SGRP | |
| s12-899848 | 938 | A>V | No | SGRP | |
| s12-899794 | 956 | E>A | No | SGRP | |
| s12-899732 | 977 | N>D | No | SGRP | |
| s12-899580 | 1027 | E>D | No | SGRP |
No associated diseases with Q06010
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytosol | The part of the cytoplasm that does not contain organelles but which does contain other particulate matter, such as protein complexes. |
| extrinsic component of membrane | The component of a membrane consisting of gene products and protein complexes that are loosely bound to one of its surfaces, but not integrated into the hydrophobic region. |
| mitochondrion | A semiautonomous, self replicating organelle that occurs in varying numbers, shapes, and sizes in the cytoplasm of virtually all eukaryotic cells. It is notably the site of tissue respiration. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| metal ion binding | Binding to a metal ion. |
| metalloendopeptidase activity | Catalysis of the hydrolysis of internal, alpha-peptide bonds in a polypeptide chain by a mechanism in which water acts as a nucleophile, one or two metal ions hold the water molecule in place, and charged amino acid side chains are ligands for the metal ions. |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| peptide catabolic process | The chemical reactions and pathways resulting in the breakdown of peptides, compounds of 2 or more (but usually less than 100) amino acids where the alpha carboxyl group of one is bound to the alpha amino group of another. |
| peptide mating pheromone maturation involved in positive regulation of conjugation with cellular fusion | The formation of a mature peptide mating pheromone by proteolysis and/or modification of a peptide precursor, occurring in the context of conjugation with cellular fusion. |
| proteolysis involved in protein catabolic process | The hydrolysis of a peptide bond or bonds within a protein as part of the chemical reactions and pathways resulting in the breakdown of a protein by individual cells. |
| response to pheromone | Any process that results in a change in state or activity of a cell or an organism (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of a pheromone stimulus. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MGVSLLASSS | AFVTKPLLTQ | LVHLSPISLN | FTVRRFKPFT | CLSRYYTTNP | YNMTSNFKTF |
| 70 | 80 | 90 | 100 | 110 | 120 |
| NLDFLKPDLD | ERSYRFIELP | NKLKALLIQD | PKADKAAASL | DVNIGAFEDP | KNLPGLAHFC |
| 130 | 140 | 150 | 160 | 170 | 180 |
| EHLLFMGSEK | FPDENEYSSY | LSKHGGSSNA | YTASQNTNYF | FEVNHQHLFG | ALDRFSGFFS |
| 190 | 200 | 210 | 220 | 230 | 240 |
| CPLFNKDSTD | KEINAVNSEN | KKNLQNDIWR | IYQLDKSLTN | TKHPYHKFST | GNIETLGTLP |
| 250 | 260 | 270 | 280 | 290 | 300 |
| KENGLNVRDE | LLKFHKNFYS | ANLMKLCILG | REDLDTLSDW | TYDLFKDVAN | NGREVPLYAE |
| 310 | 320 | 330 | 340 | 350 | 360 |
| PIMQPEHLQK | IIQVRPVKDL | KKLEISFTVP | DMEEHWESKP | PRILSHLIGH | EGSGSLLAHL |
| 370 | 380 | 390 | 400 | 410 | 420 |
| KKLGWANELS | AGGHTVSKGN | AFFAVDIDLT | DNGLTHYRDV | IVLIFQYIEM | LKNSLPQKWI |
| 430 | 440 | 450 | 460 | 470 | 480 |
| FNELQDISNA | TFKFKQAGSP | SSTVSSLAKC | LEKDYIPVSR | ILAMGLLTKY | EPDLLTQYTD |
| 490 | 500 | 510 | 520 | 530 | 540 |
| ALVPENSRVT | LISRSLETDS | AEKWYGTAYK | VVDYPADLIK | NMKSPGLNPA | LTLPRPNEFV |
| 550 | 560 | 570 | 580 | 590 | 600 |
| STNFKVDKID | GIKPLDEPVL | LLSDDVSKLW | YKKDDRFWQP | RGYIYLSFKL | PHTHASIINS |
| 610 | 620 | 630 | 640 | 650 | 660 |
| MLSTLYTQLA | NDALKDVQYD | AACADLRISF | NKTNQGLAIT | ASGFNEKLII | LLTRFLQGVN |
| 670 | 680 | 690 | 700 | 710 | 720 |
| SFEPKKDRFE | ILKDKTIRHL | KNLLYEVPYS | QMSNYYNAII | NERSWSTAEK | LQVFEKLTFE |
| 730 | 740 | 750 | 760 | 770 | 780 |
| QLINFIPTIY | EGVYFETLIH | GNIKHEEALE | VDSLIKSLIP | NNIHNLQVSN | NRLRSYLLPK |
| 790 | 800 | 810 | 820 | 830 | 840 |
| GKTFRYETAL | KDSQNVNSCI | QHVTQLDVYS | EDLSALSGLF | AQLIHEPCFD | TLRTKEQLGY |
| 850 | 860 | 870 | 880 | 890 | 900 |
| VVFSSSLNNH | GTANIRILIQ | SEHTTPYLEW | RINNFYETFG | QVLRDMPEED | FEKHKEALCN |
| 910 | 920 | 930 | 940 | 950 | 960 |
| SLLQKFKNMA | EESARYTAAI | YLGDYNFTHR | QKKAKLVANI | TKQQMIDFYE | NYIMSENASK |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| LILHLKSQVE | NKELNENELD | TAKYPTGQLI | EDVGAFKSTL | FVAPVRQPMK | DFEISAPPKL |
| NNSSESE |