Q02197
Gene name |
MAK10 (NAA35, YEL053C) |
Protein name |
N-alpha-acetyltransferase 35, NatC auxiliary subunit |
Names |
Glucose repressible protein MAK10, L-A virus GAG protein N-acetyltransferase subunit MAK10, Maintenance of killer protein 10, N-terminal acetyltransferase C complex subunit MAK10, NatC complex subunit MAK10 |
Species |
Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) |
KEGG Pathway |
sce:YEL053C |
EC number |
|
Protein Class |
|
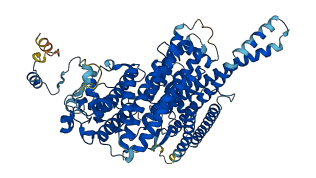
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
5 structures for Q02197
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| 6YGA | X-ray | 240 A | B | 1-733 | PDB |
| 6YGB | X-ray | 245 A | B | 1-733 | PDB |
| 6YGC | X-ray | 299 A | B | 1-733 | PDB |
| 6YGD | X-ray | 275 A | B | 1-733 | PDB |
| AF-Q02197-F1 | Predicted | AlphaFoldDB |
15 variants for Q02197
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| s05-56093 | 4 | D>H | No | SGRP | |
| s05-56039 | 22 | V>I | No | SGRP | |
| s05-56000 | 35 | P>S | No | SGRP | |
| s05-55880 | 75 | D>N | No | SGRP | |
| s05-55850 | 85 | A>S | No | SGRP | |
| s05-55841 | 88 | A>T | No | SGRP | |
| s05-55483 | 207 | A>E | No | SGRP | |
| s05-55321 | 261 | Q>P | No | SGRP | |
| s05-55304 | 267 | P>S | No | SGRP | |
| s05-55166 | 313 | K>E | No | SGRP | |
| s05-55132 | 324 | A>G | No | SGRP | |
| s05-54376 | 576 | F>S | No | SGRP | |
| s05-54237 | 622 | I>M | No | SGRP | |
| s05-54196 | 636 | R>H | No | SGRP | |
| s05-54188 | 639 | V>I | No | SGRP |
No associated diseases with Q02197
No regional properties for Q02197
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| No domain, repeats, and functional sites for Q02197 | |||
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
| cytosol | The part of the cytoplasm that does not contain organelles but which does contain other particulate matter, such as protein complexes. |
| NatC complex | A conserved complex that catalyzes the transfer of an acetyl group to the N-terminal residue of a protein acceptor molecule that has a Met-Ile, Met-Leu, Met-Trp, or Met-Phe N-terminus. In Saccharomyces the complex includes Mak3p, Mak10p, and Mak31p. |
No GO annotations of molecular function
| Name | Definition |
|---|---|
| No GO annotations for molecular function |
3 GO annotations of biological process
| Name | Definition |
|---|---|
| macroautophagy | The major inducible pathway for the general turnover of cytoplasmic constituents in eukaryotic cells, it is also responsible for the degradation of active cytoplasmic enzymes and organelles during nutrient starvation. Macroautophagy involves the formation of double-membrane-bounded autophagosomes which enclose the cytoplasmic constituent targeted for degradation in a membrane-bounded structure. Autophagosomes then fuse with a lysosome (or vacuole) releasing single-membrane-bounded autophagic bodies that are then degraded within the lysosome (or vacuole). Some types of macroautophagy, e.g. pexophagy, mitophagy, involve selective targeting of the targets to be degraded. |
| N-terminal peptidyl-methionine acetylation | The acetylation of the N-terminal methionine of proteins to form the derivative N-acetyl-L-methionine. |
| N-terminal protein amino acid acetylation | The acetylation of the N-terminal amino acid of proteins. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MEVDSILGSL | SITDDFDQLV | DVTSLFDELC | SKLKPEAIVK | DPRFDLFEGT | HSLEVNNSKL |
| 70 | 80 | 90 | 100 | 110 | 120 |
| DSSLIELTAE | EIEFDVNVAY | DPPLASVAAI | ADRLLRCVIS | WLNDYQTLPT | TVLSCRYTES |
| 130 | 140 | 150 | 160 | 170 | 180 |
| LLSSLVKGTT | AGSSWCTGNI | LYDKVLGSCI | LGVCYLTKFV | QKLLSAGIVF | EEEDLNFNNM |
| 190 | 200 | 210 | 220 | 230 | 240 |
| GFNTFDNLPG | QDVVINSLTE | SLQILEAYSD | DSLHLTMLKH | ILKIIICLVH | LEDHLTDYST |
| 250 | 260 | 270 | 280 | 290 | 300 |
| KTSHLDELIE | NANSVNGIFP | QLQLSPPKGA | FSTYIQKHRS | NQFPPRKITK | LPTDYSGFIT |
| 310 | 320 | 330 | 340 | 350 | 360 |
| LANDVKTILL | VDKAESALET | YQFAKFFNKL | EQRHVIARIL | FPLFFIRDDR | TVLGKFSYTQ |
| 370 | 380 | 390 | 400 | 410 | 420 |
| FYLLHVKEFS | AQTPSEFESS | IGNELIQESS | NMLLEWYQNC | SQNTCRYRQG | FNRQLILWDS |
| 430 | 440 | 450 | 460 | 470 | 480 |
| LQAQFESVNS | QVYCSWTYFM | KLSSMIEFSL | KGFDLDIYKP | FEAYSMFWYV | YYLSHHLETF |
| 490 | 500 | 510 | 520 | 530 | 540 |
| LKDSQNDIES | NINAIHSMNK | KLKKLKAGEK | KDQLRLKYRF | AMDNEMEQLQ | ATKQFLNYLL |
| 550 | 560 | 570 | 580 | 590 | 600 |
| KEINITKSLC | LIEVFQFAIL | KSFGLIDNKN | STPSKFSNER | LIHNLRFKPF | NSIGVPELPE |
| 610 | 620 | 630 | 640 | 650 | 660 |
| YEVFQQTLKD | FVIEEKGAAF | DIKLERATNF | IETEVRNVVS | SIDEIMQGIK | GGDNNGVLVT |
| 670 | 680 | 690 | 700 | 710 | 720 |
| GTRLVQELSL | EYYCKLKHTS | KALSVNSKVI | VNTLKKNIKN | KDSHEYKVEL | VHTTEGWNYF |
| 730 | |||||
| PIQTLRIKQD | RYK |