P25615
Gene name |
POL4 (POLX, YCR014C, YCR14C) |
Protein name |
DNA polymerase IV |
Names |
POL IV |
Species |
Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) |
KEGG Pathway |
sce:YCR014C |
EC number |
2.7.7.7: Nucleotidyltransferases |
Protein Class |
|
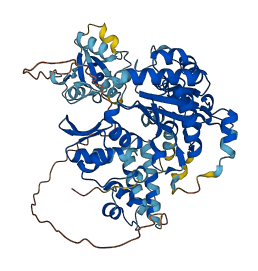
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for P25615
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-P25615-F1 | Predicted | AlphaFoldDB |
12 variants for P25615
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| s03-140787 | 49 | V>I | No | SGRP | |
| s03-140654 | 93 | V>A | No | SGRP | |
| s03-140476 | 152 | D>E | No | SGRP | |
| s03-140420 | 171 | G>E | No | SGRP | |
| s03-140384 | 183 | T>M | No | SGRP | |
| s03-140336 | 199 | T>K | No | SGRP | |
| s03-140028 | 302 | K>E | No | SGRP | |
| s03-139932 | 334 | T>A | No | SGRP | |
| s03-139838 | 365 | C>S | No | SGRP | |
| s03-139686 | 416 | K>Q | No | SGRP | |
| s03-139547 | 462 | M>K | No | SGRP | |
| s03-139187 | 582 | A>G | No | SGRP |
No associated diseases with P25615
5 regional properties for P25615
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | DNA-directed DNA polymerase X | 185 - 574 | IPR002054 |
| domain | DNA polymerase beta-like, N-terminal domain | 188 - 254 | IPR010996 |
| binding_site | DNA polymerase family X, binding site | 356 - 375 | IPR019843 |
| domain | DNA polymerase beta, palm domain | 327 - 406 | IPR028207 |
| domain | DNA polymerase beta, thumb domain | 516 - 574 | IPR029398 |
Functions
| Description | ||
|---|---|---|
| EC Number | 2.7.7.7 | Nucleotidyltransferases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
3 GO annotations of molecular function
| Name | Definition |
|---|---|
| DNA binding | Any molecular function by which a gene product interacts selectively and non-covalently with DNA (deoxyribonucleic acid). |
| DNA-directed DNA polymerase activity | Catalysis of the reaction: deoxynucleoside triphosphate + DNA(n) = diphosphate + DNA(n+1); the synthesis of DNA from deoxyribonucleotide triphosphates in the presence of a DNA template and a 3'hydroxyl group. |
| metal ion binding | Binding to a metal ion. |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| double-strand break repair | The repair of double-strand breaks in DNA via homologous and nonhomologous mechanisms to reform a continuous DNA helix. |
| double-strand break repair via nonhomologous end joining | The repair of a double-strand break in DNA in which the two broken ends are rejoined with little or no sequence complementarity. Information at the DNA ends may be lost due to the modification of broken DNA ends. This term covers instances of separate pathways, called classical (or canonical) and alternative nonhomologous end joining (C-NHEJ and A-NHEJ). These in turn may further branch into sub-pathways, but evidence is still unclear. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSLKGKFFAF | LPNPNTSSNK | FFKSILEKKG | ATIVSSIQNC | LQSSRKEVVI | LIEDSFVDSD |
| 70 | 80 | 90 | 100 | 110 | 120 |
| MHLTQKDIFQ | REAGLNDVDE | FLGKIEQSGI | QCVKTSCITK | WVQNDKFAFQ | KDDLIKFQPS |
| 130 | 140 | 150 | 160 | 170 | 180 |
| IIVISDNADD | GQSSTDKESE | ISTDVESERN | DDSNNKDMIQ | ASKPLKRLLQ | GDKGRASLVT |
| 190 | 200 | 210 | 220 | 230 | 240 |
| DKTKYKNNEL | IIGALKRLTK | KYEIEGEKFR | ARSYRLAKQS | MENCDFNVRS | GEEAHTKLRN |
| 250 | 260 | 270 | 280 | 290 | 300 |
| IGPSIAKKIQ | VILDTGVLPG | LNDSVGLEDK | LKYFKNCYGI | GSEIAKRWNL | LNFESFCVAA |
| 310 | 320 | 330 | 340 | 350 | 360 |
| KKDPEEFVSD | WTILFGWSYY | DDWLCKMSRN | ECFTHLKKVQ | KALRGIDPEC | QVELQGSYNR |
| 370 | 380 | 390 | 400 | 410 | 420 |
| GYSKCGDIDL | LFFKPFCNDT | TELAKIMETL | CIKLYKDGYI | HCFLQLTPNL | EKLFLKRIVE |
| 430 | 440 | 450 | 460 | 470 | 480 |
| RFRTAKIVGY | GERKRWYSSE | IIKKFFMGVK | LSPRELEELK | EMKNDEGTLL | IEEEEEEETK |
| 490 | 500 | 510 | 520 | 530 | 540 |
| LKPIDQYMSL | NAKDGNYCRR | LDFFCCKWDE | LGAGRIHYTG | SKEYNRWIRI | LAAQKGFKLT |
| 550 | 560 | 570 | 580 | ||
| QHGLFRNNIL | LESFNERRIF | ELLNLKYAEP | EHRNIEWEKK | TA |