E9Q4Z2
Gene name |
Acacb |
Protein name |
Acetyl-CoA carboxylase 2 |
Names |
ACC-beta |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:100705 |
EC number |
6.4.1.2: Forming carbon-carbon bonds |
Protein Class |
|
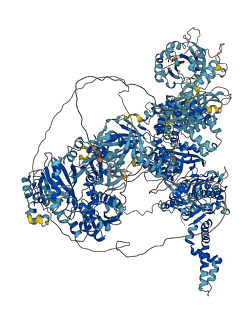
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for E9Q4Z2
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-E9Q4Z2-F1 | Predicted | AlphaFoldDB |
114 variants for E9Q4Z2
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs3388777524 | 39 | A>T | No | EVA | |
| rs51877709 | 40 | N>S | No | EVA | |
| rs240131872 | 55 | G>E | No | EVA | |
| rs3388777578 | 60 | E>V | No | EVA | |
| rs225090511 | 64 | H>Q | No | EVA | |
| rs45917980 | 64 | H>R | No | EVA | |
| rs3388753754 | 78 | Q>* | No | EVA | |
| rs232958066 | 78 | Q>H | No | EVA | |
| rs47813780 | 88 | R>K | No | EVA | |
| rs3388767913 | 97 | N>T | No | EVA | |
| rs3388781546 | 98 | D>H | No | EVA | |
| rs3388782653 | 101 | P>T | No | EVA | |
| rs215608464 | 109 | W>C | No | EVA | |
| rs226038449 | 110 | T>P | No | EVA | |
| rs212554964 | 112 | A>G | No | EVA | |
| rs3388770646 | 120 | A>T | No | EVA | |
| rs217854757 | 130 | P>L | No | EVA | |
| rs3388788746 | 136 | S>F | No | EVA | |
| rs3388782143 | 140 | E>G | No | EVA | |
| rs3388781568 | 155 | F>I | No | EVA | |
| rs3388775226 | 180 | K>R | No | EVA | |
| rs3388770669 | 206 | T>I | No | EVA | |
| rs3388785795 | 225 | K>N | No | EVA | |
| rs3396016677 | 237 | P>Q | No | EVA | |
| rs3395958201 | 238 | A>T | No | EVA | |
| rs3411342105 | 272 | W>* | No | EVA | |
| rs3388753685 | 280 | E>K | No | EVA | |
| rs232572141 | 284 | R>W | No | EVA | |
| rs3388782418 | 338 | W>* | No | EVA | |
| rs3395679169 | 343 | H>P | No | EVA | |
| rs3388782675 | 373 | G>R | No | EVA | |
| rs3396086846 | 382 | A>P | No | EVA | |
| rs3388781630 | 400 | E>* | No | EVA | |
| rs3388782187 | 476 | G>D | No | EVA | |
| rs3388781598 | 479 | I>T | No | EVA | |
| rs3388782155 | 493 | V>I | No | EVA | |
| rs3388767838 | 494 | Q>H | No | EVA | |
| rs3388782123 | 503 | A>V | No | EVA | |
| rs3388779791 | 533 | V>M | No | EVA | |
| rs3388762986 | 570 | E>* | No | EVA | |
| rs3388767878 | 573 | P>L | No | EVA | |
| rs3388788757 | 580 | P>T | No | EVA | |
| rs3388777559 | 593 | A>T | No | EVA | |
| rs3388782668 | 602 | P>H | No | EVA | |
| rs3388782638 | 666 | S>G | No | EVA | |
| rs3388767892 | 673 | Y>N | No | EVA | |
| rs3388782141 | 680 | G>W | No | EVA | |
| rs3388762934 | 694 | F>S | No | EVA | |
| rs3388782655 | 770 | L>F | No | EVA | |
| rs3388781608 | 807 | L>M | No | EVA | |
| rs3388767884 | 821 | Q>H | No | EVA | |
| rs3388782430 | 835 | I>M | No | EVA | |
| rs3388770653 | 859 | Y>* | No | EVA | |
| rs3388767876 | 897 | Q>H | No | EVA | |
| rs3388781586 | 900 | V>M | No | EVA | |
| rs3388778685 | 905 | H>R | No | EVA | |
| rs3388770692 | 941 | I>L | No | EVA | |
| rs3388775188 | 948 | V>M | No | EVA | |
| rs3395679771 | 1004 | E>G | No | EVA | |
| rs3395673593 | 1013 | D>V | No | EVA | |
| rs3388779779 | 1018 | L>P | No | EVA | |
| rs3388785821 | 1049 | K>Q | No | EVA | |
| rs3388773485 | 1062 | I>V | No | EVA | |
| rs3388788696 | 1079 | D>G | No | EVA | |
| rs3388782483 | 1102 | V>A | No | EVA | |
| rs3388779797 | 1142 | C>S | No | EVA | |
| rs3388779786 | 1156 | Q>R | No | EVA | |
| rs3388782600 | 1202 | L>P | No | EVA | |
| rs3388781584 | 1303 | E>V | No | EVA | |
| rs3388781629 | 1335 | D>H | No | EVA | |
| rs3388753710 | 1364 | R>I | No | EVA | |
| rs3388767867 | 1379 | F>Y | No | EVA | |
| rs47121625 | 1387 | L>P | No | EVA | |
| rs3388785824 | 1431 | V>I | No | EVA | |
| rs3388782198 | 1533 | R>Q | No | EVA | |
| rs3388773504 | 1596 | K>M | No | EVA | |
| rs3388785863 | 1616 | R>* | No | EVA | |
| rs3388775207 | 1619 | Q>H | No | EVA | |
| rs3388762933 | 1631 | S>* | No | EVA | |
| rs3388767900 | 1639 | L>I | No | EVA | |
| rs3388775202 | 1716 | Q>* | No | EVA | |
| rs3388785831 | 1729 | P>L | No | EVA | |
| rs3388753691 | 1751 | R>L | No | EVA | |
| rs3388788740 | 1759 | G>D | No | EVA | |
| rs3388783382 | 1774 | E>D | No | EVA | |
| rs220649250 | 1779 | V>I | No | EVA | |
| rs3388781623 | 1786 | T>N | No | EVA | |
| rs3388770703 | 1804 | S>Y | No | EVA | |
| rs3388785798 | 1805 | E>V | No | EVA | |
| rs3388788691 | 1851 | Y>N | No | EVA | |
| rs3388782623 | 1899 | R>G | No | EVA | |
| rs1134351994 | 1919 | S>G | No | EVA | |
| rs33236572 | 1925 | A>T | No | EVA | |
| rs3388767874 | 1933 | V>M | No | EVA | |
| rs3388773473 | 1954 | A>T | No | EVA | |
| rs3388782480 | 1954 | A>V | No | EVA | |
| rs3388775215 | 1971 | G>S | No | EVA | |
| rs3388777493 | 2005 | K>R | No | EVA | |
| rs3388782414 | 2007 | N>D | No | EVA | |
| rs3388788699 | 2011 | V>I | No | EVA | |
| rs3388775222 | 2101 | D>H | No | EVA | |
| rs50223129 | 2120 | F>C | No | EVA | |
| rs3388775255 | 2158 | Y>C | No | EVA | |
| rs3388777489 | 2183 | I>L | No | EVA | |
| rs3388773464 | 2249 | V>M | No | EVA | |
| rs3388775174 | 2311 | T>I | No | EVA | |
| rs3388775187 | 2350 | R>L | No | EVA | |
| rs3396087665 | 2357 | E>A | No | EVA | |
| rs3388773496 | 2368 | N>S | No | EVA | |
| rs49366190 | 2388 | T>N | No | EVA | |
| rs3388775236 | 2391 | E>V | No | EVA | |
| rs3388777551 | 2392 | N>S | No | EVA | |
| rs3388775245 | 2396 | L>Q | No | EVA | |
| rs3388781243 | 2408 | L>P | No | EVA |
No associated diseases with E9Q4Z2
10 regional properties for E9Q4Z2
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Biotin/lipoyl attachment | 878 - 952 | IPR000089 |
| domain | Carbamoyl-phosphate synthetase large subunit-like, ATP-binding domain | 421 - 604 | IPR005479 |
| domain | Biotin carboxylase-like, N-terminal domain | 250 - 369 | IPR005481 |
| domain | Biotin carboxylase, C-terminal | 640 - 747 | IPR005482 |
| domain | ATP-grasp fold | 408 - 599 | IPR011761 |
| domain | Acetyl-coenzyme A carboxyltransferase, N-terminal | 1685 - 2015 | IPR011762 |
| domain | Acetyl-coenzyme A carboxyltransferase, C-terminal | 2019 - 2335 | IPR011763 |
| domain | Biotin carboxylation domain | 249 - 751 | IPR011764 |
| domain | Acetyl-CoA carboxylase, central domain | 952 - 1678 | IPR013537 |
| domain | Acetyl-CoA carboxylase | 1770 - 2323 | IPR034733 |
Functions
| Description | ||
|---|---|---|
| EC Number | 6.4.1.2 | Forming carbon-carbon bonds |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
2 GO annotations of cellular component
| Name | Definition |
|---|---|
| mitochondrion | A semiautonomous, self replicating organelle that occurs in varying numbers, shapes, and sizes in the cytoplasm of virtually all eukaryotic cells. It is notably the site of tissue respiration. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| acetyl-CoA carboxylase activity | Catalysis of the reaction: ATP + acetyl-CoA + HCO3- = ADP + phosphate + malonyl-CoA. |
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| biotin binding | Binding to biotin (cis-tetrahydro-2-oxothieno(3,4-d)imidazoline-4-valeric acid), the (+) enantiomer of which is very widely distributed in cells and serves as a carrier in a number of enzymatic beta-carboxylation reactions. |
| identical protein binding | Binding to an identical protein or proteins. |
| metal ion binding | Binding to a metal ion. |
16 GO annotations of biological process
| Name | Definition |
|---|---|
| acetyl-CoA metabolic process | The chemical reactions and pathways involving acetyl-CoA, a derivative of coenzyme A in which the sulfhydryl group is acetylated; it is a metabolite derived from several pathways (e.g. glycolysis, fatty acid oxidation, amino-acid catabolism) and is further metabolized by the tricarboxylic acid cycle. It is a key intermediate in lipid and terpenoid biosynthesis. |
| energy homeostasis | Any process involved in the balance between food intake (energy input) and energy expenditure. |
| fatty acid biosynthetic process | The chemical reactions and pathways resulting in the formation of a fatty acid, any of the aliphatic monocarboxylic acids that can be liberated by hydrolysis from naturally occurring fats and oils. Fatty acids are predominantly straight-chain acids of 4 to 24 carbon atoms, which may be saturated or unsaturated; branched fatty acids and hydroxy fatty acids also occur, and very long chain acids of over 30 carbons are found in waxes. |
| malonyl-CoA biosynthetic process | The chemical reactions and pathways resulting in the formation of malonyl-CoA, the S-malonyl derivative of coenzyme A. |
| negative regulation of catalytic activity | Any process that stops or reduces the activity of an enzyme. |
| negative regulation of fatty acid beta-oxidation | Any process that stops, prevents, or reduces the frequency, rate or extent of fatty acid beta-oxidation. |
| negative regulation of fatty acid oxidation | Any process that stops, prevents, or reduces the frequency, rate or extent of fatty acid oxidation. |
| negative regulation of gene expression | Any process that decreases the frequency, rate or extent of gene expression. Gene expression is the process in which a gene's coding sequence is converted into a mature gene product (protein or RNA). |
| negative regulation of lipid catabolic process | Any process that stops, prevents, or reduces the frequency, rate or extent of the chemical reactions and pathways resulting in the breakdown of lipids. |
| positive regulation of heart growth | Any process that increases the rate or extent of heart growth. Heart growth is the increase in size or mass of the heart. |
| positive regulation of lipid storage | Any process that increases the rate, frequency or extent of lipid storage. Lipid storage is the accumulation and maintenance in cells or tissues of lipids, compounds soluble in organic solvents but insoluble or sparingly soluble in aqueous solvents. Lipid reserves can be accumulated during early developmental stages for mobilization and utilization at later stages of development. |
| protein homotetramerization | The formation of a protein homotetramer, a macromolecular structure consisting of four noncovalently associated identical subunits. |
| regulation of glucose metabolic process | Any process that modulates the rate, frequency or extent of glucose metabolism. Glucose metabolic processes are the chemical reactions and pathways involving glucose, the aldohexose gluco-hexose. |
| response to nutrient levels | Any process that results in a change in state or activity of a cell or an organism (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of a stimulus reflecting the presence, absence, or concentration of nutrients. |
| response to organic cyclic compound | Any process that results in a change in state or activity of a cell or an organism (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of an organic cyclic compound stimulus. |
| response to xenobiotic stimulus | Any process that results in a change in state or activity of a cell or an organism (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of a stimulus from a xenobiotic, a compound foreign to the organim exposed to it. It may be synthesized by another organism (like ampicilin) or it can be a synthetic chemical. |
5 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| P11029 | ACAC | Acetyl-CoA carboxylase | Gallus gallus (Chicken) | PR |
| Q13085 | ACACA | Acetyl-CoA carboxylase 1 | Homo sapiens (Human) | PR |
| O00763 | ACACB | Acetyl-CoA carboxylase 2 | Homo sapiens (Human) | PR |
| Q5SWU9 | Acaca | Acetyl-CoA carboxylase 1 | Mus musculus (Mouse) | PR |
| P11497 | Acaca | Acetyl-CoA carboxylase 1 | Rattus norvegicus (Rat) | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MVLLLFLTCL | VFSCLTFSWL | KIWGKMTDSK | PLTNSKVEAN | LLSSEESLSA | SELSGEQLQE |
| 70 | 80 | 90 | 100 | 110 | 120 |
| HGDHSCLSYR | GPRDASQQRN | SLPSSCQRPP | RNPLSSNDTW | PSPELQTNWT | AAPGPEVPDA |
| 130 | 140 | 150 | 160 | 170 | 180 |
| NGLSFPARPP | SQRTVSPSRE | DRKQAHIKRQ | LMTSFILGSL | DDNSSDEDPS | AGSFQNSSRK |
| 190 | 200 | 210 | 220 | 230 | 240 |
| SSRASLGTLS | QEAALNTSDP | ESHAPTMRPS | MSGLHLVKRG | REHKKLDLHR | DFTVASPAEF |
| 250 | 260 | 270 | 280 | 290 | 300 |
| VTRFGGNRVI | EKVLIANNGI | AAVKCMRSIR | RWAYEMFRNE | RAIRFVVMVT | PEDLKANAEY |
| 310 | 320 | 330 | 340 | 350 | 360 |
| IKMADQYVPV | PGGPNNNNYA | NVELIIDIAK | RIPVQAVWAG | WGHASENPKL | PELLCKHEIA |
| 370 | 380 | 390 | 400 | 410 | 420 |
| FLGPPSEAMW | ALGDKIASTI | VAQTLQIPTL | PWSGSGLTVE | WTEDSRHQGK | CISVPEDVYE |
| 430 | 440 | 450 | 460 | 470 | 480 |
| QGCVKDVDEG | LQAAEKIGFP | LMIKASEGGG | GKGIRKAESA | EDFPMLFRQV | QSEIPGSPIF |
| 490 | 500 | 510 | 520 | 530 | 540 |
| LMKLAQNARH | LEVQVLADQY | GNAVSLFGRD | CSIQRRHQKI | IEEAPATIAA | PAVFEFMEQC |
| 550 | 560 | 570 | 580 | 590 | 600 |
| AVLLAKMVGY | VSAGTVEYLY | SQDGSFHFLE | LNPRLQVEHP | CTEMIADVNL | PAAQLQIAMG |
| 610 | 620 | 630 | 640 | 650 | 660 |
| VPLHRLKDIR | LLYGESPWGV | TPIPFETPLS | PPIARGHVIA | ARITSENPDE | GFKPSSGTVQ |
| 670 | 680 | 690 | 700 | 710 | 720 |
| ELNFRSNKNV | WGYFSVAAAG | GLHEFADSQF | GHCFSWGENR | EEAISNMVVA | LKELSIRGDF |
| 730 | 740 | 750 | 760 | 770 | 780 |
| RTTVEYLVNL | LETESFQNND | IDTGWLDHLI | AQRVQAEKPD | IMLGVVCGAL | NVADAMFRTC |
| 790 | 800 | 810 | 820 | 830 | 840 |
| MTEFLHSLER | GQVLPADSLL | NIVDVELIYG | GIKYALKVAR | QSLTMFVLIM | NGCHIEIDAH |
| 850 | 860 | 870 | 880 | 890 | 900 |
| RLNDGGLLLS | YNGSSYTTYM | KEEVDSYRIT | IGNKTCVFEK | ENDPTVLRSP | SAGKLMQYTV |
| 910 | 920 | 930 | 940 | 950 | 960 |
| EDGDHVEAGS | SYAEMEVMKM | IMTLNVQESG | RVKYIKRPGV | ILEAGCVVAR | LELDDPSKVH |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| AAQPFTGELP | AQQTLPILGE | KLHQVFHGVL | ENLTNVMSGY | CLPEPFFSMK | LKDWVQKLMM |
| 1030 | 1040 | 1050 | 1060 | 1070 | 1080 |
| TLRHPSLPLL | ELQEIMTSVA | GRIPAPVEKA | VRRVMAQYAS | NITSVLCQFP | SQQIATILDC |
| 1090 | 1100 | 1110 | 1120 | 1130 | 1140 |
| HAATLQRKAD | REVFFMNTQS | IVQLVQRYRS | GTRGYMKAVV | LDLLRKYLNV | EHHFQQAHYD |
| 1150 | 1160 | 1170 | 1180 | 1190 | 1200 |
| KCVINLREQF | KPDMTQVLDC | IFSHSQVAKK | NQLVTMLIDE | LCGPDPTLSD | ELTSILCELT |
| 1210 | 1220 | 1230 | 1240 | 1250 | 1260 |
| QLSRSEHCKV | ALRARQVLIA | SHLPSYELRH | NQVESIFLSA | IDMYGHQFCP | ENLKKLILSE |
| 1270 | 1280 | 1290 | 1300 | 1310 | 1320 |
| TTIFDVLPTF | FYHENKVVCM | ASLEVYVRRG | YIAYELNSLQ | HRELPDGTCV | VEFQFMLPSS |
| 1330 | 1340 | 1350 | 1360 | 1370 | 1380 |
| HPNRMAVPIS | VSNPDLLRHS | TELFMDSGFS | PLCQRMGAMV | AFRRFEEFTR | NFDEVISCFA |
| 1390 | 1400 | 1410 | 1420 | 1430 | 1440 |
| NVQTDTLLFS | KACTSLYSEE | DSKSLREEPI | HILNVAIQCA | DHMEDEALVP | VFRAFVQSKK |
| 1450 | 1460 | 1470 | 1480 | 1490 | 1500 |
| HILVDYGLRR | ITFLVAQERE | FPKFFTFRAR | DEFAEDRIYR | HLEPALAFQL | ELSRMRNFDL |
| 1510 | 1520 | 1530 | 1540 | 1550 | 1560 |
| TAVPCANHKM | HLYLGAAKVK | EGLEVTDHRF | FIRAIIRHSD | LITKEASFEY | LQNEGERLLL |
| 1570 | 1580 | 1590 | 1600 | 1610 | 1620 |
| EAMDELEVAF | NNTSVRTDCN | HIFLNFVPTV | IMDPLKIEES | VRDMVMRYGS | RLWKLRVLQA |
| 1630 | 1640 | 1650 | 1660 | 1670 | 1680 |
| EVKINIRQTT | SDSAIPIRLF | ITNESGYYLD | ISLYREVTDS | RSGNIMFHSF | GNKQGSLHGM |
| 1690 | 1700 | 1710 | 1720 | 1730 | 1740 |
| LINTPYVTKD | LLQAKRFQAQ | SLGTTYVYDF | PEMFRQALFK | LWGSPEKYPK | DILTYTELVL |
| 1750 | 1760 | 1770 | 1780 | 1790 | 1800 |
| DSQGQLVEMN | RLPGCNEVGM | VAFKMRFKTP | EYPEGRDAVV | IGNDITFQIG | SFGIGEDFLY |
| 1810 | 1820 | 1830 | 1840 | 1850 | 1860 |
| LRASEMARTE | GIPQIYLAAN | SGARMGLAEE | IKQIFQVAWV | DPEDPHKGFR | YLYLTPQDYT |
| 1870 | 1880 | 1890 | 1900 | 1910 | 1920 |
| QISSQNSVHC | KHIEDEGESR | YVIVDVIGKD | ANLGVENLRG | SGMIAGEASL | AYEKTVTISM |
| 1930 | 1940 | 1950 | 1960 | 1970 | 1980 |
| VTCRALGIGA | YLVRLGQRVI | QVENSHIILT | GAGALNKVLG | REVYTSNNQL | GGVQIMHTNG |
| 1990 | 2000 | 2010 | 2020 | 2030 | 2040 |
| VSHVTVPDDF | EGVCTILEWL | SFIPKDNRSP | VPITTPSDPI | DREIEFTPTK | APYDPRWMLA |
| 2050 | 2060 | 2070 | 2080 | 2090 | 2100 |
| GRPHPTLKGT | WQSGFFDHGS | FKEIMAPWAQ | TVVTGRARLG | GIPVGVIAVE | TRTVEVAVPA |
| 2110 | 2120 | 2130 | 2140 | 2150 | 2160 |
| DPANLDSEAK | IIQQAGQVWF | PDSAYKTAQV | IRDFNKERLP | LMIFANWRGF | SGGMKDMYEQ |
| 2170 | 2180 | 2190 | 2200 | 2210 | 2220 |
| MLKFGAYIVD | GLRLYEQPIL | IYIPPCAELR | GGSWVVLDST | INPLCIEMYA | DKESRGGVLE |
| 2230 | 2240 | 2250 | 2260 | 2270 | 2280 |
| PEGTVEIKFR | KKDLVKTIRR | IDPVCKKLVG | QLGKAQLPDK | DRKELEGQLK | AREELLLPIY |
| 2290 | 2300 | 2310 | 2320 | 2330 | 2340 |
| HQVAVQFADL | HDTPGHMLEK | GIISDVLEWK | TARTFFYWRL | RRLLLEAQVK | QEILRASPEL |
| 2350 | 2360 | 2370 | 2380 | 2390 | 2400 |
| NHEHTQSMLR | RWFVETEGAV | KAYLWDSNQV | VVQWLEQHWS | AKDGLRSTIR | ENINYLKRDS |
| 2410 | 2420 | 2430 | 2440 | ||
| VLKTIQSLVQ | EHPEVIMDCV | AYLSQHLTPA | ERIQVAQLLS | TTESPASS |