Q9SUE7
Gene name |
ATX4 (SDG16, SET16, TX4, At4g27910, T13J8.20) |
Protein name |
Histone-lysine N-methyltransferase ATX4 |
Names |
Protein SET DOMAIN GROUP 16, Trithorax-homolog protein 4, TRX-homolog protein 4, Trithorax 4 |
Species |
Arabidopsis thaliana (Mouse-ear cress) |
KEGG Pathway |
ath:AT4G27910 |
EC number |
|
Protein Class |
|
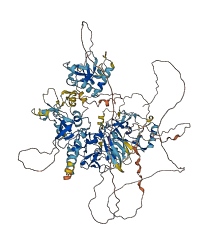
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q9SUE7
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q9SUE7-F1 | Predicted | AlphaFoldDB |
47 variants for Q9SUE7
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| tmp_4_13894722_A_G | 10 | Q>R | No | 1000Genomes | |
| tmp_4_13894899_C_T | 69 | T>I | No | 1000Genomes | |
| ENSVATH12268846 | 71 | P>S | No | 1000Genomes | |
| tmp_4_13894907_G_A | 72 | V>I | No | 1000Genomes | |
| tmp_4_13894913_G_C | 74 | V>L | No | 1000Genomes | |
| ENSVATH14304444 | 78 | L>F | No | 1000Genomes | |
| ENSVATH00542038 | 80 | K>T | No | 1000Genomes | |
| ENSVATH06788012 | 83 | S>F | No | 1000Genomes | |
| ENSVATH06788013 | 87 | T>P | No | 1000Genomes | |
| ENSVATH06788014 | 94 | A>P | No | 1000Genomes | |
| tmp_4_13895130_T_A | 146 | V>D | No | 1000Genomes | |
| ENSVATH00542039 | 150 | R>Q | No | 1000Genomes | |
| ENSVATH12268847 | 160 | K>N | No | 1000Genomes | |
| tmp_4_13895206_G_T | 171 | L>F | No | 1000Genomes | |
| tmp_4_13895207_T_C | 172 | C>R | No | 1000Genomes | |
| ENSVATH00542040 | 179 | E>V | No | 1000Genomes | |
| tmp_4_13895250_G_A | 186 | R>H | No | 1000Genomes | |
| tmp_4_13895354_T_A | 221 | F>I | No | 1000Genomes | |
| tmp_4_13895411_T_G | 240 | S>A | No | 1000Genomes | |
| ENSVATH06788015 | 281 | Q>L | No | 1000Genomes | |
| ENSVATH12268850 | 317 | H>Y | No | 1000Genomes | |
| tmp_4_13895841_G_A | 331 | R>K | No | 1000Genomes | |
| tmp_4_13896016_C_A | 352 | L>M | No | 1000Genomes | |
| ENSVATH02933680 | 356 | H>L | No | 1000Genomes | |
| ENSVATH06788018 | 367 | T>I | No | 1000Genomes | |
| tmp_4_13896068_T_A | 369 | I>N | No | 1000Genomes | |
| ENSVATH14304447 | 376 | K>I | No | 1000Genomes | |
| ENSVATH06788019 | 384 | D>N | No | 1000Genomes | |
| ENSVATH06788020 | 413 | N>K | No | 1000Genomes | |
| ENSVATH06788024 | 433 | I>K | No | 1000Genomes | |
| ENSVATH14304448 | 444 | T>P | No | 1000Genomes | |
| ENSVATH06788029 | 489 | A>T | No | 1000Genomes | |
| tmp_4_13897024_A_C | 512 | K>T | No | 1000Genomes | |
| tmp_4_13897108_A_T | 540 | K>M | No | 1000Genomes | |
| ENSVATH12268889 | 550 | L>I | No | 1000Genomes | |
| tmp_4_13897959_A_T | 645 | I>F | No | 1000Genomes | |
| ENSVATH00542044 | 647 | R>Q | No | 1000Genomes | |
| tmp_4_13898736_T_A | 755 | S>T | No | 1000Genomes | |
| tmp_4_13898867_G_A | 768 | V>M | No | 1000Genomes | |
| tmp_4_13898881_A_T | 772 | Q>H | No | 1000Genomes | |
| ENSVATH06788050 | 798 | I>V | No | 1000Genomes | |
| ENSVATH12268894 | 821 | R>L | No | 1000Genomes | |
| tmp_4_13899036_A_T | 824 | K>I | No | 1000Genomes | |
| tmp_4_13899151_G_A | 835 | E>K | No | 1000Genomes | |
| ENSVATH02933688 | 851 | A>P | No | 1000Genomes | |
| ENSVATH02933688 | 851 | A>T | No | 1000Genomes | |
| ENSVATH06788053 | 852 | A>G | No | 1000Genomes |
No associated diseases with Q9SUE7
12 regional properties for Q9SUE7
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | PWWP domain | 207 - 301 | IPR000313 |
| domain | SET domain | 885 - 1008 | IPR001214 |
| domain | Zinc finger, PHD-type | 400 - 452 | IPR001965-1 |
| domain | Zinc finger, PHD-type | 594 - 641 | IPR001965-2 |
| domain | Zinc finger, PHD-type | 705 - 761 | IPR001965-3 |
| domain | Post-SET domain | 1011 - 1027 | IPR003616 |
| conserved_site | Zinc finger, PHD-type, conserved site | 595 - 640 | IPR019786 |
| domain | Zinc finger, PHD-finger | 398 - 454 | IPR019787-1 |
| domain | Zinc finger, PHD-finger | 592 - 643 | IPR019787-2 |
| domain | Extended PHD (ePHD) domain | 646 - 761 | IPR034732 |
| domain | ATX3/4/5, ePHD domain | 649 - 760 | IPR041955 |
| domain | ATX3/4/5, PHD domain | 594 - 640 | IPR042011 |
2 GO annotations of cellular component
| Name | Definition |
|---|---|
| Ino80 complex | A multisubunit protein complex that contains the Ino80p ATPase; exhibits chromatin remodeling activity. |
| Set1C/COMPASS complex | A conserved protein complex that catalyzes methylation of histone H3. In Saccharomyces the complex contains Shg1p, Sdc1p, Swd1p, Swd2p, Swd3p, Spp1p, Bre2p, and the trithorax-related Set1p; in mammals it contains the catalytic subunit (SETD1A or SETD1B), WDR5, WDR82, RBBP5, ASH2L/ASH2, CXXC1/CFP1, HCFC1 and DPY30. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| histone-lysine N-methyltransferase activity | Catalysis of the reaction: S-adenosyl-L-methionine + histone L-lysine = S-adenosyl-L-homocysteine + histone N6-methyl-L-lysine. The methylation of peptidyl-lysine in histones forms N6-methyl-L-lysine, N6,N6-dimethyl-L-lysine and N6,N6,N6-trimethyl-L-lysine derivatives. |
| metal ion binding | Binding to a metal ion. |
3 GO annotations of biological process
| Name | Definition |
|---|---|
| chromatin organization | The assembly or remodeling of chromatin composed of DNA complexed with histones, other associated proteins, and sometimes RNA. |
| positive regulation of histone H3-K4 methylation | Any process that activates or increases the frequency, rate or extent of the covalent addition of a methyl group to the lysine at position 4 of histone H3. |
| regulation of transcription by RNA polymerase II | Any process that modulates the frequency, rate or extent of transcription mediated by RNA polymerase II. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MIIKRKFKTQ | IPSLERCKLG | NESRKKKRKL | NLGGGGYYYP | LNLLGEIAAG | IVPGNGRNGF |
| 70 | 80 | 90 | 100 | 110 | 120 |
| SASWCTEVTK | PVEVEESLSK | RRSDSGTVRD | SPPAEVSRPP | LVRTSRGRIQ | VLPSRFNDSV |
| 130 | 140 | 150 | 160 | 170 | 180 |
| LDNWRKDSKS | DCDLEEEEIE | CRNEKVVSFR | VPKATNLKSK | ELDRKSKYSA | LCKEERFHEQ |
| 190 | 200 | 210 | 220 | 230 | 240 |
| HNDEARARVD | EKLPNKKGTF | GPENFYSGDL | VWAKSGRNEP | FWPAIVIDPM | TQAPELVLRS |
| 250 | 260 | 270 | 280 | 290 | 300 |
| CIPDAACVVF | FGHSGNENER | DYAWVRRGMI | FPFVDYVARF | QEQPELQGCK | PGNFQMALEE |
| 310 | 320 | 330 | 340 | 350 | 360 |
| AFLADQGFTE | KLMHDIHLAA | GNSTFDDSFY | RWIQETAVSN | QELNNNAPRQ | GLLKKHRNPL |
| 370 | 380 | 390 | 400 | 410 | 420 |
| ACAGCETVIS | FEMAKKMKDL | IPGDQLLCKP | CSRLTKSKHI | CGICKKIRNH | LDNKSWVRCD |
| 430 | 440 | 450 | 460 | 470 | 480 |
| GCKVRIHAEC | DQISDRHLKD | LRETDYYCPT | CRAKFNFDLS | DSEKQNSKSK | VAKGDGQMVL |
| 490 | 500 | 510 | 520 | 530 | 540 |
| PDKVIVVCAG | VEGVYFPRLH | LVVCKCGSCG | PKKKALSEWE | RHTGSKSKNW | KTSVKVKSSK |
| 550 | 560 | 570 | 580 | 590 | 600 |
| LALEDWMMNL | AELHANATAA | KVPKRPSIKQ | RKQRLLAFLS | ETYEPVNAKW | TTERCAVCRW |
| 610 | 620 | 630 | 640 | 650 | 660 |
| VEDWDYNKII | ICNRCQIAVH | QECYGARHVR | DFTSWVCKAC | ERPDIKRECC | LCPVKGGALK |
| 670 | 680 | 690 | 700 | 710 | 720 |
| PTDVETLWVH | VTCAWFQPEV | CFASEEKMEP | AVGILSIPST | NFVKICVICK | QIHGSCTQCC |
| 730 | 740 | 750 | 760 | 770 | 780 |
| KCSTYYHAMC | ASRAGYRMEL | HCLEKNGQQI | TKMVSYCAYH | RAPNPDNVLI | IQTPSGAFSA |
| 790 | 800 | 810 | 820 | 830 | 840 |
| KSLVQNKKKG | GSRLISLIRE | DDEAPAENTI | TCDPFSAARC | RVFKRKINSK | KRIEEEAIPH |
| 850 | 860 | 870 | 880 | 890 | 900 |
| HTRGPRHHAS | AAIQTLNTFR | HVPEEPKSFS | SFRERLHHLQ | RTEMDRVCFG | RSGIHGWGLF |
| 910 | 920 | 930 | 940 | 950 | 960 |
| ARRNIQEGEM | VLEYRGEQVR | GSIADLREAR | YRRVGKDCYL | FKISEEVVVD | ATDKGNIARL |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| INHSCTPNCY | ARIMSVGDEE | SRIVLIAKAN | VAVGEELTYD | YLFDPDEAEE | LKVPCLCKAP |
| NCRKFMN |