Q9DBY8
Gene name |
Nvl |
Protein name |
Nuclear valosin-containing protein-like |
Names |
NVLp, Nuclear VCP-like protein |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:67459 |
EC number |
|
Protein Class |
|
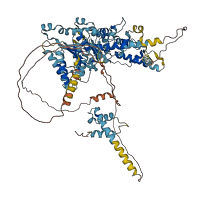
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
2 structures for Q9DBY8
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| 2RRE | NMR | - | A | 1-74 | PDB |
| AF-Q9DBY8-F1 | Predicted | AlphaFoldDB |
46 variants for Q9DBY8
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs259359459 | 6 | G>A | No | EVA | |
| rs3388523033 | 7 | V>I | No | EVA | |
| rs3388523074 | 16 | R>G | No | EVA | |
| rs3388520377 | 65 | I>K | No | EVA | |
| rs3388520358 | 68 | S>I | No | EVA | |
| rs238546158 | 76 | K>R | No | EVA | |
| rs3388524330 | 91 | E>D | No | EVA | |
| rs218298034 | 96 | T>P | No | EVA | |
| rs3388523417 | 99 | Y>N | No | EVA | |
| rs32753958 | 106 | M>I | No | EVA | |
| rs258452003 | 113 | Q>R | No | EVA | |
| rs256028156 | 117 | P>H | No | EVA | |
| rs248706985 | 128 | R>K | No | EVA | |
| rs259710695 | 132 | E>D | No | EVA | |
| rs234274508 | 136 | T>S | No | EVA | |
| rs220574822 | 137 | T>A | No | EVA | |
| rs251354052 | 140 | W>L | No | EVA | |
| rs230922114 | 141 | G>E | No | EVA | |
| rs3391088571 | 146 | T>P | No | EVA | |
| rs245989955 | 157 | G>D | No | EVA | |
| rs226707733 | 159 | V>M | No | EVA | |
| rs3388522470 | 170 | G>R | No | EVA | |
| rs3388518282 | 182 | K>E | No | EVA | |
| rs3388516121 | 246 | Q>H | No | EVA | |
| rs3388523442 | 248 | K>R | No | EVA | |
| rs3388522052 | 262 | K>N | No | EVA | |
| rs3388523020 | 266 | V>A | No | EVA | |
| rs3391115277 | 301 | L>P | No | EVA | |
| rs3388522484 | 313 | L>H | No | EVA | |
| rs3388522487 | 327 | K>R | No | EVA | |
| rs32754698 | 351 | Q>H | No | EVA | |
| rs215346488 | 374 | V>I | No | EVA | |
| rs265482374 | 402 | R>Q | No | EVA | |
| rs51443741 | 476 | L>F | No | EVA | |
| rs3388516528 | 478 | R>Q | No | EVA | |
| rs3388521966 | 490 | M>K | No | EVA | |
| rs32753816 | 513 | E>K | No | EVA | |
| rs3388524289 | 529 | R>S | No | EVA | |
| rs3388518334 | 573 | T>I | No | EVA | |
| rs3413052871 | 606 | F>V | No | EVA | |
| rs3388518531 | 748 | P>L | No | EVA | |
| rs3388524332 | 760 | I>T | No | EVA | |
| rs3388522574 | 772 | D>V | No | EVA | |
| rs3388522907 | 775 | L>M | No | EVA | |
| rs3388518280 | 776 | E>D | No | EVA | |
| rs32751966 | 844 | V>M | No | EVA |
No associated diseases with Q9DBY8
9 regional properties for Q9DBY8
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | AAA+ ATPase domain | 296 - 435 | IPR003593-1 |
| domain | AAA+ ATPase domain | 613 - 749 | IPR003593-2 |
| domain | ATPase, AAA-type, core | 300 - 430 | IPR003959-1 |
| domain | ATPase, AAA-type, core | 617 - 746 | IPR003959-2 |
| conserved_site | ATPase, AAA-type, conserved site | 403 - 421 | IPR003960-1 |
| conserved_site | ATPase, AAA-type, conserved site | 717 - 735 | IPR003960-2 |
| domain | NVL2, nucleolin binding domain | 2 - 71 | IPR031996 |
| domain | AAA ATPase, AAA+ lid domain | 460 - 489 | IPR041569-1 |
| domain | AAA ATPase, AAA+ lid domain | 772 - 828 | IPR041569-2 |
5 GO annotations of cellular component
| Name | Definition |
|---|---|
| nuclear exosome (RNase complex) | A ribonuclease complex that has 3-prime to 5-prime processive and distributive hydrolytic exoribonuclease activity and endoribonuclease activity, producing 5-prime-phosphomonoesters. Participates in a multitude of cellular RNA processing and degradation events preventing nuclear export and/or translation of aberrant RNAs. Restricted to processing linear and circular single-stranded RNAs (ssRNA) only. RNAs with complex secondary structures may have to be unwound or pre-processed by co-factors prior to entering the complex, esp if the 3-prime end is structured. |
| nucleolus | A small, dense body one or more of which are present in the nucleus of eukaryotic cells. It is rich in RNA and protein, is not bounded by a limiting membrane, and is not seen during mitosis. Its prime function is the transcription of the nucleolar DNA into 45S ribosomal-precursor RNA, the processing of this RNA into 5.8S, 18S, and 28S components of ribosomal RNA, and the association of these components with 5S RNA and proteins synthesized outside the nucleolus. This association results in the formation of ribonucleoprotein precursors; these pass into the cytoplasm and mature into the 40S and 60S subunits of the ribosome. |
| nucleoplasm | That part of the nuclear content other than the chromosomes or the nucleolus. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
| telomerase holoenzyme complex | Telomerase is a ribonucleoprotein enzyme complex, with a minimal catalytic core composed of a catalytic reverse transcriptase subunit and an RNA subunit that provides the template for telomeric DNA addition. In vivo, the holoenzyme complex often contains additional subunits. |
3 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP hydrolysis activity | Catalysis of the reaction: ATP + H2O = ADP + H+ phosphate. ATP hydrolysis is used in some reactions as an energy source, for example to catalyze a reaction or drive transport against a concentration gradient. |
| preribosome binding | Binding to a preribosome. |
6 GO annotations of biological process
| Name | Definition |
|---|---|
| positive regulation of protein binding | Any process that activates or increases the frequency, rate or extent of protein binding. |
| positive regulation of telomerase activity | Any process that activates or increases the frequency, rate or extent of telomerase activity, the catalysis of the reaction: deoxynucleoside triphosphate + DNA(n) = diphosphate + DNA(n+1). |
| regulation of protein localization to nucleolus | Any process that modulates the frequency, rate or extent of protein localization to nucleolus. |
| ribosomal large subunit biogenesis | A cellular process that results in the biosynthesis of constituent macromolecules, assembly, and arrangement of constituent parts of a large ribosomal subunit; includes transport to the sites of protein synthesis. |
| ribosome biogenesis | A cellular process that results in the biosynthesis of constituent macromolecules, assembly, and arrangement of constituent parts of ribosome subunits; includes transport to the sites of protein synthesis. |
| rRNA processing | Any process involved in the conversion of a primary ribosomal RNA (rRNA) transcript into one or more mature rRNA molecules. |
1 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| O15381 | NVL | Nuclear valosin-containing protein-like | Homo sapiens (Human) | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MKPRPGVFVD | RKLKQRVIQY | LSSNRCGKYV | DTGILASDLQ | RLYSVDYGRR | KRNAFRIQVE |
| 70 | 80 | 90 | 100 | 110 | 120 |
| KVFSIISSEK | ELKNLKELED | GHLAKRARQD | EEDEYTESYS | DDDSNMEDYP | DPQSANPMNS |
| 130 | 140 | 150 | 160 | 170 | 180 |
| SLLSLYRRGN | SESVSTTPKW | GQREATTSTP | LLTSKTGSVP | LKTPARESEG | GWFIDKTPGG |
| 190 | 200 | 210 | 220 | 230 | 240 |
| KKESLPLDLS | DDQSNSKKQD | SEIQILKDSS | LLESDKKRKG | RAKGKGNKRK | TENLQEVDGE |
| 250 | 260 | 270 | 280 | 290 | 300 |
| IEALLQKKAK | ARSTELQISN | VKFEDVGGND | ATLKEVCKML | IHMRHPEVYQ | HLGVVPPRGV |
| 310 | 320 | 330 | 340 | 350 | 360 |
| LLHGPPGCGK | TLLAHAIAGE | LDLPILKVAA | PEIVSGVSGE | SEQKLRELFD | QAVSNAPCIV |
| 370 | 380 | 390 | 400 | 410 | 420 |
| FIDEIDAITP | KREVASKDME | RRIVAQLLTC | MDDLNNVAAT | ARVLVIGATN | RPDSLDPALR |
| 430 | 440 | 450 | 460 | 470 | 480 |
| RAGRFDREVC | LGIPDEAARE | RILQTLCRKL | RLPETFNFCH | LAHLTPGFVG | ADLMALCREA |
| 490 | 500 | 510 | 520 | 530 | 540 |
| AMCAVNRVLM | KQQAQQKKKP | EIEGLPSEGD | QEERLGAEPT | SETQDELQRL | LGLLRDQDPL |
| 550 | 560 | 570 | 580 | 590 | 600 |
| SEEQMQGLCI | ELNDFIVALA | EVQPSAKREG | FVTVPNVTWA | DIGALEDIRD | ELIMAILAPV |
| 610 | 620 | 630 | 640 | 650 | 660 |
| RNPDQFRTLG | LGTPAGILLA | GPPGCGKTLL | AKAVANESGL | NFISVKGPEL | LNMYVGESER |
| 670 | 680 | 690 | 700 | 710 | 720 |
| AVRQVFQRAK | NSAPCVIFFD | EVDALCPRRS | DRETGASVRV | VNQLLTEMDG | LETRQQVFIL |
| 730 | 740 | 750 | 760 | 770 | 780 |
| AATNRPDIID | PAILRPGRLD | KTLFVGLPPP | ADRVAILKTI | TKNGTKPPLD | EDVNLETIAN |
| 790 | 800 | 810 | 820 | 830 | 840 |
| DLRCNCYTGA | DLTALVREAS | LCALRQEITA | QKNGVGAGEL | KVSHKHFEDA | FKKVKPSISI |
| 850 | |||||
| KDQVMYEALQ | RSLSQ |