Q8K2I9
Gene name |
Fbh1 |
Protein name |
F-box DNA helicase 1 |
Names |
F-box only protein 18 |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:50755 |
EC number |
5.6.2.4: Enzymes altering nucleic acid conformation |
Protein Class |
|
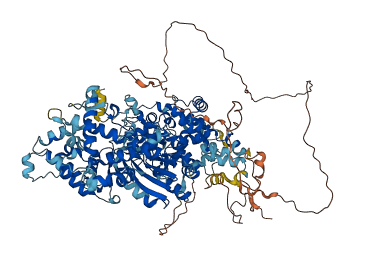
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q8K2I9
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q8K2I9-F1 | Predicted | AlphaFoldDB |
73 variants for Q8K2I9
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs3388530203 | 2 | R>S | No | EVA | |
| rs27099273 | 15 | H>Q | No | EVA | |
| rs3388529991 | 51 | N>D | No | EVA | |
| rs3388529645 | 52 | R>G | No | EVA | |
| rs3388523522 | 57 | Q>R | No | EVA | |
| rs3410289568 | 68 | H>L | No | EVA | |
| rs3391264155 | 81 | V>F | No | EVA | |
| rs27099278 | 88 | D>E | No | EVA | |
| rs242637718 | 89 | A>S | No | EVA | |
| rs235196652 | 91 | G>S | No | EVA | |
| rs3388531245 | 104 | P>S | No | EVA | |
| rs3388528105 | 133 | T>I | No | EVA | |
| rs3388526758 | 134 | E>V | No | EVA | |
| rs3388527715 | 136 | G>D | No | EVA | |
| rs3388530015 | 137 | Q>R | No | EVA | |
| rs3388531246 | 146 | P>L | No | EVA | |
| rs3388526867 | 176 | G>R | No | EVA | |
| rs3388531232 | 188 | D>V | No | EVA | |
| rs3388530036 | 212 | R>S | No | EVA | |
| rs3388528084 | 216 | E>V | No | EVA | |
| rs3388530222 | 232 | W>C | No | EVA | |
| rs3413020318 | 238 | C>F | No | EVA | |
| rs3388527819 | 241 | W>* | No | EVA | |
| rs3388527788 | 252 | P>S | No | EVA | |
| rs3388530010 | 255 | K>* | No | EVA | |
| rs3388527802 | 297 | T>I | No | EVA | |
| rs3388528074 | 303 | S>N | No | EVA | |
| rs3388526868 | 307 | E>V | No | EVA | |
| rs3388524819 | 308 | R>S | No | EVA | |
| rs3388526824 | 310 | L>V | No | EVA | |
| rs3391316588 | 361 | H>Q | No | EVA | |
| rs3391025937 | 362 | L>M | No | EVA | |
| rs244562379 | 369 | P>A | No | EVA | |
| rs3388526767 | 370 | S>R | No | EVA | |
| rs27099293 | 376 | P>A | No | EVA | |
| rs3388527734 | 456 | Q>* | No | EVA | |
| rs3391261756 | 472 | L>L* | No | EVA | |
| rs3391261740 | 510 | F>L | No | EVA | |
| rs3391251617 | 512 | S>C | No | EVA | |
| rs260011459 | 539 | N>S | No | EVA | |
| rs3388527996 | 565 | S>T | No | EVA | |
| rs3388525820 | 578 | W>* | No | EVA | |
| rs234068681 | 582 | S>N | No | EVA | |
| rs216353905 | 583 | H>Q | No | EVA | |
| rs3388527761 | 599 | L>I | No | EVA | |
| rs3388529667 | 604 | L>F | No | EVA | |
| rs3388526835 | 611 | L>* | No | EVA | |
| rs3388526835 | 612 | G>* | No | EVA | |
| rs3388526739 | 616 | E>K | No | EVA | |
| rs3388529607 | 635 | P>H | No | EVA | |
| rs27099313 | 638 | A>S | No | EVA | |
| rs3388530164 | 639 | S>P | No | EVA | |
| rs3388527704 | 678 | T>A | No | EVA | |
| rs3388530159 | 712 | A>V | No | EVA | |
| rs3388531216 | 722 | R>S | No | EVA | |
| rs3391138552 | 726 | L>S | No | EVA | |
| rs3388530611 | 727 | V>F | No | EVA | |
| rs256686703 | 739 | I>V | No | EVA | |
| rs3388529597 | 748 | R>K | No | EVA | |
| rs3388527969 | 756 | E>D | No | EVA | |
| rs3388527661 | 770 | H>Q | No | EVA | |
| rs3388524796 | 779 | G>R | No | EVA | |
| rs3388527940 | 833 | E>* | No | EVA | |
| rs3388530156 | 834 | A>G | No | EVA | |
| rs3388526842 | 836 | I>F | No | EVA | |
| rs3388530212 | 846 | I>S | No | EVA | |
| rs3388530595 | 849 | L>P | No | EVA | |
| rs3391261776 | 864 | A>G | No | EVA | |
| rs3388525846 | 895 | R>K | No | EVA | |
| rs220727637 | 899 | A>P | No | EVA | |
| rs253306730 | 903 | H>Q | No | EVA | |
| rs259628099 | 927 | R>Q | No | EVA | |
| rs3388529660 | 1021 | A>S | No | EVA |
No associated diseases with Q8K2I9
Functions
| Description | ||
|---|---|---|
| EC Number | 5.6.2.4 | Enzymes altering nucleic acid conformation |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| chromatin | The ordered and organized complex of DNA, protein, and sometimes RNA, that forms the chromosome. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
| SCF ubiquitin ligase complex | A ubiquitin ligase complex in which a cullin from the Cul1 subfamily and a RING domain protein form the catalytic core; substrate specificity is conferred by a Skp1 adaptor and an F-box protein. SCF complexes are involved in targeting proteins for degradation by the proteasome. The best characterized complexes are those from yeast and mammals (with core subunits named Cdc53/Cul1, Rbx1/Hrt1/Roc1). |
7 GO annotations of molecular function
| Name | Definition |
|---|---|
| 3'-5' DNA helicase activity | Unwinding a DNA helix in the direction 5' to 3', driven by ATP hydrolysis. |
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP hydrolysis activity | Catalysis of the reaction: ATP + H2O = ADP + H+ phosphate. ATP hydrolysis is used in some reactions as an energy source, for example to catalyze a reaction or drive transport against a concentration gradient. |
| DNA helicase activity | Unwinding of a DNA helix, driven by ATP hydrolysis. |
| DNA translocase activity | Generation of movement along a single- or double-stranded DNA molecule, driven by ATP hydrolysis. |
| double-stranded DNA binding | Binding to double-stranded DNA. |
| single-stranded DNA binding | Binding to single-stranded DNA. |
13 GO annotations of biological process
| Name | Definition |
|---|---|
| cell death | Any biological process that results in permanent cessation of all vital functions of a cell. A cell should be considered dead when any one of the following molecular or morphological criteria is met: (1) the cell has lost the integrity of its plasma membrane; (2) the cell, including its nucleus, has undergone complete fragmentation into discrete bodies (frequently referred to as apoptotic bodies). The cell corpse (or its fragments) may be engulfed by an adjacent cell in vivo, but engulfment of whole cells should not be considered a strict criteria to define cell death as, under some circumstances, live engulfed cells can be released from phagosomes (see PMID:18045538). |
| cellular response to DNA damage stimulus | Any process that results in a change in state or activity of a cell (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of a stimulus indicating damage to its DNA from environmental insults or errors during metabolism. |
| DNA catabolic process, endonucleolytic | The chemical reactions and pathways resulting in the breakdown of DNA, involving the hydrolysis of internal 3',5'-phosphodiester bonds in one or two strands of deoxyribonucleotides. |
| double-strand break repair via homologous recombination | The error-free repair of a double-strand break in DNA in which the broken DNA molecule is repaired using homologous sequences. A strand in the broken DNA searches for a homologous region in an intact chromosome to serve as the template for DNA synthesis. The restoration of two intact DNA molecules results in the exchange, reciprocal or nonreciprocal, of genetic material between the intact DNA molecule and the broken DNA molecule. |
| negative regulation of chromatin binding | Any process that stops or reduces the frequency, rate or extent of chromatin binding. Chromatin binding is the selective interaction with chromatin, the network of fibers of DNA, protein, and sometimes RNA, that make up the chromosomes of the eukaryotic nucleus during interphase. |
| negative regulation of double-strand break repair via homologous recombination | Any process that stops, prevents, or reduces the frequency, rate or extent of double-strand break repair via homologous recombination. |
| positive regulation of intrinsic apoptotic signaling pathway in response to DNA damage | Any process that activates or increases the frequency, rate or extent of intrinsic apoptotic signaling pathway in response to DNA damage. |
| positive regulation of protein phosphorylation | Any process that activates or increases the frequency, rate or extent of addition of phosphate groups to amino acids within a protein. |
| protein ubiquitination | The process in which one or more ubiquitin groups are added to a protein. |
| recombinational repair | A DNA repair process that involves the exchange, reciprocal or nonreciprocal, of genetic material between the broken DNA molecule and a homologous DNA region. |
| replication fork processing | The process in which a DNA replication fork that has stalled is restored to a functional state and replication is restarted. The stalling may be due to DNA damage, DNA secondary structure, bound proteins, dNTP shortage, or other causes. |
| replication fork protection | Any process that prevents the collapse of stalled replication forks. |
| response to intra-S DNA damage checkpoint signaling | A process that occurs in response to signals generated as a result of intra-S DNA damage checkpoint signaling. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MRRFKRKHLT | VVDCHHLARS | HLAVTQPFSQ | RWTNRDPNHG | LYPRPRTKGR | NRGRGCQRYI |
| 70 | 80 | 90 | 100 | 110 | 120 |
| SEFFLAGHQH | CTNDMAKSNS | VGQDSCQDAE | GDMILTAESS | CTLPQVDNGE | ARLGSSGSAQ |
| 130 | 140 | 150 | 160 | 170 | 180 |
| PARKRAHCFE | EATESGQWDG | VTKKTPRHRL | FPSCSRLREA | RQGAEDSLSQ | CSPVPGEAGR |
| 190 | 200 | 210 | 220 | 230 | 240 |
| DIEDIGPDPL | PDSYYGLLGM | LPCQEVPSHI | CRLPSEVLRH | IFAFLPVEDL | YWNLSLVCHL |
| 250 | 260 | 270 | 280 | 290 | 300 |
| WREIINDPLF | IPWKKLYHRY | LINEEQAVSK | VDGILSSHGI | EKDSDLCVLN | LIRYTATTKC |
| 310 | 320 | 330 | 340 | 350 | 360 |
| SPSVDPERVL | WSLRDHPLLL | EAEACMRQQL | PDLYAAAGGI | NVWALVAAMV | LLSSCVNDIQ |
| 370 | 380 | 390 | 400 | 410 | 420 |
| HLLFCLRRPS | STVTMPDVTE | TLYCIAVLLY | AMREKGINIS | NRIHYNIFYC | LYLQENSCTQ |
| 430 | 440 | 450 | 460 | 470 | 480 |
| ATKVTEEPSV | WPGKKTSIQL | THEQQLILNH | KMEPLQVVKI | MAFAGTGKTS | TLVKYAEKWS |
| 490 | 500 | 510 | 520 | 530 | 540 |
| QSRFLYVTFN | KSIAKQAELV | FPSNVICKTF | HSMAYSHVGR | KYQLKKKLNL | FKLTPFMVNS |
| 550 | 560 | 570 | 580 | 590 | 600 |
| VLAEGKGGFI | RAKLVCKTLE | NFFASADEEL | TIDHVPIWCK | NSHGQRVMVE | QSEKLNGVLE |
| 610 | 620 | 630 | 640 | 650 | 660 |
| ASRLWDNMRK | LGECKEEAYQ | MTHDGYLKLW | QLSKPLLASF | DAIFVDEAQD | CTPAIMNIVL |
| 670 | 680 | 690 | 700 | 710 | 720 |
| SQPCGKIFVG | DPHQQIYTFR | GAVNALFTVP | HTHVFYLTQS | FRFGVEIAYV | GATILDVCKR |
| 730 | 740 | 750 | 760 | 770 | 780 |
| VRKKTLVGGN | HQSGIRGDIK | GQVALLSRTN | ANVFDEAVRV | TEGESPARIH | LIGGIKSFGL |
| 790 | 800 | 810 | 820 | 830 | 840 |
| DRIIDIWTLL | QPEEERRKRD | LIIKDRFIRR | WVHKEGFSGF | KRYVTAAEDK | ELEAKIAVVE |
| 850 | 860 | 870 | 880 | 890 | 900 |
| KYNIRIPELV | ERIERCHIDD | LDFAEYILGT | VHKAKGLEFD | TVHVLDDFVK | VPCARHNLAQ |
| 910 | 920 | 930 | 940 | 950 | 960 |
| LPHFRVESFS | EDEWNLLYVA | VTRAKKRLIM | TKSLENILTL | AGEYFLQAEL | TSNVLKTGVV |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| HCCVGQCNNT | IPVDTILTMK | KLPITYSNRK | ENKGGYLCHS | CAEQRIGPLA | FLTASPEQVR |
| 1030 | 1040 | ||||
| AMERTVEDIV | LPRQEALLFL | VF |