Q8JZQ9
Gene name |
Eif3b (Eif3s9) |
Protein name |
Eukaryotic translation initiation factor 3 subunit B |
Names |
eIF3b, Eukaryotic translation initiation factor 3 subunit 9, eIF-3-eta, eIF3 p116 |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:27979 |
EC number |
|
Protein Class |
|
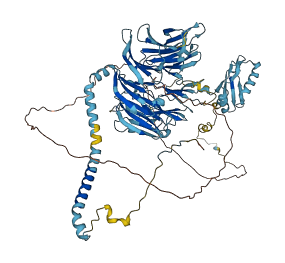
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q8JZQ9
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q8JZQ9-F1 | Predicted | AlphaFoldDB |
33 variants for Q8JZQ9
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs13464234 | 25 | A>V | No | EVA | |
| rs214415308 | 32 | D>E | No | EVA | |
| rs250468613 | 55 | G>R | No | EVA | |
| rs220537639 | 59 | E>D | No | EVA | |
| rs251559509 | 76 | P>S | No | EVA | |
| rs260435418 | 78 | A>T | No | EVA | |
| rs239545417 | 84 | S>L | No | EVA | |
| rs3388804747 | 168 | E>K | No | EVA | |
| rs3388799161 | 192 | L>I | No | EVA | |
| rs3388800555 | 199 | I>N | No | EVA | |
| rs3388804819 | 217 | K>R | No | EVA | |
| rs3388793582 | 220 | G>W | No | EVA | |
| rs3388799166 | 229 | P>S | No | EVA | |
| rs3388798689 | 236 | V>M | No | EVA | |
| rs3388786158 | 260 | K>T | No | EVA | |
| rs3388804266 | 309 | W>R | No | EVA | |
| rs3388786135 | 335 | G>D | No | EVA | |
| rs3388805802 | 343 | Q>P | No | EVA | |
| rs3388799120 | 382 | P>A | No | EVA | |
| rs3388805824 | 385 | D>N | No | EVA | |
| rs3388804338 | 417 | I>N | No | EVA | |
| rs3388811284 | 420 | W>C | No | EVA | |
| rs3388789250 | 429 | R>G | No | EVA | |
| rs3413143525 | 490 | R>T | No | EVA | |
| rs3388804259 | 490 | R>TPHYLNHH* | No | EVA | |
| rs3388798776 | 562 | N>K | No | EVA | |
| rs3396356047 | 582 | H>* | No | EVA | |
| rs3388799142 | 586 | N>S | No | EVA | |
| rs3388793637 | 598 | Q>P | No | EVA | |
| rs3396359134 | 620 | M>D* | No | EVA | |
| rs3388811274 | 739 | R>W | No | EVA | |
| rs224825055 | 753 | A>T | No | EVA | |
| rs3396282101 | 795 | E>L | No | EVA |
No associated diseases with Q8JZQ9
7 regional properties for Q8JZQ9
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | FERM domain | 17 - 298 | IPR000299 |
| domain | FERM adjacent | 308 - 354 | IPR014847 |
| domain | FERM, N-terminal | 21 - 83 | IPR018979 |
| domain | FERM, C-terminal PH-like domain | 214 - 302 | IPR018980 |
| conserved_site | FERM conserved site | 71 - 100 | IPR019747 |
| domain | FERM central domain | 103 - 210 | IPR019748 |
| domain | Band 4.1 domain | 13 - 210 | IPR019749 |
6 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytoplasmic stress granule | A dense aggregation in the cytosol composed of proteins and RNAs that appear when the cell is under stress. |
| eukaryotic 43S preinitiation complex | A protein complex composed of the 40S ribosomal subunit plus eIF1A, eIF3, and eIF2-GTP-bound methionyl-initiator methionine tRNA. |
| eukaryotic 48S preinitiation complex | A protein complex composed of the small ribosomal subunit, eIF3, eIF1A, methionyl-initiatior methionine and a capped mRNA. The complex is initially positioned at the 5'-end of the capped mRNA. |
| eukaryotic translation initiation factor 3 complex | A complex of several polypeptides that plays at least two important roles in protein synthesis: First, eIF3 binds to the 40S ribosome and facilitates loading of the Met-tRNA/eIF2.GTP ternary complex to form the 43S preinitiation complex. Subsequently, eIF3 apparently assists eIF4 in recruiting mRNAs to the 43S complex. The eIF3 complex contains five conserved core subunits, and may contain several additional proteins; the non-core subunits are thought to mediate association of the complex with specific sets of mRNAs. |
| eukaryotic translation initiation factor 3 complex, eIF3m | An eukaryotic translation initiation factor 3 complex that contains the PCI-domain protein eIF3m. |
| synapse | The junction between an axon of one neuron and a dendrite of another neuron, a muscle fiber or a glial cell. As the axon approaches the synapse it enlarges into a specialized structure, the presynaptic terminal bouton, which contains mitochondria and synaptic vesicles. At the tip of the terminal bouton is the presynaptic membrane; facing it, and separated from it by a minute cleft (the synaptic cleft) is a specialized area of membrane on the receiving cell, known as the postsynaptic membrane. In response to the arrival of nerve impulses, the presynaptic terminal bouton secretes molecules of neurotransmitters into the synaptic cleft. These diffuse across the cleft and transmit the signal to the postsynaptic membrane. |
3 GO annotations of molecular function
| Name | Definition |
|---|---|
| RNA binding | Binding to an RNA molecule or a portion thereof. |
| translation initiation factor activity | Functions in the initiation of ribosome-mediated translation of mRNA into a polypeptide. |
| translation initiation factor binding | Binding to a translation initiation factor, any polypeptide factor involved in the initiation of ribosome-mediated translation. |
5 GO annotations of biological process
| Name | Definition |
|---|---|
| formation of cytoplasmic translation initiation complex | Joining of the large subunit, with release of IF2/eIF2 and IF3/eIF3. This leaves the functional ribosome at the AUG, with the methionyl/formyl-methionyl-tRNA positioned at the P site. |
| IRES-dependent viral translational initiation | Process by which viral mRNA translation is initiated, where a domain in the 5' untranslated region (UTR) of the viral mRNA called an internal ribosome entry site (IRES) binds the host 43S preinitiation complex, circumventing regular cap-dependent translation initiation. |
| regulation of translational initiation | Any process that modulates the frequency, rate or extent of translational initiation. |
| translational initiation | The process preceding formation of the peptide bond between the first two amino acids of a protein. This includes the formation of a complex of the ribosome, mRNA or circRNA, and an initiation complex that contains the first aminoacyl-tRNA. |
| viral translational termination-reinitiation | A process which occurs as part of viral mRNA translation which allows expression of a downstream open reading frame (ORF) in a dicistronic mRNA. In this process, ribosomes translate the upstream ORF but following termination, a proportion of 40S subunits remain tethered to the mRNA and go on to re-initiate translation at the start codon of the downstream ORF. |
4 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| A7MB16 | EIF3B | Eukaryotic translation initiation factor 3 subunit B | Bos taurus (Bovine) | PR |
| P55884 | EIF3B | Eukaryotic translation initiation factor 3 subunit B | Homo sapiens (Human) | PR |
| Q4G061 | Eif3b | Eukaryotic translation initiation factor 3 subunit B | Rattus norvegicus (Rat) | PR |
| Q9XWI6 | eif-3.B | Eukaryotic translation initiation factor 3 subunit B | Caenorhabditis elegans | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MQDAENVAVP | EAAEERAEPA | RQQPASESPP | TDEAAGSGGS | EVGQTEDAEE | DAEAGPEPEV |
| 70 | 80 | 90 | 100 | 110 | 120 |
| RAKPAAQSEE | ETATSPAASP | TPQSAERSPS | QEPSAPGKAE | AVGEQARGHP | SAGAEEEGGS |
| 130 | 140 | 150 | 160 | 170 | 180 |
| DGSAAEAEPR | ALENGEADEP | SFSDPEDFVD | DVSEEELLGD | VLKDRPQEAD | GIDSVIVVDN |
| 190 | 200 | 210 | 220 | 230 | 240 |
| VPQVGPDRLE | KLKNVIHKIF | SKFGKIINDY | YPEEDGKTKG | YIFLEYASPA | HAVDAVKNAD |
| 250 | 260 | 270 | 280 | 290 | 300 |
| GYKLDKQHTF | RVNLFTDFDK | YMTISDEWDI | PEKQPFKDLG | NLRYWLEEAE | CRDQYSVIFE |
| 310 | 320 | 330 | 340 | 350 | 360 |
| SGDRTSIFWN | DVKDPVSIEE | RARWTETYVR | WSPKGTYLAT | FHQRGIALWG | GDKFKQIQRF |
| 370 | 380 | 390 | 400 | 410 | 420 |
| SHQGVQLIDF | SPCERYLVTF | SPLMDTQDDP | QAIIIWDILT | GHKKRGFHCE | SSAHWPIFKW |
| 430 | 440 | 450 | 460 | 470 | 480 |
| SHDGKFFARM | TLDTLSIYET | PSMGLLDKKS | LKISGIKDFS | WSPGGNIIAF | WVPEDKDIPA |
| 490 | 500 | 510 | 520 | 530 | 540 |
| RVTLMQLPTR | QEIRVRNLFN | VVDCKLHWQK | NGDYLCVKVD | RTPKGTQGVV | TNFEIFRMRE |
| 550 | 560 | 570 | 580 | 590 | 600 |
| KQVPVDVVEM | KETIIAFAWE | PNGSKFAVLH | GEAPRISVSF | YHVKSNGKIE | LIKMFDKQQA |
| 610 | 620 | 630 | 640 | 650 | 660 |
| NTIFWSPQGQ | FVVLAGLRSM | NGALAFVDTS | DCTVMNIAEH | YMASDVEWDP | TGRYVVTSVS |
| 670 | 680 | 690 | 700 | 710 | 720 |
| WWSHKVDNAY | WLWTFQGRLL | QKNNKDRFCQ | LLWRPRPPTL | LSQDQIKQIK | KDLKKYSKIF |
| 730 | 740 | 750 | 760 | 770 | 780 |
| EQKDRLSQSK | ASKELVERRR | TMMEDFRQYR | KMAQELYMKQ | KNERLELRGG | VDTDELDSNV |
| 790 | 800 | ||||
| DDWEEETIEF | FVTEEVIPLG | SQE |