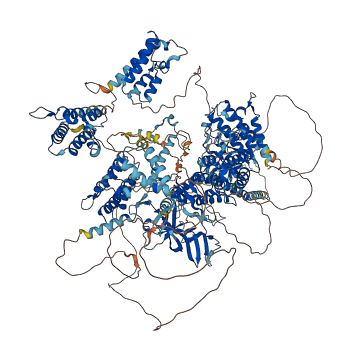
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
2 structures for Q8BSQ9
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| 2YQD | NMR | - | A | 650-762 | PDB |
| AF-Q8BSQ9-F1 | Predicted | AlphaFoldDB |
40 variants for Q8BSQ9
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs3389312127 | 53 | L>F | No | EVA | |
| rs3389241139 | 60 | Y>F | No | EVA | |
| rs3389288924 | 64 | Q>K | No | EVA | |
| rs3389306781 | 257 | K>E | No | EVA | |
| rs3389289007 | 259 | A>V | No | EVA | |
| rs3389298321 | 260 | K>N | No | EVA | |
| rs3389270403 | 387 | H>Q | No | EVA | |
| rs46367466 | 391 | D>N | No | EVA | |
| rs3389288944 | 469 | I>F | No | EVA | |
| rs3389281129 | 475 | K>R | No | EVA | |
| rs3389241132 | 492 | D>E | No | EVA | |
| rs3389281162 | 497 | D>E | No | EVA | |
| rs3389310972 | 514 | S>N | No | EVA | |
| rs241680213 | 814 | S>F | No | EVA | |
| rs3404237716 | 1110 | E>K | No | EVA | |
| rs226361707 | 1124 | N>S | No | EVA | |
| rs3404828083 | 1138 | M>R | No | EVA | |
| rs3389317237 | 1190 | Y>N | No | EVA | |
| rs3389316286 | 1222 | E>K | No | EVA | |
| rs3389288937 | 1301 | P>L | No | EVA | |
| rs3389288988 | 1307 | K>N | No | EVA | |
| rs3389312141 | 1307 | K>R | No | EVA | |
| rs3389310974 | 1323 | D>E | No | EVA | |
| rs237784946 | 1352 | E>D | No | EVA | |
| rs3405014580 | 1369 | K>* | No | EVA | |
| rs3403476304 | 1369 | K>I | No | EVA | |
| rs3405014627 | 1369 | K>N | No | EVA | |
| rs3389316272 | 1454 | S>N | No | EVA | |
| rs3389310949 | 1467 | H>Y | No | EVA | |
| rs3413105247 | 1474 | G>S | No | EVA | |
| rs3405036498 | 1476 | P>YHAVLRVLIHW* | No | EVA | |
| rs3389313994 | 1477 | G>D | No | EVA | |
| rs3389270349 | 1480 | P>L | No | EVA | |
| rs3389316334 | 1496 | A>T | No | EVA | |
| rs3389322131 | 1499 | G>R | No | EVA | |
| rs3389241167 | 1503 | G>R | No | EVA | |
| rs3389325646 | 1505 | Q>H | No | EVA | |
| rs3405099487 | 1609 | D>A | No | EVA | |
| rs3404922973 | 1609 | D>Y | No | EVA | |
| rs3404926877 | 1613 | R>C | No | EVA |
No associated diseases with Q8BSQ9
15 regional properties for Q8BSQ9
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Bromo adjacent homology (BAH) domain | 956 - 1074 | IPR001025-1 |
| domain | Bromo adjacent homology (BAH) domain | 1156 - 1272 | IPR001025-2 |
| domain | Bromodomain | 43 - 153 | IPR001487-1 |
| domain | Bromodomain | 175 - 289 | IPR001487-2 |
| domain | Bromodomain | 379 - 489 | IPR001487-3 |
| domain | Bromodomain | 516 - 627 | IPR001487-4 |
| domain | Bromodomain | 651 - 765 | IPR001487-5 |
| domain | Bromodomain | 775 - 881 | IPR001487-6 |
| domain | High mobility group box domain | 1378 - 1448 | IPR009071 |
| conserved_site | Bromodomain, conserved site | 72 - 126 | IPR018359-1 |
| conserved_site | Bromodomain, conserved site | 205 - 262 | IPR018359-2 |
| conserved_site | Bromodomain, conserved site | 405 - 462 | IPR018359-3 |
| conserved_site | Bromodomain, conserved site | 548 - 600 | IPR018359-4 |
| conserved_site | Bromodomain, conserved site | 681 - 738 | IPR018359-5 |
| domain | Protein polybromo-1, Bromodomain 5 | 658 - 762 | IPR037968 |
7 GO annotations of cellular component
| Name | Definition |
|---|---|
| chromatin | The ordered and organized complex of DNA, protein, and sometimes RNA, that forms the chromosome. |
| kinetochore | A multisubunit complex that is located at the centromeric region of DNA and provides an attachment point for the spindle microtubules. |
| nuclear matrix | The dense fibrillar network lying on the inner side of the nuclear membrane. |
| nucleoplasm | That part of the nuclear content other than the chromosomes or the nucleolus. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
| RSC-type complex | A SWI/SNF-type complex that contains a bromodomain containing-protein, such as yeast Rsc1 or Rsc4 or mammalian PB1/BAF180. The RSC complex is generally recruited to RNA polymerase III promoters and is specifically recruited to RNA polymerase II promoters by transcriptional activators and repressors; it is also involved in non-homologous end joining. |
| SWI/SNF complex | A SWI/SNF-type complex that contains 8 to 14 proteins, including both conserved (core) and nonconserved components; contains the ATPase product of the yeast SNF2 or mammalian SMARCA4/BAF190A/BRG1 gene, or an ortholog thereof. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| chromatin binding | Binding to chromatin, the network of fibers of DNA, protein, and sometimes RNA, that make up the chromosomes of the eukaryotic nucleus during interphase. |
| DNA binding | Any molecular function by which a gene product interacts selectively and non-covalently with DNA (deoxyribonucleic acid). |
21 GO annotations of biological process
| Name | Definition |
|---|---|
| blastocyst formation | The initial formation of a blastocyst from a solid ball of cells known as a morula. |
| blood vessel remodeling | The reorganization or renovation of existing blood vessels. |
| cardiac vascular smooth muscle cell development | The process whose specific outcome is the progression of a cardiac vascular smooth muscle cell over time, from its formation to the mature state. |
| chromatin remodeling | A dynamic process of chromatin reorganization resulting in changes to chromatin structure. These changes allow DNA metabolic processes such as transcriptional regulation, DNA recombination, DNA repair, and DNA replication. |
| epicardium-derived cardiac endothelial cell differentiation | The process in which an epicardial cell acquires the specialized structural and/or functional features of a cardiac endothelial cell. |
| heart development | The process whose specific outcome is the progression of the heart over time, from its formation to the mature structure. The heart is a hollow, muscular organ, which, by contracting rhythmically, keeps up the circulation of the blood. |
| heart morphogenesis | The developmental process in which the heart is generated and organized. The heart is a hollow, muscular organ, which, by contracting rhythmically, keeps up the circulation of the blood. |
| negative regulation of cell population proliferation | Any process that stops, prevents or reduces the rate or extent of cell proliferation. |
| placenta development | The process whose specific outcome is the progression of the placenta over time, from its formation to the mature structure. The placenta is an organ of metabolic interchange between fetus and mother, partly of embryonic origin and partly of maternal origin. |
| positive regulation of cell differentiation | Any process that activates or increases the frequency, rate or extent of cell differentiation. |
| positive regulation of dendritic spine development | Any process that increases the rate, frequency, or extent of dendritic spine development, the process whose specific outcome is the progression of the dendritic spine over time, from its formation to the mature structure. |
| positive regulation of DNA-templated transcription | Any process that activates or increases the frequency, rate or extent of cellular DNA-templated transcription. |
| positive regulation of double-strand break repair | Any process that activates or increases the frequency, rate or extent of double-strand break repair. |
| positive regulation of myoblast differentiation | Any process that activates or increases the frequency, rate or extent of myoblast differentiation. A myoblast is a mononucleate cell type that, by fusion with other myoblasts, gives rise to the myotubes that eventually develop into skeletal muscle fibers. |
| positive regulation of T cell differentiation | Any process that activates or increases the frequency, rate or extent of T cell differentiation. |
| regulation of G0 to G1 transition | A cell cycle process that modulates the rate or extent of the transition from the G0 quiescent state to the G1 phase. |
| regulation of G1/S transition of mitotic cell cycle | Any signalling pathway that modulates the activity of a cell cycle cyclin-dependent protein kinase to modulate the switch from G1 phase to S phase of the mitotic cell cycle. |
| regulation of mitotic metaphase/anaphase transition | Any process that modulates the frequency, rate or extent of the cell cycle process in which a cell progresses from metaphase to anaphase during mitosis, triggered by the activation of the anaphase promoting complex by Cdc20/Sleepy homolog which results in the degradation of Securin. |
| regulation of nucleotide-excision repair | Any process that modulates the frequency, rate or extent of nucleotide-excision repair. |
| regulation of transcription by RNA polymerase II | Any process that modulates the frequency, rate or extent of transcription mediated by RNA polymerase II. |
| vasculogenesis involved in coronary vascular morphogenesis | The differentiation of endothelial cells from progenitor cells that contributes to blood vessel development in the heart, and the de novo formation of blood vessels and tubes. |
1 homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| Q86U86 | PBRM1 | Protein polybromo-1 | Homo sapiens (Human) | PR |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MGSKRRRATS | PSSSVSGDFD | DGHHSVPTPG | PSRKRRRLSN | LPTVDPIAVC | HELYNTIRDY |
| 70 | 80 | 90 | 100 | 110 | 120 |
| KDEQGRLLCE | LFIRAPKRRN | QPDYYEVVSQ | PIDLMKIQQK | LKMEEYDDVN | LLTADFQLLF |
| 130 | 140 | 150 | 160 | 170 | 180 |
| NNAKAYYKPD | SPEYKAACKL | WDLYLRTRNE | FVQKGEADDE | DDDEDGQDNQ | GTLADGSSPG |
| 190 | 200 | 210 | 220 | 230 | 240 |
| YLKEILEQLL | EAIVVATNPS | GRLISELFQK | LPSKVQYPDY | YAIIKEPIDL | KTIAQRIQNG |
| 250 | 260 | 270 | 280 | 290 | 300 |
| SYKSIHAMAK | DIDLLAKNAK | TYNEPGSQVF | KDANSIKKIF | YMKKAEIEHH | EMTKSSLRIR |
| 310 | 320 | 330 | 340 | 350 | 360 |
| TASNLAAARL | TGPSHNKSSL | GEERNPTSKY | YRNKRAVQGG | RLSAITMALQ | YGSESEEDAA |
| 370 | 380 | 390 | 400 | 410 | 420 |
| LAAARYEEGE | SEAESITSFM | DVSNPFHQLY | DTVRSCRNHQ | GQLIAEPFFH | LPSKKKYPDY |
| 430 | 440 | 450 | 460 | 470 | 480 |
| YQQIKMPISL | QQIRTKLKNQ | EYETLDHLEC | DLNLMFENAK | RYNVPNSAIY | KRVLKLQQVM |
| 490 | 500 | 510 | 520 | 530 | 540 |
| QAKKKELARR | DDIEDGDSMI | SSATSDTGSA | KRKSKKNIRK | QRMKILFNVV | LEAREPGSGR |
| 550 | 560 | 570 | 580 | 590 | 600 |
| RLCDLFMVKP | SKKDYPDYYK | IILEPMDLKI | IEHNIRNDKY | AGEEGMMEDM | KLMFRNARHY |
| 610 | 620 | 630 | 640 | 650 | 660 |
| NEEGSQVYND | AHILEKLLKD | KRKELGPLPD | DDDMASPKLK | LSRKSGVSPK | KSKYMTPMQQ |
| 670 | 680 | 690 | 700 | 710 | 720 |
| KLNEVYEAVK | NYTDKRGRRL | SAIFLRLPSR | SELPDYYLTI | KKPMDMEKIR | SHMMANKYQD |
| 730 | 740 | 750 | 760 | 770 | 780 |
| IDSMVEDFVM | MFNNACTYNE | PESLIYKDAL | VLHKVLLETR | RDLEGDEDSH | VPNVTLLIQE |
| 790 | 800 | 810 | 820 | 830 | 840 |
| LIHNLFVSVM | SHQDDEGRCY | SDSLAEIPAV | DPNSPNKPPL | TFDIIRKNVE | SNRYRRLDLF |
| 850 | 860 | 870 | 880 | 890 | 900 |
| QEHMFEVLER | ARRMNRTDSE | IYEDAVELQQ | FFIRIRDELC | KNGEILLSPA | LSYTTKHLHN |
| 910 | 920 | 930 | 940 | 950 | 960 |
| DVEKEKKEKL | PKEIEEDKLK | REEEKREAEK | SEDSSGTTGL | SGLHRTYSQD | CSFKNSMYHV |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| GDYVYVEPAE | ANLQPHIVCI | ERLWEDSAGE | KWLYGCWFYR | PNETFHLATR | KFLEKEVFKS |
| 1030 | 1040 | 1050 | 1060 | 1070 | 1080 |
| DYYNKVPVSK | ILGKCVVMFV | KEYFKLCPEN | FRDEDVFVCE | SRYSAKTKSF | KKIKLWTMPI |
| 1090 | 1100 | 1110 | 1120 | 1130 | 1140 |
| SSVRFVPRDV | PLPVVRVASV | FANADKGDDE | KNTDNSDDNR | AEDNFNLEKE | KEDVPVEMSN |
| 1150 | 1160 | 1170 | 1180 | 1190 | 1200 |
| GEPGCHYFEQ | LRYNDMWLKV | GDCVFIKSHG | LVRPRVGRIE | KVWVRDGAAY | FYGPIFIHPE |
| 1210 | 1220 | 1230 | 1240 | 1250 | 1260 |
| ETEHEPTKMF | YKKEVFLSNL | EETCPMSCIL | GKCAVLSFKD | FLSCRPTEIP | ENDILLCESR |
| 1270 | 1280 | 1290 | 1300 | 1310 | 1320 |
| YNESDKQMKK | FKGLKRFSLS | AKVVDDEIYY | FRKPIIPQKE | PSPLLEKKIQ | LLEAKFAELE |
| 1330 | 1340 | 1350 | 1360 | 1370 | 1380 |
| GGDDDIEEMG | EEDSEVIEAP | SLPQLQTPLA | NELDLMPYTP | PQSTPKSAKG | SAKKESSKRK |
| 1390 | 1400 | 1410 | 1420 | 1430 | 1440 |
| INMSGYILFS | SEMRAVIKAQ | HPDYSFGELS | RLVGTEWRNL | ETAKKAEYEG | MMGGYPPGLP |
| 1450 | 1460 | 1470 | 1480 | 1490 | 1500 |
| PLQGPVDGLV | SMGSMQPLHP | GGPPPHHLPP | GVPGLPGIPP | PGVMNQGVAP | MVGTPAPGGS |
| 1510 | 1520 | 1530 | 1540 | 1550 | 1560 |
| PYGQQVGVLG | PPGQQAPPPY | PGPHPAGPPV | IQQPTTPMFV | APPPKTQRLL | HSEAYLKYIE |
| 1570 | 1580 | 1590 | 1600 | 1610 | 1620 |
| GLSAESNSIS | KWDQTLAARR | RDVHLSKEQE | SRLPSHWLKS | KGAHTTMADA | LWRLRDLMLR |
| 1630 | |||||
| DTLNIRQAYN | LENV |