Q8BIP0
Gene name |
Dars2 |
Protein name |
Aspartate--tRNA ligase, mitochondrial |
Names |
Aspartyl-tRNA synthetase, AspRS |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:226539 |
EC number |
6.1.1.12: Ligases forming aminoacyl-tRNA and related compounds |
Protein Class |
|
Descriptions
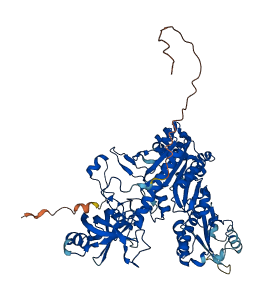
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q8BIP0
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q8BIP0-F1 | Predicted | AlphaFoldDB |
43 variants for Q8BIP0
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs246378572 | 5 | F>S | No | EVA | |
| rs51557988 | 9 | R>S | No | EVA | |
| rs3388512970 | 38 | Q>L | No | EVA | |
| rs3390872287 | 81 | V>G | No | EVA | |
| rs3388510407 | 108 | E>G | No | EVA | |
| rs3388509327 | 109 | A>G | No | EVA | |
| rs3388509401 | 110 | P>S | No | EVA | |
| rs3388507075 | 111 | V>G | No | EVA | |
| rs3388506071 | 115 | V>G | No | EVA | |
| rs3388511401 | 116 | R>S | No | EVA | |
| rs3388509788 | 117 | V>L | No | EVA | |
| rs3388509841 | 118 | S>Y | No | EVA | |
| rs3388509777 | 134 | P>* | No | EVA | |
| rs3388511337 | 134 | P>R | No | EVA | |
| rs3388509392 | 141 | K>N | No | EVA | |
| rs3388508371 | 143 | K>* | No | EVA | |
| rs3388509844 | 167 | A>* | No | EVA | |
| rs3388510848 | 167 | A>E | No | EVA | |
| rs3412833541 | 189 | R>G | No | EVA | |
| rs233525171 | 196 | M>I | No | EVA | |
| rs3388508403 | 252 | G>R | No | EVA | |
| rs3388510901 | 266 | D>G | No | EVA | |
| rs3388511430 | 304 | W>* | No | EVA | |
| rs3388508395 | 310 | P>S | No | EVA | |
| rs3388511222 | 323 | A>T | No | EVA | |
| rs229942736 | 326 | T>N | No | EVA | |
| rs3388509816 | 338 | M>V | No | EVA | |
| rs3388509825 | 346 | V>M | No | EVA | |
| rs232005332 | 352 | L>I | No | EVA | |
| rs3388509304 | 367 | K>R | No | EVA | |
| rs33754544 | 370 | C>R | No | EVA | |
| rs31573477 | 429 | M>L | No | EVA | |
| rs254984776 | 436 | I>M | No | EVA | |
| rs3388507052 | 469 | L>F | No | EVA | |
| rs3390884397 | 492 | S>C | No | EVA | |
| rs3388510906 | 500 | H>N | No | EVA | |
| rs3388510460 | 500 | H>R | No | EVA | |
| rs3388512982 | 507 | N>Y | No | EVA | |
| rs3388508566 | 529 | V>F | No | EVA | |
| rs3388510895 | 532 | G>D | No | EVA | |
| rs229027610 | 620 | V>M | No | EVA | |
| rs3388509361 | 630 | I>T | No | EVA | |
| rs246962275 | 640 | E>D | No | EVA |
No associated diseases with Q8BIP0
6 regional properties for Q8BIP0
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Aminoacyl-tRNA synthetase, class II (D/K/N) | 166 - 605 | IPR004364 |
| domain | OB-fold nucleic acid binding domain, AA-tRNA synthetase-type | 65 - 148 | IPR004365 |
| domain | Aminoacyl-tRNA synthetase, class II | 186 - 604 | IPR006195 |
| domain | GAD domain | 356 - 451 | IPR029351 |
| domain | Aspartate-tRNA ligase, type 1, anticodon recognition domain | 49 - 182 | IPR047089 |
| domain | Aspartate-tRNA ligase, type 1, core domain | 186 - 606 | IPR047090 |
Functions
| Description | ||
|---|---|---|
| EC Number | 6.1.1.12 | Ligases forming aminoacyl-tRNA and related compounds |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| mitochondrial matrix | The gel-like material, with considerable fine structure, that lies in the matrix space, or lumen, of a mitochondrion. It contains the enzymes of the tricarboxylic acid cycle and, in some organisms, the enzymes concerned with fatty acid oxidation. |
| mitochondrion | A semiautonomous, self replicating organelle that occurs in varying numbers, shapes, and sizes in the cytoplasm of virtually all eukaryotic cells. It is notably the site of tissue respiration. |
| nucleoplasm | That part of the nuclear content other than the chromosomes or the nucleolus. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| aspartate-tRNA ligase activity | Catalysis of the reaction: ATP + L-aspartate + tRNA(Asp) = AMP + diphosphate + L-aspartyl-tRNA(Asp). |
| aspartate-tRNA(Asn) ligase activity | Catalysis of the reaction: tRNA(Asx) + L-aspartate + ATP = aspartyl-tRNA(Asx) + diphosphate + AMP. |
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| nucleic acid binding | Binding to a nucleic acid. |
| protein homodimerization activity | Binding to an identical protein to form a homodimer. |
3 GO annotations of biological process
| Name | Definition |
|---|---|
| aspartyl-tRNA aminoacylation | The process of coupling aspartate to aspartyl-tRNA, catalyzed by aspartyl-tRNA synthetase. The aspartyl-tRNA synthetase is a class-II synthetase. The activated amino acid is transferred to the 3'-OH group of an aspartic acid accetping tRNA. |
| mitochondrial asparaginyl-tRNA aminoacylation | The process of coupling asparagine to asparaginyl-tRNA in a mitochondrion, catalyzed by asparaginyl-tRNA synthetase. In tRNA aminoacylation, the amino acid is first activated by linkage to AMP and then transferred to either the 2'- or the 3'-hydroxyl group of the 3'-adenosine residue of the tRNA. |
| tRNA aminoacylation | The chemical reactions and pathways by which the various amino acids become bonded to their corresponding tRNAs. The most common route for synthesis of aminoacyl tRNA is by the formation of an ester bond between the 3'-hydroxyl group of the most 3' adenosine of the tRNA and the alpha carboxylic acid group of an amino acid, usually catalyzed by the cognate aminoacyl-tRNA ligase. A given aminoacyl-tRNA ligase aminoacylates all species of an isoaccepting group of tRNA molecules. |
3 homologous proteins in AiPD
| 10 | 20 | 30 | 40 | 50 | 60 |
| MYLGFWLSRL | CRGLSRPIGK | TMRPIWGSLS | RNLALSSQRI | PEFSSFVART | NTCGELRSSH |
| 70 | 80 | 90 | 100 | 110 | 120 |
| LGQEVTLCGW | IQYRRQNTFL | VLRDCHGLVQ | ILIPQDESAA | SVRRILCEAP | VESVVRVSGT |
| 130 | 140 | 150 | 160 | 170 | 180 |
| VISRPPGQEN | PKMPTGEIEI | KVKTAELLNA | CKKLPFEIKD | FVKKTEALRL | QYRYLDLRSF |
| 190 | 200 | 210 | 220 | 230 | 240 |
| QMQYNLRLRS | QMVMKMREYL | CNLHGFVDIE | TPTLFKRTPG | GAKEFLVPSR | EPGKFYSLPQ |
| 250 | 260 | 270 | 280 | 290 | 300 |
| SPQQFKQLLM | VGGLDRYFQV | ARCYRDEGSR | PDRQPEFTQI | DIEMSFVEQT | GIQRLVEGLL |
| 310 | 320 | 330 | 340 | 350 | 360 |
| QYSWPGDKDP | LVTPFPSMTF | AEALATYGTD | KPDTRFGMKI | VDVSDVFRNT | ELRFLQDALA |
| 370 | 380 | 390 | 400 | 410 | 420 |
| KPQGTVKAIC | VHDGAKYLRK | EDIEFIRKFA | VHHFSQEVLP | IFLNAKKNWS | SPFAKFIMEE |
| 430 | 440 | 450 | 460 | 470 | 480 |
| ERLELARSME | IQEEDIVLLT | AGEHEKACSL | LGKLRLECAD | LLEMRGAVLR | DPAVFSFLWV |
| 490 | 500 | 510 | 520 | 530 | 540 |
| VDFPLFLAKE | ESPTELESAH | HPFTAPNSSD | IHLLYTEPEK | VRGQHYDLVL | NGNEIGGGSV |
| 550 | 560 | 570 | 580 | 590 | 600 |
| RIHDAQLQRY | ILETLLKEDV | KLLSHLLQAL | DYGAPPHGGI | ALGLDRLVCL | VTGAPSIRDV |
| 610 | 620 | 630 | 640 | 650 | |
| IAFPKSYRGQ | DLMSNAPDSV | SPEELKPYHI | HVLWPADSEE | ESASATPSKH | LSS |