Q12387
Gene name |
MDM20 (DEC1, YOL076W) |
Protein name |
N-terminal acetyltransferase B complex subunit MDM20 |
Names |
NatB complex subunit MDM20, Dislikes extra CIN8 protein 1, Mitochondrial distribution and morphology protein 20 |
Species |
Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) |
KEGG Pathway |
sce:YOL076W |
EC number |
|
Protein Class |
|
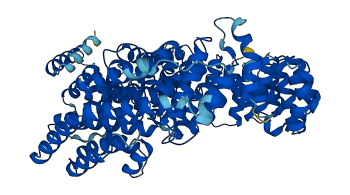
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
3 structures for Q12387
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| 8BIP | EM | 310 A | B | 1-796 | PDB |
| 8BJQ | EM | 380 A | B/D | 1-796 | PDB |
| AF-Q12387-F1 | Predicted | AlphaFoldDB |
18 variants for Q12387
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| s15-187180 | 53 | K>E | No | SGRP | |
| s15-187204 | 61 | E>K | No | SGRP | |
| s15-187401 | 126 | Q>H | No | SGRP | |
| s15-187687 | 222 | A>T | No | SGRP | |
| s15-187949 | 309 | Y>C | No | SGRP | |
| s15-188140 | 373 | I>F | No | SGRP | |
| s15-188149 | 376 | D>N | No | SGRP | |
| s15-188308 | 429 | E>K | No | SGRP | |
| s15-188321 | 433 | A>V | No | SGRP | |
| s15-188662 | 547 | T>S | No | SGRP | |
| s15-188862 | 613 | L>F | No | SGRP | |
| s15-188908 | 629 | E>Q | No | SGRP | |
| s15-188972 | 650 | I>T | No | SGRP | |
| s15-189241 | 740 | S>G | No | SGRP | |
| s15-189256 | 745 | V>I | No | SGRP | |
| s15-189284 | 754 | V>G | No | SGRP | |
| s15-189304 | 761 | K>Q | No | SGRP | |
| s15-189367 | 782 | I>V | No | SGRP |
No associated diseases with Q12387
No regional properties for Q12387
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| No domain, repeats, and functional sites for Q12387 | |||
2 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
| NatB complex | A conserved complex that catalyzes the transfer of an acetyl group to the N-terminal residue of a protein acceptor molecule that has a Met-Glu, Met-Asp, Met-Asn, or Met-Met N-terminus. In Saccharomyces the complex includes Nat3p and Mdm20p. |
No GO annotations of molecular function
| Name | Definition |
|---|---|
| No GO annotations for molecular function |
5 GO annotations of biological process
| Name | Definition |
|---|---|
| cytoskeleton organization | A process that is carried out at the cellular level which results in the assembly, arrangement of constituent parts, or disassembly of cytoskeletal structures. |
| mitochondrion inheritance | The distribution of mitochondria, including the mitochondrial genome, into daughter cells after mitosis or meiosis, mediated by interactions between mitochondria and the cytoskeleton. |
| N-terminal peptidyl-methionine acetylation | The acetylation of the N-terminal methionine of proteins to form the derivative N-acetyl-L-methionine. |
| N-terminal protein amino acid acetylation | The acetylation of the N-terminal amino acid of proteins. |
| regulation of actin cytoskeleton organization | Any process that modulates the frequency, rate or extent of the formation, arrangement of constituent parts, or disassembly of cytoskeletal structures comprising actin filaments and their associated proteins. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSDKIQEEIL | GLVSRSNFKQ | CYAKLGQLQK | QFPNALYFKI | LETYVKFKQS | PGKFDYNKLL |
| 70 | 80 | 90 | 100 | 110 | 120 |
| EEPYGLKGTT | ITGDTRSLEF | LHNFFVELGK | YDEALHVYER | GNFKFPSYEL | SYHWFMKALE |
| 130 | 140 | 150 | 160 | 170 | 180 |
| DSNYNQMSKA | SLQLAKYSDS | GNLPKRAYYF | WNAISILAVS | RFQENTLSDP | KKILLSRLAR |
| 190 | 200 | 210 | 220 | 230 | 240 |
| QSLLDLKPFQ | NVQEIIVYCL | VLDELFPQSR | EISEEIVAIT | FANFDTSVNL | YLKNFILKHT |
| 250 | 260 | 270 | 280 | 290 | 300 |
| KLLNSPQKLF | EVCSKLIEKG | LDDYELITNL | IDAAYKLSKS | KDEVKQWIDE | NLGDSRNTRL |
| 310 | 320 | 330 | 340 | 350 | 360 |
| ARLKLDIMYT | DSVSESSLSY | YLSKYHNKPC | CSIDLNHYSG | HINIDMLKSI | MSKYDPEDKD |
| 370 | 380 | 390 | 400 | 410 | 420 |
| LIHHCNILEL | GLIGSDSINN | YNKFKGTLEK | KSVTDYSSCS | TFLLEIVKDK | CKKTNPELKD |
| 430 | 440 | 450 | 460 | 470 | 480 |
| VLLCITILEN | YQAKDPHNFD | TMCWLIVLYM | YLGLVPDAYF | HFINLKIKNV | QTDSLDYMIF |
| 490 | 500 | 510 | 520 | 530 | 540 |
| SRFSTLFPNK | QSDFYSKTFH | EHNNLYDTSL | ANLPRYIQVA | FERNSYSKIL | GMLEMRDKLM |
| 550 | 560 | 570 | 580 | 590 | 600 |
| KSYTRWTKTL | ENLQFSRLCN | DKRGHLLQKL | HEDWRSLEMT | QSVSFSDNRD | FSILDENFAQ |
| 610 | 620 | 630 | 640 | 650 | 660 |
| FLNRGKILEY | ANLNEESIFL | TLIRELIIEA | LPNGEKTEQI | SALLKKLPSI | NLEELLNNNL |
| 670 | 680 | 690 | 700 | 710 | 720 |
| TEVESASFLI | FFEIYENNGK | NLHDLISRLM | KVPINAKQNW | MVSHTYLTKM | ATLKTLDSLK |
| 730 | 740 | 750 | 760 | 770 | 780 |
| RIKDKEIQKL | IKNSLKELRS | CCDDVFKGYS | KALVQAYEEL | KKDECGNLLK | ELDVKAENVK |
| 790 | |||||
| NIKNSLLGIQ | KSVRNL |