Q9Z9F4
Gene name |
lon |
Protein name |
Lon protease |
Names |
ATP-dependent protease La |
Species |
Chlamydia pneumoniae (Chlamydophila pneumoniae) |
KEGG Pathway |
cpt:CpB0031 |
EC number |
3.4.21.53: Serine endopeptidases |
Protein Class |
|
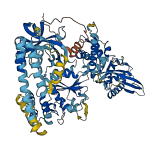
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q9Z9F4
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q9Z9F4-F1 | Predicted | AlphaFoldDB |
No variants for Q9Z9F4
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q9Z9F4 | |||||
No associated diseases with Q9Z9F4
5 regional properties for Q9Z9F4
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Lon protease, N-terminal domain | 42 - 238 | IPR003111 |
| domain | AAA+ ATPase domain | 385 - 530 | IPR003593 |
| domain | ATPase, AAA-type, core | 389 - 525 | IPR003959 |
| active_site | Peptidase S16, active site | 720 - 728 | IPR008268 |
| domain | Peptidase S16, Lon proteolytic domain | 612 - 817 | IPR008269 |
Functions
| Description | ||
|---|---|---|
| EC Number | 3.4.21.53 | Serine endopeptidases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP hydrolysis activity | Catalysis of the reaction: ATP + H2O = ADP + H+ phosphate. ATP hydrolysis is used in some reactions as an energy source, for example to catalyze a reaction or drive transport against a concentration gradient. |
| ATP-dependent peptidase activity | Catalysis of the hydrolysis of peptide bonds, driven by ATP hydrolysis. |
| sequence-specific DNA binding | Binding to DNA of a specific nucleotide composition, e.g. GC-rich DNA binding, or with a specific sequence motif or type of DNA e.g. promotor binding or rDNA binding. |
| serine-type endopeptidase activity | Catalysis of the hydrolysis of internal, alpha-peptide bonds in a polypeptide chain by a catalytic mechanism that involves a catalytic triad consisting of a serine nucleophile that is activated by a proton relay involving an acidic residue (e.g. aspartate or glutamate) and a basic residue (usually histidine). |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| cellular response to heat | Any process that results in a change in state or activity of a cell (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of a heat stimulus, a temperature stimulus above the optimal temperature for that organism. |
| protein quality control for misfolded or incompletely synthesized proteins | The chemical reactions and pathways resulting in the breakdown of misfolded or attenuated proteins. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MDSTTNSDSP | ILDPNPEDVE | KLLDESEEES | EDQSTERLLP | SELFILPLNK | RPFFPGMAAP |
| 70 | 80 | 90 | 100 | 110 | 120 |
| ILIESGPYYE | VLKVLAKSSQ | KYIGLVLTKK | ENADILKVSF | NQLHKTGVAA | RILRIMPIEG |
| 130 | 140 | 150 | 160 | 170 | 180 |
| GSAQVLLSIE | ERIRIIEPIK | DKYLKARVSY | HADNKELTEE | LKAYSISIVS | VIKDLLKLNP |
| 190 | 200 | 210 | 220 | 230 | 240 |
| LFKEELQIFL | GHSDFTEPGK | LADFSVALTT | ATREELQEVL | ETTNMHDRID | KALILLKKEL |
| 250 | 260 | 270 | 280 | 290 | 300 |
| DLSRLQSSIN | QKIEATITKS | QKEFFLKEQL | KTIKKELGLE | KEDRAIDIEK | FSERLRKRHV |
| 310 | 320 | 330 | 340 | 350 | 360 |
| PDYAMEVIQD | EIEKLQTLET | SSAEYTVCRN | YLDWLTIIPW | GIQSKEYHDL | KKAEIVLNKD |
| 370 | 380 | 390 | 400 | 410 | 420 |
| HYGLDEIKQR | ILELISVGKL | SKGLKGSIIC | LVGPPGVGKT | SIGRSIAKVL | HRKFFRFSVG |
| 430 | 440 | 450 | 460 | 470 | 480 |
| GMRDEAEIKG | HRRTYIGAMP | GKMVQALKQS | QAMNPVIMID | EVDKIGASYH | GDPASALLEV |
| 490 | 500 | 510 | 520 | 530 | 540 |
| LDPEQNKDFL | DHYLDVRVDL | SNVLFILTAN | VLDTIPDPLL | DRMEILRLSG | YILEEKLQIA |
| 550 | 560 | 570 | 580 | 590 | 600 |
| KKYLVPKARK | EIGLTASEVN | FQPEALKYMI | NNYAREAGVR | TLNGNIKKVL | RKVALKIVQN |
| 610 | 620 | 630 | 640 | 650 | 660 |
| QEKPKSKKIT | FKISSKNLQT | YLGKPIFSSD | RFYESTPVGV | ATGLAWTSLG | GATLYIESVQ |
| 670 | 680 | 690 | 700 | 710 | 720 |
| VSSLKTDMHL | TGQAGEVMKE | SSQIAWTYLH | SALHRYAPGY | TFFPKSQVHI | HIPEGATPKD |
| 730 | 740 | 750 | 760 | 770 | 780 |
| GPSAGITMVT | SLLSLLLETP | VVNNLGMTGE | ITLTGRVLGV | GGIREKLIAA | RRSRLNILIF |
| 790 | 800 | 810 | |||
| PEDNRRDYEE | LPAYLKTGLK | IHFVSHYDDV | LKVAFPKLK |