Q9CTG6
Gene name |
Atp13a2 |
Protein name |
Polyamine-transporting ATPase 13A2 |
Names |
|
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:74772 |
EC number |
|
Protein Class |
|
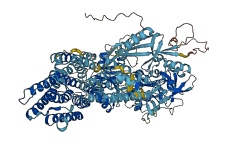
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q9CTG6
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q9CTG6-F1 | Predicted | AlphaFoldDB |
87 variants for Q9CTG6
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs3388712418 | 28 | L>P | No | EVA | |
| rs3388733779 | 32 | A>D | No | EVA | |
| rs217116759 | 104 | T>K | No | EVA | |
| rs13461262 | 112 | V>L | No | EVA | |
| rs3388724996 | 113 | V>F | No | EVA | |
| rs3388732305 | 129 | R>P | No | EVA | |
| rs3388718544 | 164 | Q>K | No | EVA | |
| rs28260916 | 186 | G>S | No | EVA | |
| rs3388727875 | 190 | D>V | No | EVA | |
| rs263930313 | 192 | V>I | No | EVA | |
| rs3388733743 | 204 | Q>H | No | EVA | |
| rs252421673 | 228 | A>V | No | EVA | |
| rs3388727447 | 241 | F>Y | No | EVA | |
| rs3388723912 | 250 | H>L | No | EVA | |
| rs3388727454 | 261 | I>F | No | EVA | |
| rs3388728530 | 275 | K>E | No | EVA | |
| rs1132291919 | 277 | S>N | No | EVA | |
| rs28260906 | 280 | L>M | No | EVA | |
| rs3394909624 | 289 | R>V | No | EVA | |
| rs3388723979 | 303 | D>E | No | EVA | |
| rs3411548080 | 326 | A>E | No | EVA | |
| rs3388725017 | 333 | C>Y | No | EVA | |
| rs3388721360 | 347 | V>M | No | EVA | |
| rs3388728778 | 379 | R>* | No | EVA | |
| rs226884563 | 392 | R>Q | No | EVA | |
| rs3395142262 | 404 | S>V | No | EVA | |
| rs3388732287 | 420 | S>T | No | EVA | |
| rs28260889 | 429 | V>I | No | EVA | |
| rs28260888 | 440 | I>V | No | EVA | |
| rs3388724927 | 445 | N>K | No | EVA | |
| rs3388733777 | 474 | V>L | No | EVA | |
| rs28260885 | 485 | T>A | No | EVA | |
| rs225795681 | 530 | V>M | No | EVA | |
| rs3395030541 | 535 | V>G | No | EVA | |
| rs3395030552 | 537 | E>V | No | EVA | |
| rs235529277 | 539 | C>R | No | EVA | |
| rs3394842561 | 543 | L>* | No | EVA | |
| rs3395004309 | 561 | D>E | No | EVA | |
| rs3395030542 | 562 | T>A | No | EVA | |
| rs3388723876 | 562 | T>N | No | EVA | |
| rs3395142244 | 574 | E>V | No | EVA | |
| rs3388728771 | 602 | P>S | No | EVA | |
| rs3388723944 | 625 | S>P | No | EVA | |
| rs3388733747 | 631 | D>G | No | EVA | |
| rs3388733723 | 638 | G>W | No | EVA | |
| rs3388721410 | 646 | V>I | No | EVA | |
| rs3388732331 | 657 | C>* | No | EVA | |
| rs3388712497 | 671 | Q>L | No | EVA | |
| rs28260875 | 695 | A>E | No | EVA | |
| rs3388732288 | 703 | D>G | No | EVA | |
| rs3388721751 | 706 | E>V | No | EVA | |
| rs3388728537 | 716 | V>I | No | EVA | |
| rs3388721414 | 753 | V>L | No | EVA | |
| rs3388732252 | 775 | E>* | No | EVA | |
| rs3388702909 | 793 | M>I | No | EVA | |
| rs3388718558 | 795 | G>W | No | EVA | |
| rs261474003 | 803 | T>M | No | EVA | |
| rs229130053 | 805 | P>L | No | EVA | |
| rs259691467 | 809 | S>F | No | EVA | |
| rs3388721417 | 816 | G>A | No | EVA | |
| rs3388732314 | 836 | Q>K | No | EVA | |
| rs3388724023 | 839 | V>I | No | EVA | |
| rs3388727424 | 840 | F>L | No | EVA | |
| rs3388733720 | 842 | R>* | No | EVA | |
| rs3388728448 | 845 | P>L | No | EVA | |
| rs3388727499 | 866 | G>R | No | EVA | |
| rs3388714494 | 873 | G>W | No | EVA | |
| rs3388721777 | 892 | V>L | No | EVA | |
| rs3388727491 | 908 | V>I | No | EVA | |
| rs3388723937 | 932 | T>N | No | EVA | |
| rs3388728529 | 938 | L>P | No | EVA | |
| rs3394842531 | 941 | Y>* | No | EVA | |
| rs3388733706 | 945 | T>I | No | EVA | |
| rs3388732285 | 980 | R>L | No | EVA | |
| rs3388712489 | 999 | A>V | No | EVA | |
| rs3388712469 | 1030 | N>H | No | EVA | |
| rs3388712463 | 1043 | S>F | No | EVA | |
| rs3388712463 | 1043 | S>Y | No | EVA | |
| rs3388724932 | 1080 | V>I | No | EVA | |
| rs3388732315 | 1109 | L>P | No | EVA | |
| rs28260845 | 1111 | G>S | No | EVA | |
| rs3388723949 | 1146 | K>N | No | EVA | |
| rs3388702832 | 1150 | R>Q | No | EVA | |
| rs3388727859 | 1156 | A>V | No | EVA | |
| rs3388723905 | 1158 | H>D | No | EVA | |
| rs3388723988 | 1160 | W>C | No | EVA | |
| rs3388724978 | 1163 | L>M | No | EVA |
No associated diseases with Q9CTG6
Functions
15 GO annotations of cellular component
| Name | Definition |
|---|---|
| autophagosome | A double-membrane-bounded compartment that engulfs endogenous cellular material as well as invading microorganisms to target them to the lytic vacuole/lysosome for degradation as part of macroautophagy. |
| autophagosome membrane | The lipid bilayer surrounding an autophagosome, a double-membrane-bounded vesicle in which endogenous cellular material is sequestered. |
| integral component of lysosomal membrane | The component of the lysosome membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
| late endosome | A prelysosomal endocytic organelle differentiated from early endosomes by lower lumenal pH and different protein composition. Late endosomes are more spherical than early endosomes and are mostly juxtanuclear, being concentrated near the microtubule organizing center. |
| late endosome membrane | The lipid bilayer surrounding a late endosome. |
| lysosomal membrane | The lipid bilayer surrounding the lysosome and separating its contents from the cell cytoplasm. |
| lysosome | A small lytic vacuole that has cell cycle-independent morphology found in most animal cells and that contains a variety of hydrolases, most of which have their maximal activities in the pH range 5-6. The contained enzymes display latency if properly isolated. About 40 different lysosomal hydrolases are known and lysosomes have a great variety of morphologies and functions. |
| membrane | A lipid bilayer along with all the proteins and protein complexes embedded in it an attached to it. |
| multivesicular body | A type of endosome in which regions of the limiting endosomal membrane invaginate to form internal vesicles; membrane proteins that enter the internal vesicles are sequestered from the cytoplasm. |
| multivesicular body membrane | The lipid bilayer surrounding a multivesicular body. |
| neuron projection | A prolongation or process extending from a nerve cell, e.g. an axon or dendrite. |
| neuronal cell body | The portion of a neuron that includes the nucleus, but excludes cell projections such as axons and dendrites. |
| transport vesicle | Any of the vesicles of the constitutive secretory pathway, which carry cargo from the endoplasmic reticulum to the Golgi, between Golgi cisternae, from the Golgi to the ER (retrograde transport) or to destinations within or outside the cell. |
| vesicle | Any small, fluid-filled, spherical organelle enclosed by membrane. |
| vesicle membrane | The lipid bilayer surrounding any membrane-bounded vesicle in the cell. |
8 GO annotations of molecular function
| Name | Definition |
|---|---|
| ABC-type polyamine transporter activity | Catalysis of the reaction: ATP + H2O + polyamine(out) = ADP + phosphate + polyamine(in). |
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP hydrolysis activity | Catalysis of the reaction: ATP + H2O = ADP + H+ phosphate. ATP hydrolysis is used in some reactions as an energy source, for example to catalyze a reaction or drive transport against a concentration gradient. |
| ATPase-coupled cation transmembrane transporter activity | Enables the transfer of a solute or solutes from one side of a membrane to the other according to the reaction: ATP + H2O + cation(out) = ADP + phosphate + cation(in). |
| metal ion binding | Binding to a metal ion. |
| P-type transmembrane transporter activity | Primary active transporter that auto-phosphorylates (hence P) at a key conserved aspartate residue, generating a conformational change that allows transport of the substrate. Hydrolysis of the phosphorylated Asp residue, catalyzed by the actuator (A) domain, results in another state with occluded substrates. Upon dissociation of Mg2+ and inorganic phosphate (Pi), the enzyme reverts to the initial state, in which the counter-transported substrate is released into the cytosol. |
| phosphatidic acid binding | Binding to phosphatidic acid, any of a class of glycerol phosphate in which both the remaining hydroxyl groups of the glycerol moiety are esterified with fatty acids. |
| phosphatidylinositol-3,5-bisphosphate binding | Binding to phosphatidylinositol-3,5-bisphosphate, a derivative of phosphatidylinositol in which the inositol ring is phosphorylated at the 3' and 5' positions. |
29 GO annotations of biological process
| Name | Definition |
|---|---|
| autophagosome organization | A process that is carried out at the cellular level which results in the assembly, arrangement of constituent parts, or disassembly of an autophagosome. |
| autophagosome-lysosome fusion | The process in which autophagosomes, double-membraned vesicles containing cytoplasmic material, fuse with a vacuole (yeast) or lysosome (e.g. mammals and insects). In the case of yeast, inner membrane-bounded structures (autophagic bodies) appear in the vacuole. Fusion provides an acidic environment and digestive function to the interior of the autophagosome. |
| autophagy | The cellular catabolic process in which cells digest parts of their own cytoplasm; allows for both recycling of macromolecular constituents under conditions of cellular stress and remodeling the intracellular structure for cell differentiation. |
| cellular calcium ion homeostasis | Any process involved in the maintenance of an internal steady state of calcium ions at the level of a cell. |
| cellular iron ion homeostasis | Any process involved in the maintenance of an internal steady state of iron ions at the level of a cell. |
| cellular response to manganese ion | Any process that results in a change in state or activity of a cell (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of a manganese ion stimulus. |
| cellular response to oxidative stress | Any process that results in a change in state or activity of a cell (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of oxidative stress, a state often resulting from exposure to high levels of reactive oxygen species, e.g. superoxide anions, hydrogen peroxide (H2O2), and hydroxyl radicals. |
| cellular zinc ion homeostasis | Any process involved in the maintenance of an internal steady state of zinc ions at the level of a cell. |
| extracellular exosome biogenesis | The assembly and secretion of an extracellular exosome, a membrane-bounded vesicle that is released into the extracellular region by fusion of the limiting endosomal membrane of a multivesicular body with the plasma membrane. |
| lipid homeostasis | Any process involved in the maintenance of an internal steady state of lipid within an organism or cell. |
| lysosomal transport | The directed movement of substances into, out of or within a lysosome. |
| peptidyl-aspartic acid autophosphorylation | The phosphorylation by a protein of one or more of its own aspartate amino acid residues, or an aspartate residue on an identical protein. |
| polyamine transmembrane transport | The process in which a polyamine macromolecule is transported across a membrane. |
| positive regulation of exosomal secretion | Any process that activates or increases the frequency, rate or extent of exosomal secretion. |
| positive regulation of gene expression | Any process that increases the frequency, rate or extent of gene expression. Gene expression is the process in which a gene's coding sequence is converted into a mature gene product (protein or RNA). |
| positive regulation of protein secretion | Any process that activates or increases the frequency, rate or extent of the controlled release of a protein from a cell. |
| protein localization to lysosome | A process in which a protein is transported to, or maintained in, a location within a lysosome. |
| regulation of autophagosome size | Any process that modulates the size of the autophagosome. |
| regulation of endopeptidase activity | Any process that modulates the frequency, rate or extent of endopeptidase activity, the endohydrolysis of peptide bonds within proteins. |
| regulation of glucosylceramidase activity | Any process that modulates the frequency, rate or extent of glucosylceramidase activity. |
| regulation of intracellular protein transport | Any process that modulates the frequency, rate or extent of the directed movement of proteins within cells. |
| regulation of lysosomal protein catabolic process | Any process that modulates the frequency, rate or extent of lysosomal protein catabolic process. |
| regulation of macroautophagy | Any process that modulates the frequency, rate or extent of macroautophagy. |
| regulation of mitochondrion organization | Any process that modulates the frequency, rate or extent of a process involved in the formation, arrangement of constituent parts, or disassembly of a mitochondrion. |
| regulation of protein localization to nucleus | Any process that modulates the frequency, rate or extent of protein localization to nucleus. |
| regulation of ubiquitin-specific protease activity | Any process that modulates the frequency, rate or extent of regulation of ubiquitin-specific protease activity (deubiquitinase) activity. |
| spermine transmembrane transport | The process in which spermine is transported across a membrane. |
| transmembrane transport | The process in which a solute is transported across a lipid bilayer, from one side of a membrane to the other. |
| zinc ion homeostasis | Any process involved in the maintenance of an internal steady state of zinc ions within an organism or cell. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSADSSLLMG | STPPSYGTLT | TGTSIDPLSS | SASSVRLSGY | CGSPWRAIGY | HAAVWMLAGI |
| 70 | 80 | 90 | 100 | 110 | 120 |
| PWLLFRWKPL | WGVRLRLKPC | SLAHAETLVI | EIKDKEGSSR | QLFTVQVQTE | AVVQGSLELP |
| 130 | 140 | 150 | 160 | 170 | 180 |
| PQAQAEDGRS | QAAVGVTPEG | TWQDTSELHR | QEEAKQVLRY | YVLQGQRYVW | METQQAFCQV |
| 190 | 200 | 210 | 220 | 230 | 240 |
| SLLDHGRTCD | DVHCSSSGLS | LQDQATRKTI | YGPNVISIPV | KSYLQLLADE | ALNPYYGFQA |
| 250 | 260 | 270 | 280 | 290 | 300 |
| FSIALWLADH | YYWYALCIFL | ISAISICLAL | YKTRKQSLTL | RDMVKLSVRV | QVCRPGGEEE |
| 310 | 320 | 330 | 340 | 350 | 360 |
| WVDSSELVPG | DCLVLPQEGG | VMPCDAALVA | GECVVNESSL | TGESTPVLKT | ALPEGPKPYC |
| 370 | 380 | 390 | 400 | 410 | 420 |
| PETHRRHTLF | CGTLILQARA | YVGPRVLAVV | TRTGFCTAKG | GLVSSILHPR | PISFKFYKHS |
| 430 | 440 | 450 | 460 | 470 | 480 |
| MKFVAALSVL | ALLGTVYSII | ILYRNRVPVR | EIVIRALDLV | TVVVPPALPA | AMTVCTLYAQ |
| 490 | 500 | 510 | 520 | 530 | 540 |
| SRLRTQGIFC | IHPLRINLGG | KLRLVCFDKT | GTLTEDGLDV | MGVVPLKGQV | LLPLVPEPCH |
| 550 | 560 | 570 | 580 | 590 | 600 |
| LPLGPLLRAL | ATCHALSQLH | DTPVGDPMDL | KMVESTGWVL | EEGPAAGSAP | GSQVLVVMRP |
| 610 | 620 | 630 | 640 | 650 | 660 |
| PPGGPRQQEE | PPVPVSVLCR | FPFSSALQRM | DVVVTWPGAT | QPEAYVKGSP | ELVASLCSPE |
| 670 | 680 | 690 | 700 | 710 | 720 |
| TVPSDFSQVL | QSYTAAGYRV | VALAGKPLPI | APSLAAAQQL | TRDTVERELS | LLGLLVMRNL |
| 730 | 740 | 750 | 760 | 770 | 780 |
| LKPQTAPVIQ | TLRKTGIRTV | MVTGDNLQTA | VTVARACGMV | GAQEHLAVIH | ATHPEQGQPA |
| 790 | 800 | 810 | 820 | 830 | 840 |
| ALEFLPTESS | AVMNGAKATG | YPTVPEPQSC | HLALSGSTFA | VLRKHFPKLL | PKVLVQATVF |
| 850 | 860 | 870 | 880 | 890 | 900 |
| ARMAPEQKTE | LVCELQRLQY | CVGMCGDGAN | DCGALKAADV | GISLSQAEAS | VVSPFTSSMA |
| 910 | 920 | 930 | 940 | 950 | 960 |
| SIECVPTVIR | EGRCSLDTSF | SVFKYMALYS | LTQFISVLIL | YTINTNLGDL | QFLAIDLVIT |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| TTVAVLMSRT | GPALTLVRAR | PPGALLSVPV | LGSLLLQVAL | VAGIQLGGYF | LVIAQPWFVP |
| 1030 | 1040 | 1050 | 1060 | 1070 | 1080 |
| LNRTVPAPDN | LPNYENTVVF | SLSGFQYLIL | AAAVSKGAPF | RQPLYTNVPF | LVALALLGSV |
| 1090 | 1100 | 1110 | 1120 | 1130 | 1140 |
| LVGLILVPGL | LQGPLGLRNI | VDSSFKLLLL | GLVAFNFVGA | FMLESVLDQC | LPACLRWLRP |
| 1150 | 1160 | ||||
| KRASKKQFKR | LQQELAEHPW | PTLPVGSVR |