Q92462
Gene name |
pub1 (SPAC11G7.02) |
Protein name |
E3 ubiquitin-protein ligase pub1 |
Names |
HECT-type E3 ubiquitin transferase pub1 |
Species |
Schizosaccharomyces pombe (strain 972 / ATCC 24843) (Fission yeast) |
KEGG Pathway |
spo:SPAC11G7.02 |
EC number |
2.3.2.26: Aminoacyltransferases |
Protein Class |
|
Descriptions
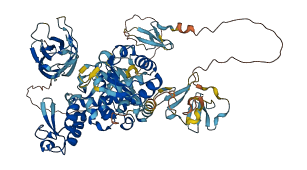
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q92462
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q92462-F1 | Predicted | AlphaFoldDB |
1 variants for Q92462
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| I_3964465_C_T | 300 | P>L | No | Jeffares_SNPs |
No associated diseases with Q92462
5 regional properties for Q92462
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | C2 domain | 1 - 111 | IPR000008 |
| domain | HECT domain | 413 - 767 | IPR000569 |
| domain | WW domain | 205 - 238 | IPR001202-1 |
| domain | WW domain | 288 - 321 | IPR001202-2 |
| domain | WW domain | 345 - 378 | IPR001202-3 |
Functions
| Description | ||
|---|---|---|
| EC Number | 2.3.2.26 | Aminoacyltransferases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
4 GO annotations of cellular component
| Name | Definition |
|---|---|
| cell periphery | The part of a cell encompassing the cell cortex, the plasma membrane, and any external encapsulating structures. |
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
| Golgi apparatus | A membrane-bound cytoplasmic organelle of the endomembrane system that further processes the core oligosaccharides (e.g. N-glycans) added to proteins in the endoplasmic reticulum and packages them into membrane-bound vesicles. The Golgi apparatus operates at the intersection of the secretory, lysosomal, and endocytic pathways. |
| membrane | A lipid bilayer along with all the proteins and protein complexes embedded in it an attached to it. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| phospholipid binding | Binding to a phospholipid, a class of lipids containing phosphoric acid as a mono- or diester. |
| ubiquitin protein ligase activity | Catalysis of the transfer of ubiquitin to a substrate protein via the reaction X-ubiquitin + S -> X + S-ubiquitin, where X is either an E2 or E3 enzyme, the X-ubiquitin linkage is a thioester bond, and the S-ubiquitin linkage is an amide bond: an isopeptide bond between the C-terminal glycine of ubiquitin and the epsilon-amino group of lysine residues in the substrate or, in the linear extension of ubiquitin chains, a peptide bond the between the C-terminal glycine and N-terminal methionine of ubiquitin residues. |
10 GO annotations of biological process
| Name | Definition |
|---|---|
| cytoplasm to vacuole transport by the NVT pathway | A pathway targeting soluble cytosolic proteins to the vacuole lumen. It uses a selective autophagy receptor protein Nbr1, which is an ortholog of mammalian NBR1, and is remotely related to S. cerevisiae Cvt pathway receptor protein Atg19. Similar to the Cvt pathway, the cargos transported by this pathway are hydrolases, which presumably contribute to the hydrolytic activities in the vacuole lumen. Different from the Cvt pathway, this pathway does not require the macroautophagy machinery, but instead relies on the ESCRT machinery for cargo sequestration. This pathway is observed in the fission yeast S. pombe. |
| negative regulation of leucine import across plasma membrane | Any process that stops, prevents or reduces the frequency, rate or extent of leucine import across plasma membrane. |
| negative regulation of uracil import across plasma membrane | Any process that stops, prevents or reduces the frequency, rate or extent of uracil import across plasma membrane. |
| proteasome-mediated ubiquitin-dependent protein catabolic process | The chemical reactions and pathways resulting in the breakdown of a protein or peptide by hydrolysis of its peptide bonds, initiated by the covalent attachment of ubiquitin, and mediated by the proteasome. |
| protein localization to Golgi apparatus | A process in which a protein is transported to, or maintained in, a location within the Golgi apparatus. |
| protein modification by small protein conjugation or removal | A protein modification process in which one or more groups of a small protein, such as ubiquitin or a ubiquitin-like protein, are covalently attached to or removed from a target protein. |
| protein polyubiquitination | Addition of multiple ubiquitin groups to a protein, forming a ubiquitin chain. |
| protein ubiquitination | The process in which one or more ubiquitin groups are added to a protein. |
| regulation of intracellular pH | Any process that modulates the internal pH of a cell, measured by the concentration of the hydrogen ion. |
| ubiquitin-dependent protein catabolic process | The chemical reactions and pathways resulting in the breakdown of a protein or peptide by hydrolysis of its peptide bonds, initiated by the covalent attachment of a ubiquitin group, or multiple ubiquitin groups, to the protein. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSNSAQSRRI | RVTIVAADGL | YKRDVFRFPD | PFAVLTVDGE | QTHTTTAIKK | TLNPYWNETF |
| 70 | 80 | 90 | 100 | 110 | 120 |
| EVNVTDNSTI | AIQVFDQKKF | KKKGQGFLGV | INLRVGDVLD | LAIGGDEMLT | RDLKKSNENT |
| 130 | 140 | 150 | 160 | 170 | 180 |
| VVHGKIIINL | STTAQSTLQV | PSSAASGART | QRTSITNDPQ | SSQSSSVSRN | PASSRAGSPT |
| 190 | 200 | 210 | 220 | 230 | 240 |
| RDNAPAASPA | SSEPRTFSSF | EDQYGRLPPG | WERRTDNLGR | TYYVDHNTRS | TTWIRPNLSS |
| 250 | 260 | 270 | 280 | 290 | 300 |
| VAGAAAAELH | SSASSANVTE | GVQPSSSNAA | RRTEASVLTS | NATTAGSGEL | PPGWEQRYTP |
| 310 | 320 | 330 | 340 | 350 | 360 |
| EGRPYFVDHN | TRTTTWVDPR | RQQYIRSYGG | PNNATIQQQP | VSQLGPLPSG | WEMRLTNTAR |
| 370 | 380 | 390 | 400 | 410 | 420 |
| VYFVDHNTKT | TTWDDPRLPS | SLDQNVPQYK | RDFRRKLIYF | LSQPALHPLP | GQCHIKVRRN |
| 430 | 440 | 450 | 460 | 470 | 480 |
| HIFEDSYAEI | MRQSATDLKK | RLMIKFDGED | GLDYGGLSRE | YFFLLSHEMF | NPFYCLFEYS |
| 490 | 500 | 510 | 520 | 530 | 540 |
| SVDNYTLQIN | PHSGINPEHL | NYFKFIGRVI | GLAIFHRRFV | DAFFVVSFYK | MILQKKVTLQ |
| 550 | 560 | 570 | 580 | 590 | 600 |
| DMESMDAEYY | RSLVWILDND | ITGVLDLTFS | VEDNCFGEVV | TIDLKPNGRN | IEVTEENKRE |
| 610 | 620 | 630 | 640 | 650 | 660 |
| YVDLVTVWRI | QKRIEEQFNA | FHEGFSELIP | QELINVFDER | ELELLIGGIS | EIDMEDWKKH |
| 670 | 680 | 690 | 700 | 710 | 720 |
| TDYRSYSEND | QIIKWFWELM | DEWSNEKKSR | LLQFTTGTSR | IPVNGFKDLQ | GSDGPRKFTI |
| 730 | 740 | 750 | 760 | ||
| EKAGEPNKLP | KAHTCFNRLD | LPPYTSKKDL | DHKLSIAVEE | TIGFGQE |