Q8VY89
Gene name |
APC7 (At2g39090, T7F6.26) |
Protein name |
Anaphase-promoting complex subunit 7 |
Names |
Cyclosome subunit 7 |
Species |
Arabidopsis thaliana (Mouse-ear cress) |
KEGG Pathway |
ath:AT2G39090 |
EC number |
|
Protein Class |
|
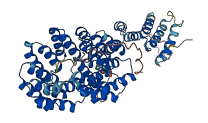
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q8VY89
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q8VY89-F1 | Predicted | AlphaFoldDB |
16 variants for Q8VY89
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| tmp_2_16317030_T_C | 32 | T>A | No | 1000Genomes | |
| ENSVATH01966774 | 34 | S>N | No | 1000Genomes | |
| ENSVATH05681945 | 49 | L>M | No | 1000Genomes | |
| tmp_2_16316553_T_A | 68 | Q>L | No | 1000Genomes | |
| ENSVATH05681927 | 98 | A>T | No | 1000Genomes | |
| tmp_2_16316455_T_C | 101 | I>V | No | 1000Genomes | |
| tmp_2_16315774_C_T | 149 | R>Q | No | 1000Genomes | |
| tmp_2_16315371_T_G | 197 | N>T | No | 1000Genomes | |
| tmp_2_16314493_C_T | 268 | R>K | No | 1000Genomes | |
| ENSVATH14597585 | 296 | Y>F | No | 1000Genomes | |
| tmp_2_16314242_C_T | 326 | R>K | No | 1000Genomes | |
| ENSVATH05681888 | 343 | D>H | No | 1000Genomes | |
| tmp_2_16313976_C_A | 362 | R>L | No | 1000Genomes | |
| ENSVATH13579441 | 416 | A>S | No | 1000Genomes | |
| ENSVATH14597579 | 463 | G>R | No | 1000Genomes | |
| tmp_2_16313176_C_A | 486 | V>F | No | 1000Genomes |
No associated diseases with Q8VY89
2 GO annotations of cellular component
| Name | Definition |
|---|---|
| anaphase-promoting complex | A ubiquitin ligase complex that degrades mitotic cyclins and anaphase inhibitory protein, thereby triggering sister chromatid separation and exit from mitosis. Substrate recognition by APC occurs through degradation signals, the most common of which is termed the Dbox degradation motif, originally discovered in cyclin B. |
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
No GO annotations of molecular function
| Name | Definition |
|---|---|
| No GO annotations for molecular function |
5 GO annotations of biological process
| Name | Definition |
|---|---|
| anaphase-promoting complex-dependent catabolic process | The chemical reactions and pathways resulting in the breakdown of a protein or peptide by hydrolysis of its peptide bonds, initiated by the covalent attachment of ubiquitin, with ubiquitin-protein ligation catalyzed by the anaphase-promoting complex, and mediated by the proteasome. |
| cell division | The process resulting in division and partitioning of components of a cell to form more cells; may or may not be accompanied by the physical separation of a cell into distinct, individually membrane-bounded daughter cells. |
| metaphase/anaphase transition of mitotic cell cycle | The cell cycle process in which a cell progresses from metaphase to anaphase during mitosis, triggered by the activation of the anaphase promoting complex by Cdc20/Sleepy homolog which results in the degradation of Securin. |
| positive regulation of mitotic metaphase/anaphase transition | Any process that activates or increases the frequency, rate or extent of the cell cycle process in which a cell progresses from metaphase to anaphase during mitosis, triggered by the activation of the anaphase promoting complex by Cdc20/Sleepy homolog which results in the degradation of Securin. |
| protein ubiquitination | The process in which one or more ubiquitin groups are added to a protein. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MEVPKEQIAT | LIEHGLYDSA | EMLGCFLVSS | PTVSAETSPQ | LKAENLILLG | DALFHQREHR |
| 70 | 80 | 90 | 100 | 110 | 120 |
| RAIHTYKQAL | HHYTRIPKQS | SGISRSSLSL | STRSSVNASS | ISAINENEVR | FKIASSHFAL |
| 130 | 140 | 150 | 160 | 170 | 180 |
| NETKAAIAEM | ESVKTRSLEM | NILMAKLHRN | SGYNRGAIAF | YKECLRQCPY | VLEAVIGLAE |
| 190 | 200 | 210 | 220 | 230 | 240 |
| LGVSAKDIIS | SFTQTSNRSA | KVSLDQIDPT | RWLQRYVEAQ | CCVASHAYKG | ALELFAELLQ |
| 250 | 260 | 270 | 280 | 290 | 300 |
| RFPNNVHLLT | ETAKVEAIIG | KNDEAIMRFE | KVRSIDPYTL | TSMDEYAMLL | QIKCDYSRLN |
| 310 | 320 | 330 | 340 | 350 | 360 |
| KLVHDLLSVD | HTRAEVFVAL | SVLWERKDAR | TALSYAEKSI | RVDERHIPGY | IMKGNLLLQA |
| 370 | 380 | 390 | 400 | 410 | 420 |
| KRPEAAAIAF | RAAQNLRSDL | RSYQGLVHSY | LAFGKTKEAL | YTAREAMNAM | PQSAKALKLV |
| 430 | 440 | 450 | 460 | 470 | 480 |
| GDVHAFTSSG | REKAKKFYES | GLRLEPGYLG | AVLALAELHL | MEGRNGDAVS | LLERYLKDYA |
| 490 | 500 | 510 | 520 | 530 | 540 |
| DDSLHVKLAQ | VFAATNMLQD | SLSHFQAALR | INPQNEAAKK | GLDRLEKQMK | GIDPDATDEN |
| 550 | |||||
| DENDVEDVDG | DTEEAELM |