Q8VD65
Gene name |
Pik3r4 (Vps15) |
Protein name |
Phosphoinositide 3-kinase regulatory subunit 4 |
Names |
PI3-kinase regulatory subunit 4 |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:75669 |
EC number |
2.7.11.1: Protein-serine/threonine kinases |
Protein Class |
|
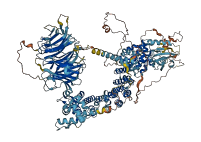
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
165-195 (Activation loop from InterPro)
Target domain |
26-324 (Protein kinase domain) |
Relief mechanism |
|
Assay |
|
Autoinhibited structure

Activated structure
1 structures for Q8VD65
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q8VD65-F1 | Predicted | AlphaFoldDB |
85 variants for Q8VD65
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs3389077079 | 94 | A>T | No | EVA | |
| rs3400600967 | 159 | W>C | No | EVA | |
| rs3400529555 | 159 | W>S | No | EVA | |
| rs3400670817 | 162 | V>D | No | EVA | |
| rs3389063471 | 169 | S>G | No | EVA | |
| rs3389047320 | 247 | V>M | No | EVA | |
| rs3389055772 | 255 | G>V | No | EVA | |
| rs3400627662 | 275 | E>A | No | EVA | |
| rs3389035754 | 354 | I>N | No | EVA | |
| rs33653996 | 360 | H>Q | No | EVA | |
| rs3389047313 | 366 | A>T | No | EVA | |
| rs3389055806 | 374 | G>D | No | EVA | |
| rs3400616986 | 390 | K>Q | No | EVA | |
| rs3400085391 | 393 | D>V | No | EVA | |
| rs3400763674 | 394 | S>C | No | EVA | |
| rs3389055811 | 434 | R>W | No | EVA | |
| rs3389076491 | 441 | L>F | No | EVA | |
| rs3389055801 | 465 | P>L | No | EVA | |
| rs3389055826 | 469 | H>L | No | EVA | |
| rs3389071997 | 479 | R>I | No | EVA | |
| rs3389068036 | 480 | L>Q | No | EVA | |
| rs3389047348 | 485 | N>T | No | EVA | |
| rs3389035760 | 488 | L>M | No | EVA | |
| rs3389035669 | 490 | A>S | No | EVA | |
| rs3389076544 | 498 | E>D | No | EVA | |
| rs47920389 | 513 | N>S | No | EVA | |
| rs3400296083 | 522 | P>H | No | EVA | |
| rs3389068092 | 526 | Y>* | No | EVA | |
| rs3400085373 | 547 | D>N | No | EVA | |
| rs3389066290 | 564 | L>M | No | EVA | |
| rs3389077123 | 581 | M>I | No | EVA | |
| rs3389070345 | 584 | F>L | No | EVA | |
| rs3389068105 | 584 | F>Y | No | EVA | |
| rs3389061446 | 642 | M>I | No | EVA | |
| rs3400616993 | 663 | F>Y | No | EVA | |
| rs3400716706 | 665 | C>Y | No | EVA | |
| rs3389063408 | 683 | A>S | No | EVA | |
| rs3389068063 | 688 | T>I | No | EVA | |
| rs1132143211 | 696 | M>I | No | EVA | |
| rs3389013521 | 700 | D>G | No | EVA | |
| rs1134889429 | 703 | I>N | No | EVA | |
| rs3400602581 | 705 | Q>L | No | EVA | |
| rs3389070420 | 706 | P>A | No | EVA | |
| rs3389070420 | 706 | P>S | No | EVA | |
| rs3400621026 | 708 | I>* | No | EVA | |
| rs3389068222 | 712 | R>G | No | EVA | |
| rs3389043218 | 720 | L>I | No | EVA | |
| rs3389055810 | 728 | I>T | No | EVA | |
| rs3389063411 | 729 | F>L | No | EVA | |
| rs3389068235 | 730 | D>H | No | EVA | |
| rs3389061426 | 747 | M>I | No | EVA | |
| rs3400671827 | 767 | I>M* | No | EVA | |
| rs3400530229 | 772 | K>Q | No | EVA | |
| rs49440445 | 774 | L>M | No | EVA | |
| rs3400085378 | 775 | L>R | No | EVA | |
| rs3389035753 | 820 | D>G | No | EVA | |
| rs3389077050 | 821 | L>M | No | EVA | |
| rs3389055854 | 828 | G>E | No | EVA | |
| rs3389076452 | 829 | R>K | No | EVA | |
| rs3389076477 | 831 | V>G | No | EVA | |
| rs3400621018 | 865 | S>T | No | EVA | |
| rs3400671810 | 868 | P>S | No | EVA | |
| rs1134979949 | 872 | P>T | No | EVA | |
| rs3389061415 | 883 | V>I | No | EVA | |
| rs3389069129 | 895 | S>Y | No | EVA | |
| rs255105531 | 916 | S>N | No | EVA | |
| rs3389063419 | 929 | L>Q | No | EVA | |
| rs3389047317 | 975 | P>L | No | EVA | |
| rs3389068285 | 1001 | V>L | No | EVA | |
| rs3389061420 | 1014 | D>N | No | EVA | |
| rs3389035737 | 1027 | G>W | No | EVA | |
| rs3389070352 | 1073 | A>T | No | EVA | |
| rs3389063404 | 1112 | L>I | No | EVA | |
| rs3389068269 | 1150 | D>G | No | EVA | |
| rs3389076514 | 1154 | C>S | No | EVA | |
| rs3389055861 | 1157 | C>Y | No | EVA | |
| rs3389077067 | 1166 | A>E | No | EVA | |
| rs3389043250 | 1171 | R>S | No | EVA | |
| rs3389068113 | 1178 | S>T | No | EVA | |
| rs3389066211 | 1185 | A>S | No | EVA | |
| rs3389063455 | 1201 | I>F | No | EVA | |
| rs3400297185 | 1218 | G>C | No | EVA | |
| rs3389076531 | 1229 | A>S | No | EVA | |
| rs3389068307 | 1249 | P>H | No | EVA | |
| rs3400530252 | 1270 | L>* | No | EVA |
No associated diseases with Q8VD65
9 regional properties for Q8VD65
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Protein kinase domain | 26 - 324 | IPR000719 |
| repeat | WD40 repeat | 982 - 1030 | IPR001680-1 |
| repeat | WD40 repeat | 1031 - 1070 | IPR001680-2 |
| repeat | WD40 repeat | 1132 - 1169 | IPR001680-3 |
| repeat | WD40 repeat | 1171 - 1214 | IPR001680-4 |
| repeat | WD40 repeat | 1228 - 1278 | IPR001680-5 |
| repeat | WD40 repeat | 1317 - 1358 | IPR001680-6 |
| active_site | Serine/threonine-protein kinase, active site | 144 - 156 | IPR008271 |
| repeat | HEAT, type 2 | 463 - 493 | IPR021133 |
Functions
| Description | ||
|---|---|---|
| EC Number | 2.7.11.1 | Protein-serine/threonine kinases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
10 GO annotations of cellular component
| Name | Definition |
|---|---|
| autophagosome | A double-membrane-bounded compartment that engulfs endogenous cellular material as well as invading microorganisms to target them to the lytic vacuole/lysosome for degradation as part of macroautophagy. |
| axoneme | The bundle of microtubules and associated proteins that forms the core of cilia (also called flagella) in eukaryotic cells and is responsible for their movements. |
| cytosol | The part of the cytoplasm that does not contain organelles but which does contain other particulate matter, such as protein complexes. |
| intracellular membrane-bounded organelle | Organized structure of distinctive morphology and function, bounded by a single or double lipid bilayer membrane and occurring within the cell. Includes the nucleus, mitochondria, plastids, vacuoles, and vesicles. Excludes the plasma membrane. |
| late endosome | A prelysosomal endocytic organelle differentiated from early endosomes by lower lumenal pH and different protein composition. Late endosomes are more spherical than early endosomes and are mostly juxtanuclear, being concentrated near the microtubule organizing center. |
| microtubule cytoskeleton | The part of the cytoskeleton (the internal framework of a cell) composed of microtubules and associated proteins. |
| nucleus-vacuole junction | An organelle membrane contact site formed between the vacuole membrane and the outer nuclear membrane. In S. cerevisiae these contacts are mediated through direct physical interaction between Vac8p and Nvj1p. |
| phosphatidylinositol 3-kinase complex, class III | A phosphatidylinositol 3-kinase complex that contains a catalytic class III phosphoinositide 3-kinase (PI3K) subunit bound to a regulatory (adaptor) subunit. Additional adaptor proteins may be present. Class III PI3Ks have a substrate specificity restricted to phosphatidylinositol (PI). |
| phosphatidylinositol 3-kinase complex, class III, type I | A class III phosphatidylinositol 3-kinase complex that is involved in autophagy. In budding yeast, this complex consists of Vps30p, Vps34p, Apg14p and Vps15p. |
| phosphatidylinositol 3-kinase complex, class III, type II | A class III phosphatidylinositol 3-kinase complex that is involved in vacuolar protein sorting (VPS) via endosomes. In budding yeast, this complex consists of Vps30p, Vps34p, Vps38 and Vps15p. |
3 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| protein serine kinase activity | Catalysis of the reactions: ATP + protein serine = ADP + protein serine phosphate. |
| protein serine/threonine kinase activity | Catalysis of the reactions: ATP + protein serine = ADP + protein serine phosphate, and ATP + protein threonine = ADP + protein threonine phosphate. |
15 GO annotations of biological process
| Name | Definition |
|---|---|
| autophagosome maturation | Removal of PI3P and Atg8/LC3 after the closure of the phagophore and before the fusion with the endosome/lysosome (e.g. mammals and insects) or vacuole (yeast), and that very likely destabilizes other Atg proteins and thus enables their efficient dissociation and recycling. |
| autophagy of peroxisome | The process in which peroxisomes are delivered to a type of vacuole and degraded in response to changing nutrient conditions. |
| cellular response to glucose starvation | Any process that results in a change in state or activity of a cell (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of deprivation of glucose. |
| early endosome to late endosome transport | The directed movement of substances, in membrane-bounded vesicles, from the early sorting endosomes to the late sorting endosomes; transport occurs along microtubules and can be experimentally blocked with microtubule-depolymerizing drugs. |
| late endosome to vacuole transport | The directed movement of substances from late endosomes to the vacuole. In yeast, after transport to the prevacuolar compartment, endocytic content is delivered to the late endosome and on to the vacuole. This pathway is analogous to endosome to lysosome transport. |
| macroautophagy | The major inducible pathway for the general turnover of cytoplasmic constituents in eukaryotic cells, it is also responsible for the degradation of active cytoplasmic enzymes and organelles during nutrient starvation. Macroautophagy involves the formation of double-membrane-bounded autophagosomes which enclose the cytoplasmic constituent targeted for degradation in a membrane-bounded structure. Autophagosomes then fuse with a lysosome (or vacuole) releasing single-membrane-bounded autophagic bodies that are then degraded within the lysosome (or vacuole). Some types of macroautophagy, e.g. pexophagy, mitophagy, involve selective targeting of the targets to be degraded. |
| phosphatidylinositol-3-phosphate biosynthetic process | The chemical reactions and pathways resulting in the formation of phosphatidylinositol-3-phosphate, a phosphatidylinositol monophosphate carrying the phosphate group at the 3-position. |
| positive regulation of phosphatidylinositol 3-kinase activity | Any process that activates or increases the frequency, rate or extent of phosphatidylinositol 3-kinase activity. |
| protein phosphorylation | The process of introducing a phosphate group on to a protein. |
| protein targeting to lysosome | The process of directing proteins towards the lysosome using signals contained within the protein. |
| protein targeting to vacuole | The process of directing proteins towards the vacuole, usually using signals contained within the protein. |
| receptor catabolic process | The chemical reactions and pathways resulting in the breakdown of a receptor molecule, a macromolecule that undergoes combination with a hormone, neurotransmitter, drug or intracellular messenger to initiate a change in cell function. |
| regulation of autophagy | Any process that modulates the frequency, rate or extent of autophagy. Autophagy is the process in which cells digest parts of their own cytoplasm. |
| regulation of cytokinesis | Any process that modulates the frequency, rate or extent of the division of the cytoplasm of a cell and its separation into two daughter cells. |
| regulation of macroautophagy | Any process that modulates the frequency, rate or extent of macroautophagy. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MGNQLAGIAP | SQILSVESYF | SDIHDFEYDK | SLGSTRFFKV | ARAKHREGLV | VVKVFAIQDP |
| 70 | 80 | 90 | 100 | 110 | 120 |
| TLPLTSYKQE | LEELKIRLHS | AQNCLPFQKA | AEKASEKAAM | LFRQYVRDNL | YDRISTRPFL |
| 130 | 140 | 150 | 160 | 170 | 180 |
| NNIEKRWIAF | QILTAVDQAH | KSGVRHGDIK | TENVMVTSWN | WVLLTDFASF | KPTYLPEDNP |
| 190 | 200 | 210 | 220 | 230 | 240 |
| ADFNYFFDTS | RRRTCYIAPE | RFVDGGMFAT | ELEYMRDPST | PLVDLNSNQR | ARGELKRAMD |
| 250 | 260 | 270 | 280 | 290 | 300 |
| IFSAGCVIAE | LFTEGVPLFD | LSQLLAYRNG | HFFPEQVLNK | IEDRSIRDLV | TQMINREPEK |
| 310 | 320 | 330 | 340 | 350 | 360 |
| RLEAEDYLKQ | QRGNAFPEIF | YTFLQPYMAQ | FAKETFLSAD | ERILVIRKDL | GNIIHNLCGH |
| 370 | 380 | 390 | 400 | 410 | 420 |
| DLPEKAEGES | RASGLVVLVS | VITSCLQTLK | SCDSKLAALE | LILHLAPRLS | VEILLDRITP |
| 430 | 440 | 450 | 460 | 470 | 480 |
| YLLHFSNDSV | PRVRAEALRT | LTKVLALVQE | VPRNDVNIYP | EYILPGIAHL | AQDDATIVRL |
| 490 | 500 | 510 | 520 | 530 | 540 |
| AYAENIALLA | ETALRFLELV | QLKTLNMENE | PDNEEVDEAT | RPNGDYDTEL | QALHEMVQQK |
| 550 | 560 | 570 | 580 | 590 | 600 |
| VVTLLSDPEN | IVKQTLMESG | ITRLCVFFGR | QKANDVLLSH | MITFLNDKND | WHLRGAFFDS |
| 610 | 620 | 630 | 640 | 650 | 660 |
| IVGVAAYVGW | QSSSILKPLL | QQGLSDAEEF | VIVKALNALT | CMCQLGLLQK | PHVYEFASDI |
| 670 | 680 | 690 | 700 | 710 | 720 |
| APFLCHPNLW | IRYGAVGFIT | VVAHQISTAD | VYCKLMPYLD | PYITQPVIQI | ERKLVLLSVL |
| 730 | 740 | 750 | 760 | 770 | 780 |
| KEPVSRSIFD | YALRSKDIAS | LFRHLHMRQK | KRNGSLLDCP | PPEDPTIAQL | LKKLLSQGMT |
| 790 | 800 | 810 | 820 | 830 | 840 |
| EEEEDKLLAL | KDFMMKSNRA | KANAVDQSHL | HDSSQKGVID | LAALGITGRQ | VDLVKTKQEP |
| 850 | 860 | 870 | 880 | 890 | 900 |
| DEKRARKHVK | QDSNVNEEWK | SMFGSLEPPN | IPQALPKTSD | HEVVQPGKPP | RSESSAGICV |
| 910 | 920 | 930 | 940 | 950 | 960 |
| PLSTSPQVSE | AAHIPSKKPV | IPVVSSTVLP | STYQIRITTC | KTELQQLIQQ | KREQCNAERI |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| AKQMMENAEW | ESKPPPPGWR | PKGLLVAHLH | EHKSAVNRIR | VSDEHLLFAT | CSNDGTVKIW |
| 1030 | 1040 | 1050 | 1060 | 1070 | 1080 |
| NSQKMEGKTT | TTRSILTYSR | IGGRVKTLTF | CQGSHYLAIA | SDNGAVQLLG | IEASKLPKSP |
| 1090 | 1100 | 1110 | 1120 | 1130 | 1140 |
| KIHPLQSRIL | DQKEDGCVVD | MHHFNSGAQS | VLAYATVNGS | LVGWDLRSSS | NAWTLKHDLK |
| 1150 | 1160 | 1170 | 1180 | 1190 | 1200 |
| SGLITSFAVD | IHQCWLCIGT | SSGAMACWDM | RFQLPISSHC | HPSRARIRRL | SMHPLYQSWV |
| 1210 | 1220 | 1230 | 1240 | 1250 | 1260 |
| IAAVQGNNEV | SMWDMETGDR | RLTLWASSAP | PLSELQPSPH | SVHGIYCSPA | DGNPILLTAG |
| 1270 | 1280 | 1290 | 1300 | 1310 | 1320 |
| SDMKIRFWDL | VSPERSYVVA | GSTGSPSVSY | YKKIIEGTEV | VQEIQNKQKV | GPSDDTPRRG |
| 1330 | 1340 | 1350 | |||
| PESLPVGHHD | IITDIATFQT | TQGFIVTASR | DGIVKVWK |