Q8R979
Gene name |
rgy |
Protein name |
Reverse gyrase |
Names |
|
Species |
Caldanaerobacter subterraneus subsp. tengcongensis (strain DSM 15242 / JCM 11007 / NBRC 100824 / MB4) (Thermoanaerobacter tengcongensis) |
KEGG Pathway |
tte:TTE1745 |
EC number |
|
Protein Class |
|
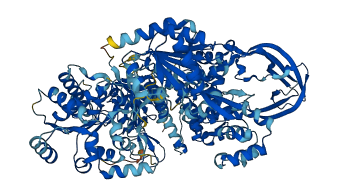
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q8R979
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q8R979-F1 | Predicted | AlphaFoldDB |
No variants for Q8R979
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q8R979 | |||||
No associated diseases with Q8R979
9 regional properties for Q8R979
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | DNA topoisomerase, type IA, domain 2 | 703 - 791 | IPR003601 |
| domain | DNA topoisomerase, type IA, DNA-binding domain | 817 - 1066 | IPR003602 |
| domain | TOPRIM domain | 555 - 712 | IPR006171 |
| domain | DEAD/DEAH box helicase domain | 88 - 270 | IPR011545 |
| domain | DNA topoisomerase, type IA, central | 676 - 689 | IPR013497-1 |
| domain | DNA topoisomerase, type IA, central | 728 - 1114 | IPR013497-2 |
| domain | Helicase superfamily 1/2, ATP-binding domain | 76 - 302 | IPR014001 |
| domain | Reverse gyrase, TOPRIM domain | 555 - 724 | IPR034142 |
| domain | Reverse gyrase, zinc finger | 10 - 50 | IPR040569 |
No GO annotations of cellular component
| Name | Definition |
|---|---|
| No GO annotations for cellular component |
6 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP hydrolysis activity | Catalysis of the reaction: ATP + H2O = ADP + H+ phosphate. ATP hydrolysis is used in some reactions as an energy source, for example to catalyze a reaction or drive transport against a concentration gradient. |
| DNA binding | Any molecular function by which a gene product interacts selectively and non-covalently with DNA (deoxyribonucleic acid). |
| DNA helicase activity | Unwinding of a DNA helix, driven by ATP hydrolysis. |
| DNA topoisomerase type II (double strand cut, ATP-hydrolyzing) activity | Catalysis of a DNA topological transformation by transiently cleaving a pair of complementary DNA strands to form a gate through which a second double-stranded DNA segment is passed, after which the severed strands in the first DNA segment are rejoined, driven by ATP hydrolysis. The enzyme changes the linking number in multiples of 2. |
| zinc ion binding | Binding to a zinc ion (Zn). |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| DNA topological change | The process in which a transformation is induced in the topological structure of a double-stranded DNA helix, resulting in a change in linking number. |
| DNA unwinding involved in DNA replication | The process in which interchain hydrogen bonds between two strands of DNA are broken or 'melted', generating unpaired template strands for DNA replication. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MALATGAKYY | HSCINCGGIN | TDTRNEKGLP | CEVCLPFEDG | DVLKGLKLNN | SLKGYEKYWN |
| 70 | 80 | 90 | 100 | 110 | 120 |
| LNQQYKEFEE | FFFSKINKKP | TGYQRFWAKR | LLLSKSFTLV | APTGVGKTTF | GLISALWIAK |
| 130 | 140 | 150 | 160 | 170 | 180 |
| KGGKVALVFP | TVSLVEQAAK | RLIEFSKEDE | DVNILFYTSS | LKKKEREKFE | KNFSEGNYDI |
| 190 | 200 | 210 | 220 | 230 | 240 |
| LVISSQFISK | RKEQLSQKVF | DLVFVDDVDA | VLKSSKNIDT | LLNMIGISQK | AIDSTLDNLK |
| 250 | 260 | 270 | 280 | 290 | 300 |
| KGNNSDKIQI | EEKAPKGRLI | VSSATAKPKG | IKPLLFRELL | GFEIGRFTTS | ARNITNVRIK |
| 310 | 320 | 330 | 340 | 350 | 360 |
| EKSLEKLLYI | INLLKDGILL | FVPTEEEGKE | IANYLEEHGV | KLGKTWEDFE | KSFEKFKEGS |
| 370 | 380 | 390 | 400 | 410 | 420 |
| LQLLCGIYSY | YGKLVRGIDL | PLRIKFAVFW | GTPSFKFSTK | LENAPRFILE | RNFQDYLENN |
| 430 | 440 | 450 | 460 | 470 | 480 |
| PKLKAYFKDL | QRLSTEKLRK | SVEKYISPET | WEKLIQKNFP | TTKFDKEKNL | IVIPDVYTYI |
| 490 | 500 | 510 | 520 | 530 | 540 |
| QASGRTSRIF | GTSLTKGISI | LFEEDDSLFE | LLKARLLYLT | EEEWTEEGEI | EHLVKEAEET |
| 550 | 560 | 570 | 580 | 590 | 600 |
| RKAISTDSSS | KDMKSRMIIV | ESPTKAQTIS | KFLEKSSTRR | YGSLMVHESI | TQEGILLLTA |
| 610 | 620 | 630 | 640 | 650 | 660 |
| SKGHLYDLET | KTGLHGVEIN | DGRFIPYYNS | IKRCSSCGAQ | FTDELPRCPY | CNSDKIDDKK |
| 670 | 680 | 690 | 700 | 710 | 720 |
| KILEALRDIA | MEVDEVIIAT | DPDVEGEKIG | WDISQYIKPV | NKNVQRIEMH | EITKFGFDKA |
| 730 | 740 | 750 | 760 | 770 | 780 |
| IRNRRNCDVN | LVKSQIVRRI | EDRWVGFELS | LRLQKNFQNS | NLSAGRVQST | VLGWILEKEI |
| 790 | 800 | 810 | 820 | 830 | 840 |
| EHSKSKKTVT | QFTLDNGFKF | EVDGKIDVDE | VEVEIVEEKE | QALSPLPPFN | TPSLLTAASQ |
| 850 | 860 | 870 | 880 | 890 | 900 |
| QFKLPVQQIM | EILQTLFELG | FITYHRTDST | RISSTGQKIA | RSYLEKIGKI | TLLSEREWGK |
| 910 | 920 | 930 | 940 | 950 | 960 |
| EGAHEAIRPV | KPISPEELSE | FITEKIAAYL | SPMHIKVYSL | IFNRFMASQM | TSPVVINQKI |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| LIKNGSFQVE | REVPVKLQEE | GWNIFNPITV | YTPFEEKKYS | VVSKRTYTTH | TVPLFTQASL |
| 1030 | 1040 | 1050 | 1060 | 1070 | 1080 |
| IEEMQKRNIG | RPSTYAKIVD | ILFKRKYIIE | DVYKRLRTTA | LGRKVYSYLS | ERYMNYINEE |
| 1090 | 1100 | 1110 | |||
| TTRQLEKLME | SVETGEKDYQ | SVLKNLYEEL | NEILIKN |