Q8PXE1
Gene name |
fae-hps |
Protein name |
Bifunctional enzyme Fae/Hps |
Names |
|
Species |
Methanosarcina mazei (strain ATCC BAA-159 / DSM 3647 / Goe1 / Go1 / JCM 11833 / OCM 88) (Methanosarcina frisia) |
KEGG Pathway |
mma:MM_1279 |
EC number |
4.1.2.43: Aldehyde-lyases |
Protein Class |
|
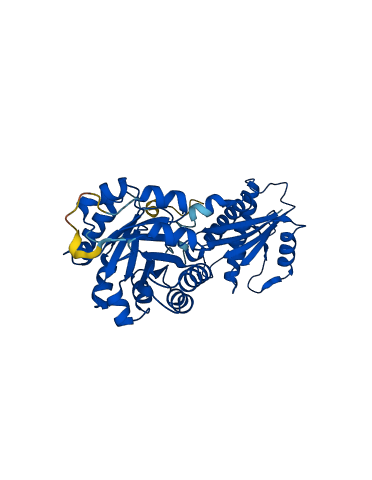
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q8PXE1
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q8PXE1-F1 | Predicted | AlphaFoldDB |
No variants for Q8PXE1
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q8PXE1 | |||||
No associated diseases with Q8PXE1
No regional properties for Q8PXE1
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| No domain, repeats, and functional sites for Q8PXE1 | |||
Functions
| Description | ||
|---|---|---|
| EC Number | 4.1.2.43 | Aldehyde-lyases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
No GO annotations of cellular component
| Name | Definition |
|---|---|
| No GO annotations for cellular component |
4 GO annotations of molecular function
| Name | Definition |
|---|---|
| carbon-nitrogen lyase activity | Catalysis of the release of ammonia or one of its derivatives, with the formation of a double bond or ring. Enzymes with this activity may catalyze the actual elimination of the ammonia, amine or amide, e.g. CH-CH(-NH-R) = C=CH- + NH2-R. Others, however, catalyze elimination of another component, e.g. water, which is followed by spontaneous reactions that lead to breakage of the C-N bond, e.g. L-serine ammonia-lyase (EC:4.3.1.17), so that the overall reaction is C(-OH)-CH(-NH2) = CH2-CO- + NH3, i.e. an elimination with rearrangement. The sub-subclasses of EC:4.3 are the ammonia-lyases (EC:4.3.1), lyases acting on amides, amidines, etc. (EC:4.3.2), the amine-lyases (EC:4.3.3), and other carbon-nitrogen lyases (EC:4.3.99). |
| hexulose-6-phosphate synthase activity | Catalysis of the reaction: D-ribulose 5-phosphate + formaldehyde = D-arabino-3-hexulose 6-phosphate. |
| hydro-lyase activity | Catalysis of the cleavage of a carbon-oxygen bond by elimination of water. |
| orotidine-5'-phosphate decarboxylase activity | Catalysis of the reaction: H(+) + orotidine 5'-phosphate = CO(2) + UMP. |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| 'de novo' pyrimidine nucleobase biosynthetic process | The chemical reactions and pathways resulting in the formation of pyrimidine nucleobases, 1,3-diazine, organic nitrogenous bases, beginning with the synthesis of a pyrimidine ring from simpler precursors. |
| carbohydrate biosynthetic process | The chemical reactions and pathways resulting in the formation of carbohydrates, any of a group of organic compounds based of the general formula Cx(H2O)y. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MFQIGEALMG | QGSELAHVDL | MIGDKGGPVG | QAFANGLTQL | SAGHTPLLSV | IRPNLPPKPS |
| 70 | 80 | 90 | 100 | 110 | 120 |
| TLIIPKVTVK | NMDQAARIFG | PAQSAVAKAV | ADSVEEGVIP | KDQVEDLVIV | ASVFIHPEAQ |
| 130 | 140 | 150 | 160 | 170 | 180 |
| DYNKIYRYNY | GATKLAIKRA | LEGFPDIDTV | LEESNKSTHA | IMGFKVTRLW | DPPYLQIAFD |
| 190 | 200 | 210 | 220 | 230 | 240 |
| NPNLEFVLSA | ISEIPKSDHV | IIEAGTPLIK | RYGTDVISKI | RQVRPDAFIV | ADLKTLDTGN |
| 250 | 260 | 270 | 280 | 290 | 300 |
| LEARMVADAA | GDAIVVSALA | PISTIDKLIE | EAHKTGIYAV | MDTLNQQDPI | SVLKQLKVMP |
| 310 | 320 | 330 | 340 | 350 | 360 |
| DVIELHRGID | IEGTEHAWGN | IGEIKKIAPK | ALVAVAGGVR | LDKVPVALSQ | GADILVVGRA |
| 370 | 380 | 390 | |||
| ITNAKDVREM | AEQFINSLNK | PEIDQFRVMT | DF |