Q8K9U9
Gene name |
thrA (BUsg_188) |
Protein name |
Bifunctional aspartokinase/homoserine dehydrogenase |
Names |
AK-HD |
Species |
Buchnera aphidicola subsp Schizaphis graminum (strain Sg) |
KEGG Pathway |
bas:BUsg_188 |
EC number |
1.1.1.3: With NAD(+) or NADP(+) as acceptor |
Protein Class |
|
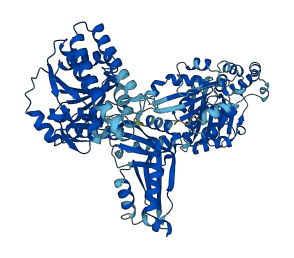
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q8K9U9
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q8K9U9-F1 | Predicted | AlphaFoldDB |
No variants for Q8K9U9
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q8K9U9 | |||||
No associated diseases with Q8K9U9
8 regional properties for Q8K9U9
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Aspartate/glutamate/uridylate kinase | 3 - 283 | IPR001048 |
| domain | Aspartate kinase | 4 - 459 | IPR001341 |
| domain | Homoserine dehydrogenase, catalytic | 613 - 810 | IPR001342 |
| domain | ACT domain | 319 - 400 | IPR002912 |
| domain | Aspartate/homoserine dehydrogenase, NAD-binding | 471 - 605 | IPR005106 |
| conserved_site | Aspartate kinase, conserved site | 3 - 11 | IPR018042 |
| conserved_site | Homoserine dehydrogenase, conserved site | 659 - 681 | IPR019811 |
| domain | Bifunctional aspartokinase/homoserine dehydrogenase, N-terminal catalytic domain | 1 - 295 | IPR041743 |
Functions
| Description | ||
|---|---|---|
| EC Number | 1.1.1.3 | With NAD(+) or NADP(+) as acceptor |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
No GO annotations of cellular component
| Name | Definition |
|---|---|
| No GO annotations for cellular component |
4 GO annotations of molecular function
| Name | Definition |
|---|---|
| aspartate kinase activity | Catalysis of the reaction: L-aspartate + ATP = 4-phospho-L-aspartate + ADP + H(+). |
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| homoserine dehydrogenase activity | Catalysis of the reaction: L-homoserine + NADP+ = L-aspartate-4-semialdehyde + NADPH + H+. |
| NADP binding | Binding to nicotinamide-adenine dinucleotide phosphate, a coenzyme involved in many redox and biosynthetic reactions; binding may be to either the oxidized form, NADP+, or the reduced form, NADPH. |
3 GO annotations of biological process
| Name | Definition |
|---|---|
| lysine biosynthetic process via diaminopimelate | The chemical reactions and pathways resulting in the formation of lysine, via the intermediate diaminopimelate. |
| phosphorylation | The process of introducing a phosphate group into a molecule, usually with the formation of a phosphoric ester, a phosphoric anhydride or a phosphoric amide. |
| threonine biosynthetic process | The chemical reactions and pathways resulting in the formation of threonine (2-amino-3-hydroxybutyric acid), a polar, uncharged, essential amino acid found in peptide linkage in proteins. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MKLLKFGGTS | LANAKKFLCV | ADIIEKKNKK | EQIAVVLSAP | AKITNYLATI | IENKIDDEVL |
| 70 | 80 | 90 | 100 | 110 | 120 |
| KKINLAKNIF | IELIQDIKRI | QPLFPYENTK | STIEIEFNKL | KKIINGILLI | KQCPEGIKPI |
| 130 | 140 | 150 | 160 | 170 | 180 |
| IISRGEILSV | DIMKNILQSR | NHEVTILNPV | TNLLSIGNYL | DSTIDIKESK | KRIKKINIDQ |
| 190 | 200 | 210 | 220 | 230 | 240 |
| KNIILMAGFI | AGNKEGELVV | LGRNGSDYSA | AILASCLNAK | CCEIWTDVDG | VLTADPRIVS |
| 250 | 260 | 270 | 280 | 290 | 300 |
| NTYLLDYISY | QEAMELSYFG | AKVLHPRTIE | PISQFQIPCV | IKNTNNTESK | GTWIGKENNP |
| 310 | 320 | 330 | 340 | 350 | 360 |
| SDNSLKGVTY | LDNIIMFNIS | GSCLKDSGNT | IARIFTILSR | ESMKIILIIQ | SSSENQINFC |
| 370 | 380 | 390 | 400 | 410 | 420 |
| TFEKDIDYIL | LILKKEFTLE | IKEGLLNDFN | IVKNLTILSV | IGSNISEKNN | IASKIFSSLG |
| 430 | 440 | 450 | 460 | 470 | 480 |
| SSKINVLAIA | HGSSKHSISI | VIKKENLLQG | IQNIHNTLFF | KKTIINVFLI | GIGGVGKALL |
| 490 | 500 | 510 | 520 | 530 | 540 |
| KQILKQEKFL | DQKNIKIQFR | MIANSKKLLF | LKNSINLNNW | EENFKKSKEK | FNLTILNELL |
| 550 | 560 | 570 | 580 | 590 | 600 |
| KNTCDSNSVI | IDCTSDYILS | KQYISFIKKG | FHIITSNKKA | NTDSLKYYSE | IRTTALKENK |
| 610 | 620 | 630 | 640 | 650 | 660 |
| KFLYETNVGA | GLPVINTLQS | LFSTGDCLIS | FKGILSGSLS | FIFGKLEEGV | LLSEATKEAK |
| 670 | 680 | 690 | 700 | 710 | 720 |
| KLGFTEPNPF | DDLSGIDVAR | KLLVLAREIG | YSIELKDISI | EPILPERFKK | YQNSEEFLFK |
| 730 | 740 | 750 | 760 | 770 | 780 |
| LKELDSFFSE | RVNKARDIGN | VLRFIGSIEK | NGKCSVKIEE | INSNNPLYKV | KNGENALTFY |
| 790 | 800 | 810 | |||
| TNYYQPIPLV | LRGYGAGNDV | TASGVFSDLL | RIIL |