Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
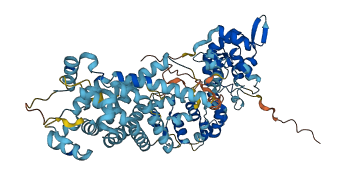
Autoinhibited structure

Activated structure
1 structures for Q8HXW2
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q8HXW2-F1 | Predicted | AlphaFoldDB |
No variants for Q8HXW2
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q8HXW2 | |||||
No associated diseases with Q8HXW2
4 regional properties for Q8HXW2
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | EF-hand domain | 87 - 122 | IPR002048 |
| repeat | Mitochondrial substrate/solute carrier | 326 - 422 | IPR018108-1 |
| repeat | Mitochondrial substrate/solute carrier | 426 - 512 | IPR018108-2 |
| repeat | Mitochondrial substrate/solute carrier | 518 - 607 | IPR018108-3 |
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| integral component of membrane | The component of a membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
| mitochondrial inner membrane | The inner, i.e. lumen-facing, lipid bilayer of the mitochondrial envelope. It is highly folded to form cristae. |
| mitochondrion | A semiautonomous, self replicating organelle that occurs in varying numbers, shapes, and sizes in the cytoplasm of virtually all eukaryotic cells. It is notably the site of tissue respiration. |
4 GO annotations of molecular function
| Name | Definition |
|---|---|
| 3-sulfino-L-alanine: proton, glutamate antiporter activity | Enables the transfer of a solute or solutes from one side of a membrane to the other according to the reaction: 3-sulfino-L-alanine (cysteinesulfinate) (out) + H(+)(in) + L-glutamate(in) = 3-sulfino-L-alanine(in) + H(+)(out) + L-glutamate(out). |
| aspartate:glutamate, proton antiporter activity | Enables the transfer of a solute or solutes from one side of a membrane to the other according to the reaction: H(+)(out) + L-aspartate(in) + L-glutamate(out) = H(+)(in) + L-aspartate(out) + L-glutamate(in). |
| calcium ion binding | Binding to a calcium ion (Ca2+). |
| identical protein binding | Binding to an identical protein or proteins. |
6 GO annotations of biological process
| Name | Definition |
|---|---|
| aspartate transmembrane transport | The process in which aspartate is transported across a lipid bilayer, from one side of a membrane to the other. |
| ATP biosynthetic process | The chemical reactions and pathways resulting in the formation of ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| cellular respiration | The enzymatic release of energy from inorganic and organic compounds (especially carbohydrates and fats) which either requires oxygen (aerobic respiration) or does not (anaerobic respiration). |
| L-glutamate transmembrane transport | The directed movement of L-glutamate across a membrane. |
| malate-aspartate shuttle | The process of transferring reducing equivalents from the cytosol into the mitochondria; NADH is used to synthesise malate in the cytosol; this compound is then transported into the mitochondria where it is converted to oxaloacetate using NADH, the oxaloacetate reacts with gluamate to form aspartate, and the aspartate then returns to the cytosol to complete the cycle. |
| response to calcium ion | Any process that results in a change in state or activity of a cell or an organism (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of a calcium ion stimulus. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MAAAKVALTK | RADPAELRTI | FLKYASIEKN | GEFFTSPNDF | VTRYLNIFGE | SQPNPKTVEL |
| 70 | 80 | 90 | 100 | 110 | 120 |
| LSGVADQTKD | GLISFQEFVA | FESVLCAPDA | LFMVAFQLFD | KAGKGEVTFE | DVKQVFGQTT |
| 130 | 140 | 150 | 160 | 170 | 180 |
| IHQHIPFNWD | SEFVQLHFGK | ERKRHLTYAE | FTQFLLEIQL | EHAKQAFVQR | DNASTGRVTA |
| 190 | 200 | 210 | 220 | 230 | 240 |
| IDFRDIMVTI | RPHVLTPFVE | ECLVAAAGGT | TSHQVSFSYF | NGFNSLLNNM | ELTRKIYSTL |
| 250 | 260 | 270 | 280 | 290 | 300 |
| AGNRKDVEVT | KEEFVLAAQK | FGQVTPMEVD | ILFRLADLYE | PRGRMTLADI | ERIAPLEEGT |
| 310 | 320 | 330 | 340 | 350 | 360 |
| LPFNLAEAQR | QKASGDSARP | VLLQVAESAY | RFGLGSVAGA | VGATAVYPID | LVKTRMQNQR |
| 370 | 380 | 390 | 400 | 410 | 420 |
| STGSFVGELM | YKNSFDCFKK | VLRYEGFFGL | YRGLLPQLLG | VAPEKAIKLT | VNDFVRDKFM |
| 430 | 440 | 450 | 460 | 470 | 480 |
| HKDGSVPLAA | EILAGGCAGG | SQVIFTNPLE | IVKIRLQVAG | EITTGPRVSA | LSVVRDLGFF |
| 490 | 500 | 510 | 520 | 530 | 540 |
| GIYKGAKACF | LRDIPFSAIY | FPCYAHARAS | FANEDGQVSP | GSLLLAGAIA | GMPAASLVTP |
| 550 | 560 | 570 | 580 | 590 | 600 |
| ADVIKTRLQV | AARAGQTTYS | GVIDCFKKIL | REEGPKALWK | GAARVFRSSP | QFGVTLLTYE |
| 610 | 620 | 630 | 640 | 650 | 660 |
| LLQRWFYIDF | GGVKPMGSEP | VPKSRINLPA | PNPDHVGGYK | LAVATFAGIE | NKFGLYLPLF |
| 670 | |||||
| KPSVPTSEAI | GGGP |