Q6CSR1
Gene name |
MSH3 (KLLA0C18590g) |
Protein name |
DNA mismatch repair protein MSH3 |
Names |
MutS protein homolog 3 |
Species |
Kluyveromyces lactis (strain ATCC 8585 / CBS 2359 / DSM 70799 / NBRC 1267 / NRRL Y-1140 / WM37) (Yeast) (Candida sphaerica) |
KEGG Pathway |
kla:KLLA0_C18590g |
EC number |
|
Protein Class |
|
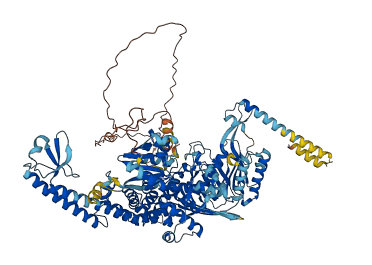
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q6CSR1
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q6CSR1-F1 | Predicted | AlphaFoldDB |
No variants for Q6CSR1
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q6CSR1 | |||||
No associated diseases with Q6CSR1
5 regional properties for Q6CSR1
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | DNA mismatch repair protein MutS, C-terminal | 795 - 988 | IPR000432 |
| domain | DNA mismatch repair protein MutS-like, N-terminal | 151 - 269 | IPR007695 |
| domain | DNA mismatch repair protein MutS, core | 432 - 779 | IPR007696 |
| domain | DNA mismatch repair protein MutS, connector domain | 293 - 374 | IPR007860 |
| domain | DNA mismatch repair protein MutS, clamp | 624 - 701 | IPR007861 |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| MutSbeta complex | A heterodimer involved in binding to and correcting insertion/deletion mutations. In human the complex consists of two subunits, MSH2 and MSH3. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP-dependent DNA damage sensor activity | A molecule that recognises toxic DNA structures, and initiates a signalling response, driven by ATP hydrolysis. |
| double-strand/single-strand DNA junction binding | Binding to a DNA segment that contains double-stranded DNA flanked by a region of single-stranded DNA. |
| heteroduplex DNA loop binding | Binding to a DNA segment containing a loop. A loop occurs when DNA contains a large insertion or deletion that causes a region of unpaired single-stranded DNA to loop out, while the rest of the DNA is in a paired double-stranded configuration. |
| Y-form DNA binding | Binding to a DNA segment shaped like a Y. This shape occurs when DNA contains a region of paired double-stranded DNA on one end and a region of unpaired DNA strands on the opposite end. |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| meiotic mismatch repair | A system for the identification and correction of base-base mismatches, small insertion-deletion loops, and regions of heterology that are present in duplex DNA formed with strands from two recombining molecules. Correction of the mismatch can result in non-Mendelian segregation of alleles following meiosis. |
| mitotic recombination | The exchange, reciprocal or nonreciprocal, of genetic material between one DNA molecule and a homologous DNA region that occurs during mitotic cell cycles. |
| removal of nonhomologous ends | The removal of nonhomologous sequences at the broken 3' single-strand DNA end before DNA repair synthesis can occur. |
| replication fork arrest | Any process that stops, prevents, or reduces the frequency, rate or extent of DNA replication by impeding the progress of the DNA replication fork. Replication fork arrest is one of the 'quality control' processes ensuring that DNA-dependent DNA replication occurs correctly. DNA replication fork arrest during DNA-dependent DNA replication is not known to occur outside of cases where a replication error needs to be prevented or corrected. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MYQPTISHFF | KSSQPSSQTD | TRQDEDQRLD | IESHEQRGGA | NMNKDELINI | LGSDSESDQD |
| 70 | 80 | 90 | 100 | 110 | 120 |
| LDEDLDQDQN | NNQDQDQEQD | RDLASKANNG | RSTLSAERIE | RRPDFNEKLK | TIMRKRNAGS |
| 130 | 140 | 150 | 160 | 170 | 180 |
| MINTGSDDEN | DDNDDVKSTK | RTKANNKKLT | ELDQQFKELK | LKHMDTILCV | RVGYKYKFFA |
| 190 | 200 | 210 | 220 | 230 | 240 |
| KDAEIVSNIL | QIKLVPGKKT | LDESDPNDRN | YRKFQYCSIP | DTRLHVHLQR | LVFFNYKVAV |
| 250 | 260 | 270 | 280 | 290 | 300 |
| VEQTETSALK | KNNNSGSLFT | REIKNIFTKV | SYGINETFDK | SEDRILGDLT | SVWAISINET |
| 310 | 320 | 330 | 340 | 350 | 360 |
| SKMRKVNLIS | VQLNSGEIVH | DQFSDDILLN | VNLEARIRYL | NPTEIITEEE | LPPSIRTIFT |
| 370 | 380 | 390 | 400 | 410 | 420 |
| KLNQDIQFYQ | SHKEACPNLF | DALQGLDLNN | ELKRLLSVLH | SYLSTFENTK | VLYFASNYSS |
| 430 | 440 | 450 | 460 | 470 | 480 |
| FTAKNFMVLP | RNTIESLEIF | ENSTTNKTNG | SLLWVMDHTR | TQFGYRLLRK | WISKPLIDLK |
| 490 | 500 | 510 | 520 | 530 | 540 |
| SILDRQDAIT | CIMKEVHSIF | FESFNELLRK | SIDLERALNR | IAYGSTSRKE | VYFFLKQIAT |
| 550 | 560 | 570 | 580 | 590 | 600 |
| FASLFKSHHT | FIHDQLHKEN | SALRKTSCLL | FNILQNLDAF | FSATDLPLFL | QMINVDAALD |
| 610 | 620 | 630 | 640 | 650 | 660 |
| KDSHKNVIEF | FNLNKYDFPE | GLLHKYRDIE | EVKTELDDEL | QNIKRVLKRP | TLSYKDTKDY |
| 670 | 680 | 690 | 700 | 710 | 720 |
| LIEVRNTQAK | TVPSNWVKVN | STKAVSRFRT | PKTEELVGKL | LYHNDLLNLL | AEDEFKRFLQ |
| 730 | 740 | 750 | 760 | 770 | 780 |
| RIVDRYAEIK | TCINNLATYD | CILSLAATSS | NVNYVKPKLT | ELHQKVKVKN | GRNPIIESLD |
| 790 | 800 | 810 | 820 | 830 | 840 |
| VNYVPNDVLM | SSNSGKINII | TGPNMGGKSS | YIRQVALLVI | MTQIGCYIPA | DSAEMSICDR |
| 850 | 860 | 870 | 880 | 890 | 900 |
| IFTRIGSHDD | LLNAKSTFQV | EMSEVLHILN | SSTPRSLLLL | DEVGRGTGTH | DGLSISFAIL |
| 910 | 920 | 930 | 940 | 950 | 960 |
| NYFVYLADNC | PLVLFITHYS | ALCQIDSKLI | ANYHMSYIEK | HQPGEKWTNV | IFLYKLVLGQ |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| AHNSYGFNVA | KLSNIPTEII | NRAFEVSEEK | ILSSKHHNFL | EIMKALKRVN | ERKLNKEALK |
| KIQAFIEDI |