Q6CNR9
Gene name |
PIM1 |
Protein name |
Lon protease homolog, mitochondrial |
Names |
|
Species |
Kluyveromyces lactis (strain ATCC 8585 / CBS 2359 / DSM 70799 / NBRC 1267 / NRRL Y-1140 / WM37) (Yeast) (Candida sphaerica) |
KEGG Pathway |
kla:KLLA0_E10407g |
EC number |
3.4.21.53: Serine endopeptidases |
Protein Class |
|
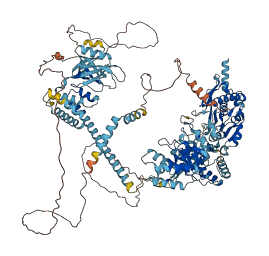
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q6CNR9
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q6CNR9-F1 | Predicted | AlphaFoldDB |
No variants for Q6CNR9
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q6CNR9 | |||||
No associated diseases with Q6CNR9
5 regional properties for Q6CNR9
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Lon protease, N-terminal domain | 184 - 448 | IPR003111 |
| domain | AAA+ ATPase domain | 594 - 740 | IPR003593 |
| domain | ATPase, AAA-type, core | 598 - 736 | IPR003959 |
| active_site | Peptidase S16, active site | 988 - 996 | IPR008268 |
| domain | Peptidase S16, Lon proteolytic domain | 877 - 1085 | IPR008269 |
Functions
| Description | ||
|---|---|---|
| EC Number | 3.4.21.53 | Serine endopeptidases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| mitochondrial chromosome | A chromosome found in the mitochondrion of a eukaryotic cell. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP hydrolysis activity | Catalysis of the reaction: ATP + H2O = ADP + H+ phosphate. ATP hydrolysis is used in some reactions as an energy source, for example to catalyze a reaction or drive transport against a concentration gradient. |
| ATP-dependent peptidase activity | Catalysis of the hydrolysis of peptide bonds, driven by ATP hydrolysis. |
| sequence-specific DNA binding | Binding to DNA of a specific nucleotide composition, e.g. GC-rich DNA binding, or with a specific sequence motif or type of DNA e.g. promotor binding or rDNA binding. |
| serine-type endopeptidase activity | Catalysis of the hydrolysis of internal, alpha-peptide bonds in a polypeptide chain by a catalytic mechanism that involves a catalytic triad consisting of a serine nucleophile that is activated by a proton relay involving an acidic residue (e.g. aspartate or glutamate) and a basic residue (usually histidine). |
6 GO annotations of biological process
| Name | Definition |
|---|---|
| cellular response to oxidative stress | Any process that results in a change in state or activity of a cell (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of oxidative stress, a state often resulting from exposure to high levels of reactive oxygen species, e.g. superoxide anions, hydrogen peroxide (H2O2), and hydroxyl radicals. |
| chaperone-mediated protein complex assembly | The aggregation, arrangement and bonding together of a set of components to form a protein complex, mediated by chaperone molecules that do not form part of the finished complex. |
| mitochondrial protein catabolic process | The chemical reactions and pathways resulting in the breakdown of a mitochondrial protein. This process is necessary to maintain the healthy state of mitochondria and is thought to occur via the induction of an intramitochondrial lysosome-like organelle that acts to eliminate the damaged oxidised mitochondrial proteins without destroying the mitochondrial structure. |
| oxidation-dependent protein catabolic process | The chemical reactions and pathways resulting in the breakdown of a protein or peptide by hydrolysis of its peptide bonds, initiated by the oxidation of one or more amino acid residues in the protein. |
| protein quality control for misfolded or incompletely synthesized proteins | The chemical reactions and pathways resulting in the breakdown of misfolded or attenuated proteins. |
| regulation of mitochondrial DNA metabolic process | Any process that modulates the frequency, rate or extent of mitochondrial DNA metabolic process. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MLRSSRSRLV | TRNILLRQFK | NGNNVRLMNA | TRFQHNGIVG | NEKLASDSQK | FVDESYHWMQ |
| 70 | 80 | 90 | 100 | 110 | 120 |
| YRKQMNDPVS | RQRLEQLESQ | WVKSIQLKQD | DKGKDIDQPE | SENRKKEEEQ | VPTEEKDNDT |
| 130 | 140 | 150 | 160 | 170 | 180 |
| AKESETSQQR | DSVAETQGPA | STSGGASGNG | ESSGNGSGDD | GNNGSGNGKP | SKNAKQPFPE |
| 190 | 200 | 210 | 220 | 230 | 240 |
| VYPQVMALPI | SRRPLFPGFY | KAVVISDERV | MKAIKDMSDR | QQPYIGAFLL | KDSTVDTDVI |
| 250 | 260 | 270 | 280 | 290 | 300 |
| HKADEVYNVG | VFAQVTSAFP | SKDEKTGAET | MTALLYPHRR | IKLDELIPPT | SEQNLKDESD |
| 310 | 320 | 330 | 340 | 350 | 360 |
| VSKSEGVENN | EQEVVKASLQ | KMENMKDVEE | DDDENLTGFL | KDYDVSLVNV | SNLADKEFNP |
| 370 | 380 | 390 | 400 | 410 | 420 |
| NSPVINALTS | EILKVFKEIS | QLNTMFREQI | ATFSASIQSA | TTNIFEEPAR | LADFAAAVSA |
| 430 | 440 | 450 | 460 | 470 | 480 |
| GEEEELQEIL | ESLDIEQRLE | KALTVLKKEL | MNAELQNKIS | KDVETKIQKR | QREYYLMEQL |
| 490 | 500 | 510 | 520 | 530 | 540 |
| KGIKRELGID | DGRDKLIESF | KDRVSKLQLP | ETVQKVFDDE | ITKLATLETS | QSEFGVIRNY |
| 550 | 560 | 570 | 580 | 590 | 600 |
| LDWITSLPWG | IISKEQYSIP | KAKKILDEDH | YGMKDVKDRI | LEFIAVGKLL | GKVDGKIICF |
| 610 | 620 | 630 | 640 | 650 | 660 |
| VGPPGVGKTS | IGKSIARSLN | RQFFRFSVGG | MTDVAEIKGH | RRTYIGALPG | RVIQALKKCQ |
| 670 | 680 | 690 | 700 | 710 | 720 |
| TQNPLILIDE | IDKIGHGGIH | GDPAAALLEL | LDPEQNNSFL | DNYMDIPIDL | SKVLFVCTAN |
| 730 | 740 | 750 | 760 | 770 | 780 |
| SLETIPRPLL | DRMEVIELTG | YVAEEKVKIA | ENYLSPSAKK | SAGLDNANVN | ITENAIVSLM |
| 790 | 800 | 810 | 820 | 830 | 840 |
| KHYCRESGVR | SLKKHIEKIY | RKAALNVVKQ | LSIDDKPMEN | EEVKDQKDIK | VKQSENKSSA |
| 850 | 860 | 870 | 880 | 890 | 900 |
| EASTVESTTE | ENELIKTQKS | HDNKGSLEVP | ETVSVTVDEN | NLKDYVGPPI | FTTDRLYEST |
| 910 | 920 | 930 | 940 | 950 | 960 |
| PPGVVMGLAW | TSMGGCAMYV | ESVLEQPLTH | STQPTLERTG | QLGDVMKESS | RLAYSFSKMY |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| LAKKFPENRF | FEVAKIHLHC | PEGATPKDGP | SAGVTMASSF | LSLALNKGLD | PTVAMTGELT |
| 1030 | 1040 | 1050 | 1060 | 1070 | 1080 |
| LTGKVLRIGG | LREKAVAAKR | SGAKTIIFPK | DNLSDWAELP | ENVKEGLEPL | AADWYEDVFQ |
| 1090 | 1100 | 1110 | |||
| RLFGDVDTNK | GNTVWSEDFK | KIDEKRNKET | K |