Q6CII8
Gene name |
RNA14 (KLLA0F26290g) |
Protein name |
mRNA 3'-end-processing protein RNA14 |
Names |
|
Species |
Kluyveromyces lactis (strain ATCC 8585 / CBS 2359 / DSM 70799 / NBRC 1267 / NRRL Y-1140 / WM37) (Yeast) (Candida sphaerica) |
KEGG Pathway |
kla:KLLA0_F26290g |
EC number |
|
Protein Class |
|
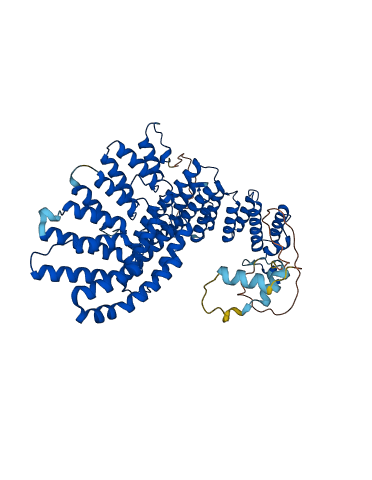
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
4 structures for Q6CII8
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| 4E6H | X-ray | 230 A | A | 18-661 | PDB |
| 4E85 | X-ray | 300 A | A/B | 18-661 | PDB |
| 4EBA | X-ray | 330 A | A/B/C/D/E/F | 18-661 | PDB |
| AF-Q6CII8-F1 | Predicted | AlphaFoldDB |
No variants for Q6CII8
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q6CII8 | |||||
No associated diseases with Q6CII8
8 regional properties for Q6CII8
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| repeat | HAT (Half-A-TPR) repeat | 62 - 94 | IPR003107-1 |
| repeat | HAT (Half-A-TPR) repeat | 99 - 133 | IPR003107-2 |
| repeat | HAT (Half-A-TPR) repeat | 147 - 179 | IPR003107-3 |
| repeat | HAT (Half-A-TPR) repeat | 190 - 223 | IPR003107-4 |
| repeat | HAT (Half-A-TPR) repeat | 256 - 296 | IPR003107-5 |
| repeat | HAT (Half-A-TPR) repeat | 466 - 498 | IPR003107-6 |
| repeat | HAT (Half-A-TPR) repeat | 500 - 535 | IPR003107-7 |
| domain | Suppressor of forked | 416 - 591 | IPR008847 |
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytosol | The part of the cytoplasm that does not contain organelles but which does contain other particulate matter, such as protein complexes. |
| mitochondrion | A semiautonomous, self replicating organelle that occurs in varying numbers, shapes, and sizes in the cytoplasm of virtually all eukaryotic cells. It is notably the site of tissue respiration. |
| mRNA cleavage factor complex | Any macromolecular complex involved in cleavage or polyadenylation of mRNA molecules. |
1 GO annotations of molecular function
| Name | Definition |
|---|---|
| RNA binding | Binding to an RNA molecule or a portion thereof. |
3 GO annotations of biological process
| Name | Definition |
|---|---|
| mRNA polyadenylation | The enzymatic addition of a sequence of 40-200 adenylyl residues at the 3' end of a eukaryotic mRNA primary transcript. |
| pre-mRNA cleavage required for polyadenylation | The targeted, endonucleolytic cleavage of a pre-mRNA, required for polyadenylation of the 3' end. This cleavage is directed by binding sites near the 3' end of the mRNA and leaves a 3' hydoxyl end which then becomes a target for adenylation. |
| response to DNA damage checkpoint signaling | A process that occurs in response to signals generated as a result of DNA damage checkpoint signaling. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSDGTATPDP | LPSSSNTSTS | LRPTSRVRDE | SDVIGKLNDM | IEEQPTDIFL | YVKLLKHHVS |
| 70 | 80 | 90 | 100 | 110 | 120 |
| LKQWKQVYET | FDKLHDRFPL | MANIWCMRLS | LEFDKMEELD | AAVIEPVLAR | CLSKELGNND |
| 130 | 140 | 150 | 160 | 170 | 180 |
| LSLWLSYITY | VRKKNDIITG | GEEARNIVIQ | AFQVVVDKCA | IFEPKSIQFW | NEYLHFLEHW |
| 190 | 200 | 210 | 220 | 230 | 240 |
| KPVNKFEEQQ | RVQYIRKLYK | TLLCQPMDCL | ESMWQRYTQW | EQDVNQLTAR | RHIGELSAQY |
| 250 | 260 | 270 | 280 | 290 | 300 |
| MNARSLYQDW | LNITKGLKRN | LPITLNQATE | SNLPKPNEYD | VQQLLIWLEW | IRWESDNKLE |
| 310 | 320 | 330 | 340 | 350 | 360 |
| LSDDLHKARM | TYVYMQAAQH | VCFAPEIWFN | MANYQGEKNT | DSTVITKYLK | LGQQCIPNSA |
| 370 | 380 | 390 | 400 | 410 | 420 |
| VLAFSLSEQY | ELNTKIPEIE | TTILSCIDRI | HLDLAALMED | DPTNESAINQ | LKSKLTYVYC |
| 430 | 440 | 450 | 460 | 470 | 480 |
| VYMNTMKRIQ | GLAASRKIFG | KCRRLKKLVT | PDIYLENAYI | EYHISKDTKT | ACKVLELGLK |
| 490 | 500 | 510 | 520 | 530 | 540 |
| YFATDGEYIN | KYLDFLIYVN | EESQVKSLFE | SSIDKISDSH | LLKMIFQKVI | FFESKVGSLN |
| 550 | 560 | 570 | 580 | 590 | 600 |
| SVRTLEKRFF | EKFPEVNKLE | EFTNKYKVLD | VNYLQRLELD | YMVRDVMPEA | IALDRGSNNL |
| 610 | 620 | 630 | 640 | 650 | 660 |
| KRTMREEEDG | QAFKKFKANE | DPIPPEIVEL | LKVLPKRQYF | KVTIFEAHAF | SEFLSDKVTI |
| Q |