Q5REG1
Gene name |
SART3 |
Protein name |
Squamous cell carcinoma antigen recognized by T-cells 3 |
Names |
SART-3 |
Species |
Pongo abelii (Sumatran orangutan) (Pongo pygmaeus abelii) |
KEGG Pathway |
pon:100171719 |
EC number |
|
Protein Class |
|
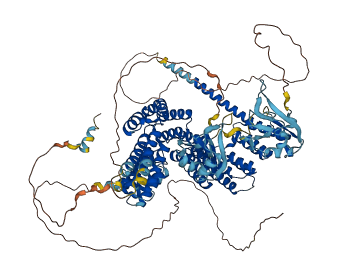
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q5REG1
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q5REG1-F1 | Predicted | AlphaFoldDB |
No variants for Q5REG1
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q5REG1 | |||||
No associated diseases with Q5REG1
12 regional properties for Q5REG1
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | RNA recognition motif domain | 722 - 800 | IPR000504-1 |
| domain | RNA recognition motif domain | 819 - 896 | IPR000504-2 |
| repeat | HAT (Half-A-TPR) repeat | 126 - 158 | IPR003107-1 |
| repeat | HAT (Half-A-TPR) repeat | 164 - 195 | IPR003107-2 |
| repeat | HAT (Half-A-TPR) repeat | 201 - 237 | IPR003107-3 |
| repeat | HAT (Half-A-TPR) repeat | 342 - 374 | IPR003107-4 |
| repeat | HAT (Half-A-TPR) repeat | 377 - 409 | IPR003107-5 |
| repeat | HAT (Half-A-TPR) repeat | 412 - 448 | IPR003107-6 |
| repeat | HAT (Half-A-TPR) repeat | 505 - 538 | IPR003107-7 |
| domain | LSM-interacting domain | 962 - 980 | IPR008669 |
| domain | SART3, RNA recognition motif 1 | 723 - 796 | IPR034217 |
| domain | SART3, RNA recognition motif 2 | 817 - 897 | IPR034218 |
5 GO annotations of cellular component
| Name | Definition |
|---|---|
| Cajal body | A class of nuclear body, first seen after silver staining by Ramon y Cajal in 1903, enriched in small nuclear ribonucleoproteins, and certain general RNA polymerase II transcription factors; ultrastructurally, they appear as a tangle of coiled, electron-dense threads roughly 0.5 micrometers in diameter; involved in aspects of snRNP biogenesis; the protein coilin serves as a marker for Cajal bodies. Some argue that Cajal bodies are the sites for preassembly of transcriptosomes, unitary particles involved in transcription and processing of RNA. |
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
| nuclear speck | A discrete extra-nucleolar subnuclear domain, 20-50 in number, in which splicing factors are seen to be localized by immunofluorescence microscopy. |
| nucleoplasm | That part of the nuclear content other than the chromosomes or the nucleolus. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
3 GO annotations of molecular function
| Name | Definition |
|---|---|
| histone binding | Binding to a histone, any of a group of water-soluble proteins found in association with the DNA of eukaryotic or archaeal chromosomes. They are involved in the condensation and coiling of chromosomes during cell division and have also been implicated in gene regulation and DNA replication. They may be chemically modified (methylated, acetlyated and others) to regulate gene transcription. |
| U6 snRNA binding | Binding to a U6 small nuclear RNA (U6 snRNA). |
| U6atac snRNA binding | Binding to a U6atac small nuclear RNA (U6atac snRNA). |
5 GO annotations of biological process
| Name | Definition |
|---|---|
| mRNA splicing, via spliceosome | The joining together of exons from one or more primary transcripts of messenger RNA (mRNA) and the excision of intron sequences, via a spliceosomal mechanism, so that mRNA consisting only of the joined exons is produced. |
| nucleosome assembly | The aggregation, arrangement and bonding together of a nucleosome, the beadlike structural units of eukaryotic chromatin composed of histones and DNA. |
| positive regulation of histone deubiquitination | Any process that activates or increases the frequency, rate or extent of histone deubiquitination. |
| spliceosomal snRNP assembly | The aggregation, arrangement and bonding together of one or more snRNA and multiple protein components to form a ribonucleoprotein complex that is involved in formation of the spliceosome. |
| spliceosomal tri-snRNP complex assembly | The formation of a tri-snRNP complex containing U4 and U6 (or U4atac and U6atac) snRNAs and U5 snRNAs and associated proteins. This includes reannealing of U4 and U6 (or U4atac and U6atac) snRNAs released from previous rounds of splicing to reform the U4/U6 snRNP (or U4atac/U6atac snRNP) as well as the subsequent association of the U5 snRNP with the U4/U6 snRNP (or U4atac/U6atac snRNP) to form a tri-snRNP that is ready to reassemble into another spliceosome complex. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MATAAATSAS | EPEAESKAGP | KADGEEDEVK | AARTRRKVLS | RAVAAATYKT | MGPGWDQQEE |
| 70 | 80 | 90 | 100 | 110 | 120 |
| GVSESDGDEY | AMASSAESSP | GEYEWEYDEE | EEKNQLEIER | LEEQLSINVY | DYNCHVDLIR |
| 130 | 140 | 150 | 160 | 170 | 180 |
| LLRLEGELTK | VRMARQKMSE | IFPLTEELWL | EWLHDEISMA | QDGLDREHVY | DLFEKAVKDY |
| 190 | 200 | 210 | 220 | 230 | 240 |
| ICPNIWLEYG | QYSVGGIGQK | GGLEKVRSVF | ERALSSVGLH | MTKGLALWEA | YREFESAIVE |
| 250 | 260 | 270 | 280 | 290 | 300 |
| AARPVAGFLS | PFDREQTFDS | QLEKVHSLFR | RQLAIPLYDM | EATFAEYEEW | SEDPIPESVI |
| 310 | 320 | 330 | 340 | 350 | 360 |
| QNYNKALQQL | EKYKPYEEAL | LQAEAPRLAE | YQAYIDFEMK | IGDPARIQLI | FERALVENCL |
| 370 | 380 | 390 | 400 | 410 | 420 |
| VPDLWIRYSQ | YLDRQLKVKD | LVLSVHNRAI | RNCPWTVALW | SRYLLAMERH | GVDHQVISVT |
| 430 | 440 | 450 | 460 | 470 | 480 |
| FEKALNAGFI | QATDYVEIWQ | AYLDYLRRRV | DFKQDSSKEL | EELRAAFTRA | LEYLKQEVEE |
| 490 | 500 | 510 | 520 | 530 | 540 |
| RFNESGDPSC | VIMQNWARIE | ARLCNNMQKA | RELWDSIMTR | GNAKYANMWL | EYYNLERAHG |
| 550 | 560 | 570 | 580 | 590 | 600 |
| DTQHCRKALH | RAVQCTSDYP | EHVCEVLLTM | ERTEGSLEDW | DIAVQKTETR | LARVNEQRMK |
| 610 | 620 | 630 | 640 | 650 | 660 |
| AAEKEAALVQ | QEEEKAEQRK | RARAEKKALK | KKKKIRGPEK | RGADEDDEKE | WGDDEEEQPS |
| 670 | 680 | 690 | 700 | 710 | 720 |
| KRRRVENSIP | AAGETQNVEV | APGPAGKCAA | VDVEPPSKQK | EKAASLKRDM | PKVLHDSSKD |
| 730 | 740 | 750 | 760 | 770 | 780 |
| SITVFVSNLP | YSMQEPDAKL | RPLFEACGEV | VQIRPIFSNR | GDFRGYRYVE | FKEEKSALQA |
| 790 | 800 | 810 | 820 | 830 | 840 |
| LEMDRKSVEG | RPMFVSPCVD | KSKNPDFKVF | RYSTSLEKHK | LFISGLPFSC | TKEELEEICK |
| 850 | 860 | 870 | 880 | 890 | 900 |
| AHGTVKDLRL | VTNRAGKPKG | LAYVEYENES | QASQAVMKMD | GMTIKENVIK | VAISNPPQRK |
| 910 | 920 | 930 | 940 | 950 | 960 |
| VPEKPETRKA | PGGPTLLPQT | YGARGKGRTQ | LSLLPRALQR | PGAAAPQAEN | GPAAAPAVAA |
| 970 | 980 | ||||
| PAATEAPKMS | NADFAKLFLR | K |