Q5RBC3
Gene name |
EXT1 |
Protein name |
Exostosin-1 |
Names |
Glucuronosyl-N-acetylglucosaminyl-proteoglycan/N-acetylglucosaminyl-proteoglycan 4-alpha-N-acetylglucosaminyltransferase, Multiple exostoses protein 1 homolog |
Species |
Pongo abelii (Sumatran orangutan) (Pongo pygmaeus abelii) |
KEGG Pathway |
pon:100172450 |
EC number |
2.4.1.225: Hexosyltransferases |
Protein Class |
|
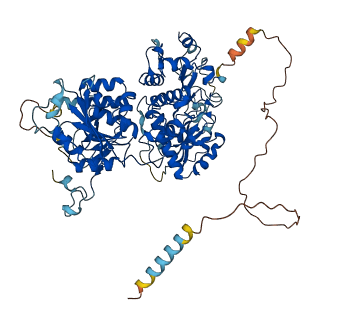
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q5RBC3
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q5RBC3-F1 | Predicted | AlphaFoldDB |
No variants for Q5RBC3
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q5RBC3 | |||||
No associated diseases with Q5RBC3
1 regional properties for Q5RBC3
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Enkurin domain | 243 - 343 | IPR027012 |
Functions
| Description | ||
|---|---|---|
| EC Number | 2.4.1.225 | Hexosyltransferases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| endoplasmic reticulum membrane | The lipid bilayer surrounding the endoplasmic reticulum. |
| Golgi membrane | The lipid bilayer surrounding any of the compartments of the Golgi apparatus. |
| integral component of membrane | The component of a membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
3 GO annotations of molecular function
| Name | Definition |
|---|---|
| glucuronosyl-N-acetylglucosaminyl-proteoglycan 4-alpha-N-acetylglucosaminyltransferase activity | Catalysis of the reaction: beta-D-glucuronosyl-(1,4)-N-acetyl-alpha-D-glucosaminyl-proteoglycan + UDP-N-acetyl-D-glucosamine = N-acetyl-alpha-D-glucosaminyl-(1,4)-beta-D-glucuronosyl-(1,4)-N-acetyl-alpha-D-glucosaminyl-proteoglycan + UDP. |
| metal ion binding | Binding to a metal ion. |
| N-acetylglucosaminyl-proteoglycan 4-beta-glucuronosyltransferase activity | Catalysis of the reaction: N-acetyl-alpha-D-glucosaminyl-(1,4)-beta-D-glucuronosyl-proteoglycan + UDP-alpha-D-glucuronate = beta-D-glucuronosyl-(1,4)-N-acetyl-alpha-D-glucosaminyl-(1,4)-beta-D-glucuronosyl-proteoglycan + UDP. |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| heparan sulfate proteoglycan biosynthetic process | The chemical reactions and pathways resulting in the formation of the heparan sulfate proteoglycan, a glycosaminoglycan with repeat unit consisting of alternating alpha-(1->4)-linked hexuronic acid and glucosamine residues; the former are a mixture of sulfated and nonsulfated D-glucuronic acid and L-iduronic acid; the L-iduronic acid is either sulfated or acetylated on its amino group as well as being sulfated on one of its hydroxyl groups; heparan sulfate chains are covalently linked to peptidyl-serine by a glycosidic attachment through the trisaccharide galactosyl-galactosyl-xylosyl to serine residues. |
| protein glycosylation | A protein modification process that results in the addition of a carbohydrate or carbohydrate derivative unit to a protein amino acid, e.g. the addition of glycan chains to proteins. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MQAKKRYFIL | LSAGSCLALL | FYFGGLQFRA | SRSHSRREEH | SGRNGLHHPS | PDHFWPRFPD |
| 70 | 80 | 90 | 100 | 110 | 120 |
| ALRPFVPWDQ | LENEDSSVHI | SPRQKRDANS | SIYKGKKCRM | ESCFDFTLCK | KNGFKVYAYP |
| 130 | 140 | 150 | 160 | 170 | 180 |
| QQKGEKIAES | YQNILAAIEG | SRFYTSDPSQ | ACLFVLSLDT | LDRDQLSPQY | VHNLRSKVQS |
| 190 | 200 | 210 | 220 | 230 | 240 |
| LHLWNNGRNH | LIFNLYSGTW | PDYTEDVGFD | IGQAMLAKAS | ISTENFRPNF | DVSIPLFSKD |
| 250 | 260 | 270 | 280 | 290 | 300 |
| HPRTGGERGF | LKFNTIPPLR | KYMLVFKGKR | YLTGIGSDTR | NALYHVHNGE | DVVLLTTCKH |
| 310 | 320 | 330 | 340 | 350 | 360 |
| GKDWQKHKDS | RCDRDNTEYE | KYDYREMLHN | ATFCLVPRGR | RLGSFRFLEA | LQAACVPVML |
| 370 | 380 | 390 | 400 | 410 | 420 |
| SNGWELPFSE | VINWNQAAVI | GDERLLLQIP | STIRSIHQDK | ILALRQQTQF | LWEAYFSSVE |
| 430 | 440 | 450 | 460 | 470 | 480 |
| KIVLTTLEII | QDRIFKHISR | NSLIWNKHPG | GLFVLPQYSS | YLGDFPYYYA | NLGLKPPSKF |
| 490 | 500 | 510 | 520 | 530 | 540 |
| TAVIHAVTPL | VSQSQPVLKL | LVAAAKSQYC | AQIIVLWNCD | KPLPAKHRWP | ATAVPVIVIE |
| 550 | 560 | 570 | 580 | 590 | 600 |
| GESKVMSSRF | LPYDNIITDA | VLSLDEDTVL | STTEVDFAFT | VWRSFPERIV | GYPARSHFWD |
| 610 | 620 | 630 | 640 | 650 | 660 |
| NSKERWGYTS | KWTNDYSMVL | TGAAIYHKYY | HYLYSHYLPA | SLKNMVDQLA | NCEDILMNFL |
| 670 | 680 | 690 | 700 | 710 | 720 |
| VSAVTKLPPI | KVTQKEQYKE | TMMGQTSRAS | RWADPDHFAQ | RQSCMNTFAS | WFGYMPLIHS |
| 730 | 740 | ||||
| QMRLDPVLFK | DQVSILRKKY | RDIERL |