Q5R9W1
Gene name |
MARCHF6 (MARCH6) |
Protein name |
E3 ubiquitin-protein ligase MARCHF6 |
Names |
Membrane-associated RING finger protein 6, Membrane-associated RING-CH protein VI, MARCH-VI, RING-type E3 ubiquitin transferase MARCH6 |
Species |
Pongo abelii (Sumatran orangutan) (Pongo pygmaeus abelii) |
KEGG Pathway |
|
EC number |
2.3.2.27: Aminoacyltransferases |
Protein Class |
|
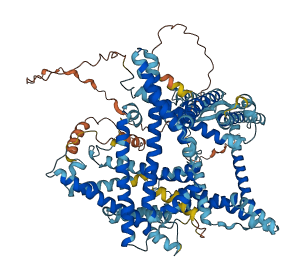
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q5R9W1
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q5R9W1-F1 | Predicted | AlphaFoldDB |
No variants for Q5R9W1
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q5R9W1 | |||||
No associated diseases with Q5R9W1
1 regional properties for Q5R9W1
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Zinc finger, RING-CH-type | 1 - 62 | IPR011016 |
Functions
| Description | ||
|---|---|---|
| EC Number | 2.3.2.27 | Aminoacyltransferases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| integral component of endoplasmic reticulum membrane | The component of the endoplasmic reticulum membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| ubiquitin protein ligase activity | Catalysis of the transfer of ubiquitin to a substrate protein via the reaction X-ubiquitin + S -> X + S-ubiquitin, where X is either an E2 or E3 enzyme, the X-ubiquitin linkage is a thioester bond, and the S-ubiquitin linkage is an amide bond: an isopeptide bond between the C-terminal glycine of ubiquitin and the epsilon-amino group of lysine residues in the substrate or, in the linear extension of ubiquitin chains, a peptide bond the between the C-terminal glycine and N-terminal methionine of ubiquitin residues. |
| zinc ion binding | Binding to a zinc ion (Zn). |
3 GO annotations of biological process
| Name | Definition |
|---|---|
| proteasome-mediated ubiquitin-dependent protein catabolic process | The chemical reactions and pathways resulting in the breakdown of a protein or peptide by hydrolysis of its peptide bonds, initiated by the covalent attachment of ubiquitin, and mediated by the proteasome. |
| protein K48-linked ubiquitination | A protein ubiquitination process in which a polymer of ubiquitin, formed by linkages between lysine residues at position 48 of the ubiquitin monomers, is added to a protein. K48-linked ubiquitination targets the substrate protein for degradation. |
| protein ubiquitination | The process in which one or more ubiquitin groups are added to a protein. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MDTAEEDICR | VCRSEGTPEK | PLYHPCVCTG | SIKFIHQECL | VQWLKHSRKE | YCELCKHRFA |
| 70 | 80 | 90 | 100 | 110 | 120 |
| FTPIYSPDMP | SRLPIQDIFA | GLVTSIGTAI | RYWFHYTLVA | FAWLGVVPLT | ACRIYKCLFT |
| 130 | 140 | 150 | 160 | 170 | 180 |
| GSVSSLLTLP | LDMLSTENLL | ADCLQGCFVV | TCTLCAFISL | VWLREQIVHG | GAPIWLEHAA |
| 190 | 200 | 210 | 220 | 230 | 240 |
| PPFNAAGHHQ | NEAPAGGNGA | ENVAADQPAN | PPAENAVVGE | NPDAQDDQAE | EEEEDNEEED |
| 250 | 260 | 270 | 280 | 290 | 300 |
| DAGVEDAADA | NNGAQDDMNW | NALEWDRAAE | ELTWERMLGL | DGSLVFLEHV | FWVVSLNTLF |
| 310 | 320 | 330 | 340 | 350 | 360 |
| ILVFAFCPYH | IGHFSLVGLG | FEEHVQASHF | EGLITTIVGY | ILLAITLIIC | HGLATLVKFH |
| 370 | 380 | 390 | 400 | 410 | 420 |
| RSRRLLGVCY | IVVKVSLLVV | VEIGVFPLIC | GWWLDICSLE | MFDATLKDRE | LSFQSAPGTT |
| 430 | 440 | 450 | 460 | 470 | 480 |
| MFLHWLVGMV | YVFYFASFIL | LLREVLRPGV | LWFLRNLNDP | DFNPVQEMIH | LPIYRHLRRF |
| 490 | 500 | 510 | 520 | 530 | 540 |
| ILSVIVFGSI | VLLMLWLPIR | IIKSVLPNFL | PYNVMLYSDA | PVSELSLELL | LLQVVLPALL |
| 550 | 560 | 570 | 580 | 590 | 600 |
| EQRTHEAVAE | GLVRAWTVTA | GYLLDLHSYL | LGDQEENENS | ANQQVNNNQH | ARNNNAIPVV |
| 610 | 620 | 630 | 640 | 650 | 660 |
| GEGLHAAHQA | ILQQGGPVGF | QPYRRPLNFP | LRIFLLIVFM | CITLLIASLI | CLTLPVFAGR |
| 670 | 680 | 690 | 700 | 710 | 720 |
| WLMSFWTGTA | KIHELYTAAC | GLYVCWLTIR | AVTVMVAWMP | QGRRVVFQKV | KEWSLMIMKT |
| 730 | 740 | 750 | 760 | 770 | 780 |
| LIVAVLLAGV | VPLLLGLLFE | LVIVAPLRVP | LDQTPLFYPW | QDWALGVLHA | KIIAAITLMG |
| 790 | 800 | 810 | 820 | 830 | 840 |
| PQWWLKTVIE | QVYANGIRNI | DLHYIVRKLA | APVISVLLLS | LCVPYVIASG | VVPLLGVTAE |
| 850 | 860 | 870 | 880 | 890 | 900 |
| MQNLVHRRIY | PFLLMVVVLM | AILSFQVRQF | KRLYEHIKND | KYLVGQRLVN | YERKSGKQGS |
| SPPPPQSSQE |