Q5B6U6
Gene name |
atg9 (AN3734) |
Protein name |
Autophagy-related protein 9 |
Names |
|
Species |
Emericella nidulans (strain FGSC A4 / ATCC 38163 / CBS 112.46 / NRRL 194 / M139) (Aspergillus nidulans) |
KEGG Pathway |
ani:AN3734.2 |
EC number |
|
Protein Class |
|
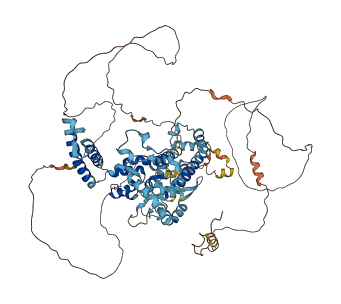
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q5B6U6
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q5B6U6-F1 | Predicted | AlphaFoldDB |
No variants for Q5B6U6
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q5B6U6 | |||||
No associated diseases with Q5B6U6
4 regional properties for Q5B6U6
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | ATPase, F1/V1/A1 complex, alpha/beta subunit, nucleotide-binding domain | 213 - 436 | IPR000194 |
| domain | ATPase, F1/V1/A1 complex, alpha/beta subunit, N-terminal domain | 6 - 68 | IPR004100 |
| active_site | ATPase, alpha/beta subunit, nucleotide-binding domain, active site | 427 - 436 | IPR020003 |
| domain | ATPsynthase alpha/beta subunit, N-terminal extension | 84 - 204 | IPR031686 |
Functions
7 GO annotations of cellular component
| Name | Definition |
|---|---|
| autophagosome | A double-membrane-bounded compartment that engulfs endogenous cellular material as well as invading microorganisms to target them to the lytic vacuole/lysosome for degradation as part of macroautophagy. |
| cytoplasmic vesicle membrane | The lipid bilayer surrounding a cytoplasmic vesicle. |
| endoplasmic reticulum membrane | The lipid bilayer surrounding the endoplasmic reticulum. |
| Golgi membrane | The lipid bilayer surrounding any of the compartments of the Golgi apparatus. |
| integral component of membrane | The component of a membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
| phagophore assembly site | Punctate structures proximal to the endoplasmic reticulum which are the sites where the Atg machinery assembles upon autophagy induction. |
| phagophore assembly site membrane | A cellular membrane associated with the phagophore assembly site. |
No GO annotations of molecular function
| Name | Definition |
|---|---|
| No GO annotations for molecular function |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| autophagy of mitochondrion | The autophagic process in which mitochondria are delivered to a type of vacuole and degraded in response to changing cellular conditions. |
| late nucleophagy | A type of nucleophagy, distinct from piecemeal microautophagy of the nucleus (PNM) where the nuclear material is delivered to the vacuole/lysosome for breakdown and recycling later than observed for PNM. |
| lipid transport | The directed movement of lipids into, out of or within a cell, or between cells, by means of some agent such as a transporter or pore. Lipids are compounds soluble in an organic solvent but not, or sparingly, in an aqueous solvent. |
| protein localization to phagophore assembly site | Any process in which a protein is transported to, or maintained at, the phagophore assembly site (PAS). |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MMASNVLSRL | LPQTGQSVYE | TIRQHDNDSD | ASDVEERAGL | VYDDDVNLGN | RFSDRELEEA |
| 70 | 80 | 90 | 100 | 110 | 120 |
| MADATREGSS | SPSDTFLTPQ | IAQRGERSAS | SGPRMRKPNN | PRFMRSVTPR | PEFVEDDLDD |
| 130 | 140 | 150 | 160 | 170 | 180 |
| DHDDDVPASL | LMEGQHDDEY | LRTRLPPPPS | HHFSDPQPSR | SARSPRREHI | RTFAFVVGFT |
| 190 | 200 | 210 | 220 | 230 | 240 |
| TFLTNCIDYR | LVRTSKSLDQ | ILISKCTSRM | SASSTFLLWL | LCLFWIGKIF | QLILDIRRLK |
| 250 | 260 | 270 | 280 | 290 | 300 |
| NMHDFYHYLL | GVSDAEIQTI | SWQEVVSRLM | TLRDANPATA | GAVSAFNRRL | LGSQSKQRMD |
| 310 | 320 | 330 | 340 | 350 | 360 |
| AHDIANRLMR | KENYLIALIN | KDILDLTLPI | PFLRNRQLFS | RILEWNINLC | IMDYVFNEQG |
| 370 | 380 | 390 | 400 | 410 | 420 |
| QLSSRQYTPL | AEWKFREFNE | LWHLFEKRIN | LSYPYATRYV | DQFPKDKTVQ | VAGFVAFISG |
| 430 | 440 | 450 | 460 | 470 | 480 |
| ALASVLALAS | ILDPELFLGF | ELTHDRTTLF | YLGVFGSVWA | FARGMVPEET | LVFDPEYALL |
| 490 | 500 | 510 | 520 | 530 | 540 |
| EVIQFTHYFP | SHWKGKLHSD | DVRREFAVLY | QMKIIIFMEE | ILSMIFTPFI | LWFSLPKCSE |
| 550 | 560 | 570 | 580 | 590 | 600 |
| RVIDFFREFT | VHVDGMGYLC | SFAVFDFKKG | TNVIPQGHIN | QRDARQDPRV | DYFSTKDGKM |
| 610 | 620 | 630 | 640 | 650 | 660 |
| LASYYGFLDN | YGGNPRATNA | NKRAFHPPPT | FPSLGSPPFV | GASNIGNRQD | PIQARVNTAS |
| 670 | 680 | 690 | 700 | 710 | 720 |
| AALGQQSMLG | ATRLGALGVG | DTQSPAPSLL | LDPQHQPSAS | GFRATNHIAP | HHRQRLGRPP |
| 730 | 740 | 750 | 760 | 770 | 780 |
| PAPVSESIID | DNEPSIAAAR | RPAPRRKSGQ | LHTNSGSSEA | LGAGDSNVED | SWGMKSGGEV |
| 790 | 800 | 810 | |||
| NDEDAEENVD | DVVGGAGVLG | LIQQFQKVNK | DNRPRAAVGL |