Q3SWZ7
Gene name |
WRAP53 |
Protein name |
Telomerase Cajal body protein 1 |
Names |
WD repeat-containing protein 79, WD40 repeat-containing protein antisense to TP53 gene homolog |
Species |
Bos taurus (Bovine) |
KEGG Pathway |
bta:509631 |
EC number |
|
Protein Class |
|
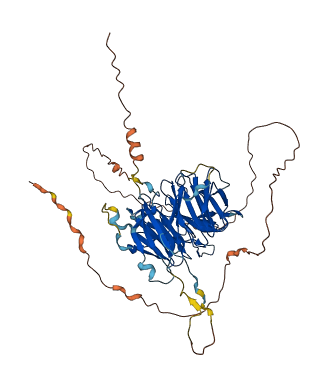
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q3SWZ7
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q3SWZ7-F1 | Predicted | AlphaFoldDB |
No variants for Q3SWZ7
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q3SWZ7 | |||||
No associated diseases with Q3SWZ7
6 regional properties for Q3SWZ7
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| repeat | WD40 repeat | 149 - 188 | IPR001680-1 |
| repeat | WD40 repeat | 252 - 295 | IPR001680-2 |
| repeat | WD40 repeat | 302 - 344 | IPR001680-3 |
| repeat | WD40 repeat | 347 - 387 | IPR001680-4 |
| repeat | WD40 repeat | 392 - 432 | IPR001680-5 |
| repeat | WD40 repeat | 441 - 477 | IPR001680-6 |
Functions
4 GO annotations of cellular component
| Name | Definition |
|---|---|
| Cajal body | A class of nuclear body, first seen after silver staining by Ramon y Cajal in 1903, enriched in small nuclear ribonucleoproteins, and certain general RNA polymerase II transcription factors; ultrastructurally, they appear as a tangle of coiled, electron-dense threads roughly 0.5 micrometers in diameter; involved in aspects of snRNP biogenesis; the protein coilin serves as a marker for Cajal bodies. Some argue that Cajal bodies are the sites for preassembly of transcriptosomes, unitary particles involved in transcription and processing of RNA. |
| chromosome, telomeric region | The end of a linear chromosome, required for the integrity and maintenance of the end. A chromosome telomere usually includes a region of telomerase-encoded repeats the length of which rarely exceeds 20 bp each and that permits the formation of a telomeric loop (T-loop). The telomeric repeat region is usually preceded by a sub-telomeric region that is gene-poor but rich in repetitive elements. Some telomeres only consist of the latter part (for eg. D. melanogaster telomeres). |
| site of double-strand break | A region of a chromosome at which a DNA double-strand break has occurred. DNA damage signaling and repair proteins accumulate at the lesion to respond to the damage and repair the DNA to form a continuous DNA helix. |
| telomerase holoenzyme complex | Telomerase is a ribonucleoprotein enzyme complex, with a minimal catalytic core composed of a catalytic reverse transcriptase subunit and an RNA subunit that provides the template for telomeric DNA addition. In vivo, the holoenzyme complex often contains additional subunits. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| RNA binding | Binding to an RNA molecule or a portion thereof. |
| telomerase RNA binding | Binding to the telomerase RNA template. |
12 GO annotations of biological process
| Name | Definition |
|---|---|
| Cajal body organization | A process that is carried out at the cellular level which results in the assembly, arrangement of constituent parts, or disassembly of Cajal bodies, nuclear bodies that appear ultrastructurally as a tangle of coiled, electron-dense threads roughly 0.5 micrometers in diameter and are enriched in ribonucleoproteins, and certain general RNA polymerase II transcription factors. |
| DNA repair | The process of restoring DNA after damage. Genomes are subject to damage by chemical and physical agents in the environment (e.g. UV and ionizing radiations, chemical mutagens, fungal and bacterial toxins, etc.) and by free radicals or alkylating agents endogenously generated in metabolism. DNA is also damaged because of errors during its replication. A variety of different DNA repair pathways have been reported that include direct reversal, base excision repair, nucleotide excision repair, photoreactivation, bypass, double-strand break repair pathway, and mismatch repair pathway. |
| positive regulation of DNA repair | Any process that activates or increases the frequency, rate or extent of DNA repair. |
| positive regulation of double-strand break repair | Any process that activates or increases the frequency, rate or extent of double-strand break repair. |
| positive regulation of double-strand break repair via homologous recombination | Any process that activates or increases the frequency, rate or extent of double-strand break repair via homologous recombination. |
| positive regulation of double-strand break repair via nonhomologous end joining | Any process that activates or increases the frequency, rate or extent of double-strand break repair via nonhomologous end joining. |
| positive regulation of telomerase activity | Any process that activates or increases the frequency, rate or extent of telomerase activity, the catalysis of the reaction: deoxynucleoside triphosphate + DNA(n) = diphosphate + DNA(n+1). |
| protein localization to Cajal body | A process in which a protein is transported to, or maintained in, a location within a Cajal body. |
| RNA folding | The process of assisting in the covalent and noncovalent assembly of single or multimeric RNAs into the correct tertiary structure. |
| scaRNA localization to Cajal body | A process in which a small Cajal body-specific RNA is transported to, or maintained in, a Cajal body. |
| telomere formation via telomerase | A cellular process that results in the formation of a telomere at a non-telomeric double-stranded DNA end that involves the activity of a telomerase enzyme. |
| telomere maintenance via telomerase | The maintenance of proper telomeric length by the addition of telomeric repeats by telomerase. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MKTPEAPPLA | PDCLPSDQAP | APARLSRQAS | PMDKNTDPEL | MPTPRDGDDP | PQVSSDPMVG |
| 70 | 80 | 90 | 100 | 110 | 120 |
| LALSQELEEG | VPASLPTPLE | SGFGSPSELS | SRVEEKELSE | NVSLPAEETN | RPELGPGEDV |
| 130 | 140 | 150 | 160 | 170 | 180 |
| EGVSEELTPE | DEGYTIWNYN | FSQVPRFLSG | SWSEFITQPE | NFLKGCKWAP | DGSCILTNSA |
| 190 | 200 | 210 | 220 | 230 | 240 |
| DNILRIYNLP | PELYNEGEQL | EYAEMAPVLR | MVEGDTIYDY | CWYSLMSSAQ | PDTSYVASSS |
| 250 | 260 | 270 | 280 | 290 | 300 |
| RENPIHIWDA | FTGELRASFR | SYNHLDELTA | AHSLCFSPDG | SQLFCGFNRT | VRVFSTSRPG |
| 310 | 320 | 330 | 340 | 350 | 360 |
| RDCEVRTTFA | KRQGQSGIIS | CIAFSPTQPL | YACGSYGRSL | GLYTWEDGSP | LALLGGHQGG |
| 370 | 380 | 390 | 400 | 410 | 420 |
| ITHLCFHPDG | NCFFSGARKD | AELLCWDLRQ | LGHPLWSLSR | EVTTNQRIYF | DLDPTGQFLV |
| 430 | 440 | 450 | 460 | 470 | 480 |
| SGSTSGAVSV | WDTGGAGLES | KPEPVLSFQP | QKDCTNGVSL | HPSLPLLATA | SGQRVFPEPT |
| 490 | 500 | 510 | 520 | 530 | |
| ESGDEREEEV | DLPLLSMRHV | HLECQLQLWW | CGGGPDTSIS | DAHQEEMGQG | RTEGGGGEFT |