Q3ANH2
Gene name |
secA |
Protein name |
Protein translocase subunit SecA |
Names |
|
Species |
Synechococcus sp (strain CC9605) |
KEGG Pathway |
syd:Syncc9605_0081 |
EC number |
7.4.2.8: Linked to the hydrolysis of a nucleoside triphosphate |
Protein Class |
|
Descriptions
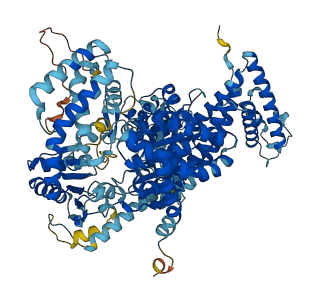
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q3ANH2
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q3ANH2-F1 | Predicted | AlphaFoldDB |
No variants for Q3ANH2
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q3ANH2 | |||||
No associated diseases with Q3ANH2
7 regional properties for Q3ANH2
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | SecA DEAD-like, N-terminal | 2 - 397 | IPR011115 |
| domain | SecA Wing/Scaffold | 714 - 927 | IPR011116 |
| domain | SecA, preprotein cross-linking domain | 231 - 353 | IPR011130 |
| domain | Helicase superfamily 1/2, ATP-binding domain | 92 - 230 | IPR014001 |
| domain | SecA motor DEAD | 1 - 716 | IPR014018 |
| conserved_site | SecA conserved site | 497 - 512 | IPR020937 |
| domain | SecA, C-terminal helicase domain | 415 - 686 | IPR044722 |
Functions
| Description | ||
|---|---|---|
| EC Number | 7.4.2.8 | Linked to the hydrolysis of a nucleoside triphosphate |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| plasma membrane-derived thylakoid membrane | The pigmented membrane of a plasma membrane-derived thylakoid. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| protein-exporting ATPase activity | Enables the transfer of a solute or solutes from one side of a membrane to the other according to the reaction: ATP + H2O + protein+(in) -> ADP + phosphate + protein+(out); drives the concomitant secretion of proteins. |
3 GO annotations of biological process
| Name | Definition |
|---|---|
| intracellular protein transmembrane transport | The directed movement of proteins in a cell, from one side of a membrane to another by means of some agent such as a transporter or pore. |
| protein import | The targeting and directed movement of proteins into a cell or organelle. Not all import involves an initial targeting event. |
| protein targeting | The process of targeting specific proteins to particular regions of the cell, typically membrane-bounded subcellular organelles. Usually requires an organelle specific protein sequence motif. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MLKLLLGDPN | ARKLKRYQPI | VSDIQLLEEE | IAPLSDDELR | GRTAAFQERL | ANAGSLANQR |
| 70 | 80 | 90 | 100 | 110 | 120 |
| PILDEILPEA | FAVVREAGKR | VLGMRHFDVQ | LIGGMVLHEG | QIAEMKTGEG | KTLVATLPSY |
| 130 | 140 | 150 | 160 | 170 | 180 |
| LNALTGRGVH | VVTVNDYLAR | RDAEWMGQVH | RFLGLSVGLI | QQDMRPEERR | RNYNCDITYA |
| 190 | 200 | 210 | 220 | 230 | 240 |
| TNSELGFDYL | RDNMAADISE | VVQREFQYCV | IDEVDSILID | EARTPLIISG | QVERPQEKYQ |
| 250 | 260 | 270 | 280 | 290 | 300 |
| QAAEVANALA | RAAELSKDGI | DPEGDYEVDE | KQRSCTLTDE | GFAKAEQMLG | VADLFNPQDP |
| 310 | 320 | 330 | 340 | 350 | 360 |
| WAHYITNALK | AKELFVKDVN | YIVRDGEAVI | VDEFTGRVMP | GRRWSDGQHQ | AIEAKEALAI |
| 370 | 380 | 390 | 400 | 410 | 420 |
| QSETQTLASI | TYQNFFLLYP | RLAGMTGTAK | TEEVEFEKTY | KLETTIVPTN | RVRARQDWAD |
| 430 | 440 | 450 | 460 | 470 | 480 |
| QVYKTEAAKW | RAVANETAEI | HKNGRPVLVG | TTSVEKSELL | SSLLAEQEIP | HNLLNAKPEN |
| 490 | 500 | 510 | 520 | 530 | 540 |
| VERESEIVAQ | AGRAGAVTIA | TNMAGRGTDI | ILGGNSDYMA | RLKLREVLLG | RLVKPEEDHT |
| 550 | 560 | 570 | 580 | 590 | 600 |
| PPVPLQRSAP | GGFSDAAAPS | LPRSGESLYP | CPLTDDTDQA | LGQLARDLVK | AWGDRALTVI |
| 610 | 620 | 630 | 640 | 650 | 660 |
| ELEERIATAA | EKAPTEAPQI | QALREAIARV | KGEYDAVVKQ | EESRVREAGG | LHVIGTERHE |
| 670 | 680 | 690 | 700 | 710 | 720 |
| SRRVDNQLRG | RAGRQGDPGS | TRFFLSLGDN | LLRIFGGDRV | AGLMNAFRVE | EDMPIESGML |
| 730 | 740 | 750 | 760 | 770 | 780 |
| TRSLEGAQKK | VETYYYDIRK | QVFEYDEVMN | NQRRAVYSER | RRVLDGRALK | KQVIGYGERT |
| 790 | 800 | 810 | 820 | 830 | 840 |
| MGEIVEAYVN | PDLPPEEWDL | DQLVGKVKEF | IYLLEDLTPD | QVQGLGMEEL | KAFLQEQLRN |
| 850 | 860 | 870 | 880 | 890 | 900 |
| AYDLKEGQIE | QQRPGLMREA | ERFFILQQID | TLWREHLQAM | DALRESVGLR | GYGQKDPLIE |
| 910 | 920 | 930 | |||
| YKNEGYDMFL | EMMTNMRRNV | IYSMFMFQPQ | APKN |