Q2U002
Gene name |
tif35 (AO090011000648) |
Protein name |
Eukaryotic translation initiation factor 3 subunit G |
Names |
eIF3g, Eukaryotic translation initiation factor 3 RNA-binding subunit, eIF-3 RNA-binding subunit, Translation initiation factor eIF3 p33 subunit homolog, eIF3 p33 homolog |
Species |
Aspergillus oryzae (strain ATCC 42149 / RIB 40) (Yellow koji mold) |
KEGG Pathway |
aor:AO090011000648 |
EC number |
|
Protein Class |
|
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
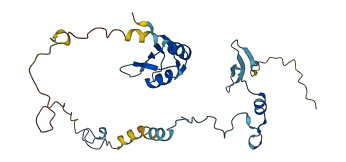
Autoinhibited structure

Activated structure
1 structures for Q2U002
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q2U002-F1 | Predicted | AlphaFoldDB |
No variants for Q2U002
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q2U002 | |||||
No associated diseases with Q2U002
5 GO annotations of cellular component
| Name | Definition |
|---|---|
| eukaryotic 43S preinitiation complex | A protein complex composed of the 40S ribosomal subunit plus eIF1A, eIF3, and eIF2-GTP-bound methionyl-initiator methionine tRNA. |
| eukaryotic 48S preinitiation complex | A protein complex composed of the small ribosomal subunit, eIF3, eIF1A, methionyl-initiatior methionine and a capped mRNA. The complex is initially positioned at the 5'-end of the capped mRNA. |
| eukaryotic translation initiation factor 3 complex, eIF3e | An eukaryotic translation initiation factor 3 complex that contains the PCI-domain protein eIF3e. |
| eukaryotic translation initiation factor 3 complex, eIF3m | An eukaryotic translation initiation factor 3 complex that contains the PCI-domain protein eIF3m. |
| multi-eIF complex | A multifactor complex composed of multiple translation initiation factors and the initiatior tRNAiMet, which is ready to bind to the small (40S) ribosome to form the 43S preinitiation complex. In S. cerevisiae, this complex is composed of eIF1, eIF2, eIF3, and eIF5. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| RNA binding | Binding to an RNA molecule or a portion thereof. |
| translation initiation factor activity | Functions in the initiation of ribosome-mediated translation of mRNA into a polypeptide. |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| formation of cytoplasmic translation initiation complex | Joining of the large subunit, with release of IF2/eIF2 and IF3/eIF3. This leaves the functional ribosome at the AUG, with the methionyl/formyl-methionyl-tRNA positioned at the P site. |
| positive regulation of ATP-dependent activity | Any process that activates or increases the rate of an ATP-dependent activity. |
| translation reinitiation | A gene-specific translational control mechanism where the small ribosomal subunit remains attached to the mRNA following termination of translation, then resumes scanning on the same mRNA molecule and initiates again at a downstream start site. Reinitiation depends on de novo recruitment of the ternary complex that is required to recognize the next AUG codon. |
| translational termination | The process resulting in the release of a polypeptide chain from the ribosome, usually in response to a termination codon (UAA, UAG, or UGA in the universal genetic code). |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSKLANRADW | ADDEEFDDPS | ALPAQQVTTN | KDGTKTVVSY | RFNDEGKKVK | VTRRIKTTVV |
| 70 | 80 | 90 | 100 | 110 | 120 |
| REHVNPQVAE | RRSWAKFGLE | KGHAPGPSFD | TTSVGENIAF | RPSINWKAQA | AEAEKNGGEK |
| 130 | 140 | 150 | 160 | 170 | 180 |
| GSMKDQLKDK | KVKCRICSGE | HFTARCPFKD | TMAPVDEPTA | GGAGEDDEAA | AGAVGTGSGS |
| 190 | 200 | 210 | 220 | 230 | 240 |
| YVPPHLRKGA | AGGGERMGGK | FEKDDLATLR | VTNVSELAEE | GELRDLFERF | GRVTRVFLAR |
| 250 | 260 | 270 | 280 | ||
| DRETQRAKGF | AFISFADRSD | AARACEKMDG | FGYRHLILRV | EFAKRTT |