Q2FYS5
Gene name |
parE |
Protein name |
DNA topoisomerase 4 subunit B |
Names |
Topoisomerase IV subunit B |
Species |
Staphylococcus aureus (strain NCTC 8325 / PS 47) |
KEGG Pathway |
sao:SAOUHSC_01351 |
EC number |
5.6.2.2: Enzymes altering nucleic acid conformation |
Protein Class |
|
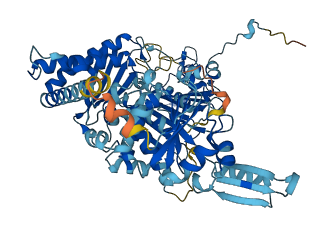
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q2FYS5
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q2FYS5-F1 | Predicted | AlphaFoldDB |
No variants for Q2FYS5
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q2FYS5 | |||||
No associated diseases with Q2FYS5
5 regional properties for Q2FYS5
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | DNA gyrase B subunit, C-terminal | 570 - 631 | IPR002288 |
| domain | Histidine kinase/HSP90-like ATPase | 32 - 176 | IPR003594 |
| domain | TOPRIM domain | 424 - 538 | IPR006171 |
| domain | DNA topoisomerase, type IIA, subunit B, domain 2 | 224 - 394 | IPR013506 |
| conserved_site | DNA topoisomerase, type IIA, conserved site | 428 - 436 | IPR018522 |
Functions
| Description | ||
|---|---|---|
| EC Number | 5.6.2.2 | Enzymes altering nucleic acid conformation |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| chromosome | A structure composed of a very long molecule of DNA and associated proteins (e.g. histones) that carries hereditary information. |
4 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| DNA binding | Any molecular function by which a gene product interacts selectively and non-covalently with DNA (deoxyribonucleic acid). |
| DNA topoisomerase type II (double strand cut, ATP-hydrolyzing) activity | Catalysis of a DNA topological transformation by transiently cleaving a pair of complementary DNA strands to form a gate through which a second double-stranded DNA segment is passed, after which the severed strands in the first DNA segment are rejoined, driven by ATP hydrolysis. The enzyme changes the linking number in multiples of 2. |
| metal ion binding | Binding to a metal ion. |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| chromosome segregation | The process in which genetic material, in the form of chromosomes, is organized into specific structures and then physically separated and apportioned to two or more sets. In eukaryotes, chromosome segregation begins with the condensation of chromosomes, includes chromosome separation, and ends when chromosomes have completed movement to the spindle poles. |
| DNA topological change | The process in which a transformation is induced in the topological structure of a double-stranded DNA helix, resulting in a change in linking number. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MNKQNNYSDD | SIQVLEGLEA | VRKRPGMYIG | STDKRGLHHL | VYEIVDNSVD | EVLNGYGNEI |
| 70 | 80 | 90 | 100 | 110 | 120 |
| DVTINKDGSI | SIEDNGRGMP | TGIHKSGKPT | VEVIFTVLHA | GGKFGQGGYK | TSGGLHGVGA |
| 130 | 140 | 150 | 160 | 170 | 180 |
| SVVNALSEWL | EVEIHRDGNI | YHQSFKNGGS | PSSGLVKKGK | TKKTGTKVTF | KPDDTIFKAS |
| 190 | 200 | 210 | 220 | 230 | 240 |
| TSFNFDVLSE | RLQESAFLLK | NLKITLNDLR | SGKERQEHYH | YEEGIKEFVS | YVNEGKEVLH |
| 250 | 260 | 270 | 280 | 290 | 300 |
| DVATFSGEAN | GIEVDVAFQY | NDQYSESILS | FVNNVRTKDG | GTHEVGFKTA | MTRVFNDYAR |
| 310 | 320 | 330 | 340 | 350 | 360 |
| RINELKTKDK | NLDGNDIREG | LTAVVSVRIP | EELLQFEGQT | KSKLGTSEAR | SAVDSVVADK |
| 370 | 380 | 390 | 400 | 410 | 420 |
| LPFYLEEKGQ | LSKSLVKKAI | KAQQAREAAR | KAREDARSGK | KNKRKDTLLS | GKLTPAQSKN |
| 430 | 440 | 450 | 460 | 470 | 480 |
| TEKNELYLVE | GDSAGGSAKL | GRDRKFQAIL | PLRGKVINTE | KARLEDIFKN | EEINTIIHTI |
| 490 | 500 | 510 | 520 | 530 | 540 |
| GAGVGTDFKI | EDSNYNRVII | MTDADTDGAH | IQVLLLTFFF | KYMKPLVQAG | RVFIALPPLY |
| 550 | 560 | 570 | 580 | 590 | 600 |
| KLEKGKGKTK | RVEYAWTDEE | LNKLQKELGK | GFTLQRYKGL | GEMNPEQLWE | TTMNPETRTL |
| 610 | 620 | 630 | 640 | 650 | 660 |
| IRVQVEDEVR | SSKRVTTLMG | DKVQPRREWI | EKHVEFGMQE | DQSILDNSEV | QVLENDQFDE |
| EEI |