Q24TH1
Gene name |
ileS |
Protein name |
Isoleucine--tRNA ligase |
Names |
Isoleucyl-tRNA synthetase, IleRS |
Species |
Desulfitobacterium hafniense (strain Y51) |
KEGG Pathway |
dsy:DSY2882 |
EC number |
6.1.1.5: Ligases forming aminoacyl-tRNA and related compounds |
Protein Class |
|
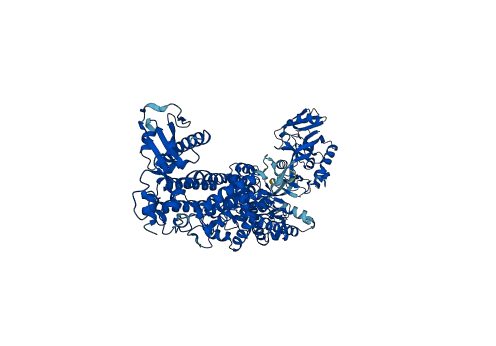
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q24TH1
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q24TH1-F1 | Predicted | AlphaFoldDB |
No variants for Q24TH1
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q24TH1 | |||||
No associated diseases with Q24TH1
5 regional properties for Q24TH1
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| conserved_site | Aminoacyl-tRNA synthetase, class I, conserved site | 57 - 68 | IPR001412 |
| domain | Aminoacyl-tRNA synthetase, class Ia | 27 - 632 | IPR002300 |
| domain | Zinc finger, FPG/IleRS-type | 889 - 918 | IPR010663 |
| domain | Methionyl/Valyl/Leucyl/Isoleucyl-tRNA synthetase, anticodon-binding | 677 - 831 | IPR013155 |
| domain | Isoleucyl tRNA synthetase type 1, anticodon-binding domain | 632 - 811 | IPR033708 |
Functions
| Description | ||
|---|---|---|
| EC Number | 6.1.1.5 | Ligases forming aminoacyl-tRNA and related compounds |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| aminoacyl-tRNA editing activity | The hydrolysis of an incorrectly aminoacylated tRNA. |
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| isoleucine-tRNA ligase activity | Catalysis of the reaction: L-isoleucine + ATP + tRNA(Ile) = L-isoleucyl-tRNA(Ile) + AMP + diphosphate + 2 H(+). |
| tRNA binding | Binding to a transfer RNA. |
| zinc ion binding | Binding to a zinc ion (Zn). |
1 GO annotations of biological process
| Name | Definition |
|---|---|
| isoleucyl-tRNA aminoacylation | The process of coupling isoleucine to isoleucyl-tRNA, catalyzed by isoleucyl-tRNA synthetase. The isoleucyl-tRNA synthetase is a class-I synthetase. The activated amino acid is transferred to the 2'-OH group of a isoleucine-accetping tRNA. The 2'-O-aminoacyl-tRNA will ultimately migrate to the 3' position via transesterification. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MDYRNTLNLP | ETDFPMRGNL | PQREPEILQK | WEEEDIYATV | QKARAGRPKF | VLHDGPPYAN |
| 70 | 80 | 90 | 100 | 110 | 120 |
| GDIHLGHALN | KVIKDIIVKY | KTMAGFDAPY | VPGWDTHGLP | IEQQVIKKLG | VNRHAVSVVE |
| 130 | 140 | 150 | 160 | 170 | 180 |
| FRRMCKEYAK | KYISIQKEQF | KRLGVRGDWK | NPYLTLEKEY | EAAQIGVFGK | MARKKYIYKG |
| 190 | 200 | 210 | 220 | 230 | 240 |
| LKPVYWCPSC | ETALAEAEIE | YAEKTSHAIY | VKFPVKEGKG | VLTDENTFVI | IWTTTPWTLP |
| 250 | 260 | 270 | 280 | 290 | 300 |
| ANLAITLHEE | FSYVQVQVEK | EHWLVAEGML | ESLRSLWNLE | LPVEKRFVGK | ELEGVICKHP |
| 310 | 320 | 330 | 340 | 350 | 360 |
| FIERDSVLIL | GEHVTLEAGT | GCVHTAPGHG | EEDFNVGKKY | GLPVLCPVDH | QGKFTAEGGA |
| 370 | 380 | 390 | 400 | 410 | 420 |
| YAGMKVDKAN | PVIIEDLKNL | HALVHEDKIK | HSYAHCWRCN | NPIIYRATEQ | WFASIDGFRK |
| 430 | 440 | 450 | 460 | 470 | 480 |
| AALEEIDKVQ | WIPSWGKDRI | YNMIADRGDW | CISRQRTWGV | PIPIFYCEDC | GKEIISDETI |
| 490 | 500 | 510 | 520 | 530 | 540 |
| AKVQEIFREE | GSDAWFLRPA | AELLPEGFTC | ACGGKSFRKE | TDIMDVWFDS | GTSHTSVLME |
| 550 | 560 | 570 | 580 | 590 | 600 |
| RKELAWPADL | YMEGSDQHRG | WFNSSLSTSV | AAYGKAPYKA | VLTHGFLVDE | KGRKMSKSLG |
| 610 | 620 | 630 | 640 | 650 | 660 |
| NGVDPLQVTK | EMGADILRLW | VCAADYKNDV | AVSPRIMKQM | SEAYRKIRNT | LRFLLSNLND |
| 670 | 680 | 690 | 700 | 710 | 720 |
| FDPAKDRVAY | KDLPEIDRWA | LLQLGKVTQR | VLQGYEKYEF | HWVYHSVHNF | CAVELSAIYL |
| 730 | 740 | 750 | 760 | 770 | 780 |
| DIVKDRLYVE | GKNSTLRRAS | QTVLYDVLNA | LVRLMAPVLT | YTADEIWPYV | PGVPAGSHVQ |
| 790 | 800 | 810 | 820 | 830 | 840 |
| TEEMPEALPQ | WLDEALEKKW | DTLLAVRSEV | TKALEKARQD | KLINHPLTAQ | VDLYPNAELE |
| 850 | 860 | 870 | 880 | 890 | 900 |
| GFLRGIPNLS | EIFIVSAVQL | HSAGEEKPEG | LSMAEDLAGF | GIAVNSAAGE | KCERCWIYDT |
| 910 | 920 | ||||
| GVGENQEHPT | LCPRCASVVS | HL |