Q1JHM2
Gene name |
rexB |
Protein name |
ATP-dependent helicase/deoxyribonuclease subunit B |
Names |
ATP-dependent helicase/nuclease RexB |
Species |
Streptococcus pyogenes serotype M2 (strain MGAS10270) |
KEGG Pathway |
sph:MGAS10270_Spy0649 |
EC number |
|
Protein Class |
|
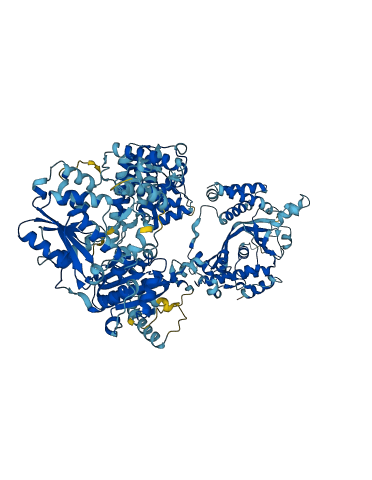
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q1JHM2
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q1JHM2-F1 | Predicted | AlphaFoldDB |
No variants for Q1JHM2
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q1JHM2 | |||||
No associated diseases with Q1JHM2
1 regional properties for Q1JHM2
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | PD-(D/E)XK endonuclease-like domain, AddAB-type | 743 - 1020 | IPR038726 |
No GO annotations of cellular component
| Name | Definition |
|---|---|
| No GO annotations for cellular component |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| 5'-3' exonuclease activity | Catalysis of the hydrolysis of ester linkages within nucleic acids by removing nucleotide residues from the 5' end. |
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP hydrolysis activity | Catalysis of the reaction: ATP + H2O = ADP + H+ phosphate. ATP hydrolysis is used in some reactions as an energy source, for example to catalyze a reaction or drive transport against a concentration gradient. |
| DNA helicase activity | Unwinding of a DNA helix, driven by ATP hydrolysis. |
| double-stranded DNA binding | Binding to double-stranded DNA. |
1 GO annotations of biological process
| Name | Definition |
|---|---|
| double-strand break repair via homologous recombination | The error-free repair of a double-strand break in DNA in which the broken DNA molecule is repaired using homologous sequences. A strand in the broken DNA searches for a homologous region in an intact chromosome to serve as the template for DNA synthesis. The restoration of two intact DNA molecules results in the exchange, reciprocal or nonreciprocal, of genetic material between the intact DNA molecule and the broken DNA molecule. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MKLIYTEMSY | SMTEILVNEA | RKAADQGYRV | FYIAPNSLSF | EKEREVLTLL | PERGTFSIIV |
| 70 | 80 | 90 | 100 | 110 | 120 |
| TRFVQMSRYF | TVESSPSKQH | LDDTTLAMIF | YRALMQLKPE | DLPSYGRLQN | NSVFIEQLVE |
| 130 | 140 | 150 | 160 | 170 | 180 |
| LYKELKNAQL | SVHDLTGLDH | PQKQEDLIKI | IELAETIMIQ | QDYNQDSPLQ | SFARAIKLGL |
| 190 | 200 | 210 | 220 | 230 | 240 |
| LNNQLSKTVI | VIDGFSRFSA | EEDYLLSLLN | NNCQEVIIGS | YVSQKAYQKS | FIKGNIYEAS |
| 250 | 260 | 270 | 280 | 290 | 300 |
| LHFLQDLAQK | YHIKPVFAIS | NQVFKPAFSR | LTQLFEATHD | FSQVDWQLQK | NDLDHFSLWQ |
| 310 | 320 | 330 | 340 | 350 | 360 |
| CHHQKEEIEH | VAKSIRQKLY | EGYRYKDILV | LLGDMDAYQL | QIGPIFDKFE | IPYYLGKAEP |
| 370 | 380 | 390 | 400 | 410 | 420 |
| MAAHPLVQFI | ESLERSQRYN | WRREDILNML | KSGLFGCFDD | SDIDRFEEYT | QFADIKGFTK |
| 430 | 440 | 450 | 460 | 470 | 480 |
| FSKPFTINSS | RQYPLDFLNE | MRQDIVLPLQ | ELFKSQKQLG | ASLVDKLILF | LKKIRLAENM |
| 490 | 500 | 510 | 520 | 530 | 540 |
| QGLAQSQLEV | EKNEEVWKRF | TDILTSFHHI | FGQEKLRLSD | CLALIKTGMK | SAQYRVVPAT |
| 550 | 560 | 570 | 580 | 590 | 600 |
| LDVVTIKSYD | LVQPHSKPFV | YAIGLTQSHF | PKQIHHSGLL | SDQERARINE | IRNYRHFDIA |
| 610 | 620 | 630 | 640 | 650 | 660 |
| SAENSKKNHQ | TALSLFNAAT | KELVLSVPTV | INETFDDLSP | YLKELINFGL | PLLDKGKNYL |
| 670 | 680 | 690 | 700 | 710 | 720 |
| SYDNSDIGNY | KALLSQIIAI | NRQDLIEMSD | QDKMFWTVVL | RYLRKQLRKQ | QLELPTSDYR |
| 730 | 740 | 750 | 760 | 770 | 780 |
| LSTKPLSKEV | IEVCFPKGIP | LKLSATALTV | FYNNQYNYFL | KYVLNLNKTE | SIHPDSRIHG |
| 790 | 800 | 810 | 820 | 830 | 840 |
| QYLHRVFERL | MKDHTQEPFD | NKLKQAIYHT | NQESFFQQVY | QDNAEAEYSL | AMLEDIVRST |
| 850 | 860 | 870 | 880 | 890 | 900 |
| APILQLNQNI | QVIDQEKNFQ | LDMGNEILVH | GIIDRIDQLS | DGSLGIVDYK | SSANQFDIGT |
| 910 | 920 | 930 | 940 | 950 | 960 |
| FYNGLSPQLV | TYLAALKQIA | PHDINQLFGA | MYLHLQDPKL | DLVTFKQIDN | TLVESIYKAL |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| TYKGIFSEVE | KEHLSTGAYQ | TKNALYSNDE | LETLLNYNKY | LYLKAAKHIK | KGHFLINPYT |
| 1030 | 1040 | 1050 | 1060 | 1070 | |
| SDGKTVQGDQ | LKAITRFEAD | LDMAQARRLV | TLPAKEKKEC | FLTLMRKESH | L |