Q03290
Gene name |
TFB3 (RIG2, YDR460W) |
Protein name |
RNA polymerase II transcription factor B subunit 3 |
Names |
RNA polymerase II transcription factor B 38 kDa subunit, RNA polymerase II transcription factor B p38 subunit |
Species |
Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) |
KEGG Pathway |
sce:YDR460W |
EC number |
|
Protein Class |
|
Descriptions
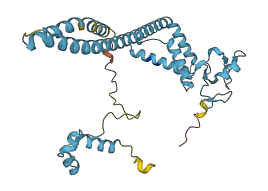
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
21 structures for Q03290
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| 5OQJ | EM | 470 A | 3 | 1-321 | PDB |
| 5OQM | EM | 580 A | 3 | 1-321 | PDB |
| 6GYM | EM | 670 A | 3 | 1-321 | PDB |
| 6XI8 | EM | 364 A | C | 259-321 | PDB |
| 7KUE | EM | 350 A | C | 1-321 | PDB |
| 7ML0 | EM | 300 A | 3 | 1-321 | PDB |
| 7ML1 | EM | 400 A | 3 | 1-321 | PDB |
| 7ML2 | EM | 340 A | 3 | 1-321 | PDB |
| 7ML3 | EM | 760 A | 3 | 1-321 | PDB |
| 7ML4 | EM | 310 A | 3 | 1-321 | PDB |
| 7O4I | EM | 320 A | 3 | 1-321 | PDB |
| 7O4J | EM | 290 A | 3 | 1-321 | PDB |
| 7O4K | EM | 360 A | 3 | 1-321 | PDB |
| 7O4L | EM | 340 A | 3 | 1-321 | PDB |
| 7O72 | EM | 340 A | 3 | 1-321 | PDB |
| 7O73 | EM | 340 A | 3 | 1-321 | PDB |
| 7O75 | EM | 320 A | 3 | 1-321 | PDB |
| 7ZS9 | EM | 310 A | 3 | 1-321 | PDB |
| 7ZSA | EM | 400 A | 3 | 1-321 | PDB |
| 7ZSB | EM | 660 A | 3 | 1-321 | PDB |
| AF-Q03290-F1 | Predicted | AlphaFoldDB |
2 variants for Q03290
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| s04-1383981 | 60 | D>G | No | SGRP | |
| s04-1384505 | 235 | K>Q | No | SGRP |
No associated diseases with Q03290
2 GO annotations of cellular component
| Name | Definition |
|---|---|
| transcription factor TFIIH holo complex | A complex that is capable of kinase activity directed towards the C-terminal Domain (CTD) of the largest subunit of RNA polymerase II and is essential for initiation at RNA polymerase II promoters in vitro. It is composed of the core TFIIH complex and the TFIIK complex. |
| transcription factor TFIIK complex | A transcription factor complex that forms part of the holo TFIIH complex. In Saccharomyces/human, TFIIK contains Ccl1p/Cyclin H, Tfb3p/MAT1 and Kin28p/CDK7. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| cyclin-dependent protein serine/threonine kinase activator activity | Binds to and increases the activity of a cyclin-dependent protein serine/threonine kinase. |
| metal ion binding | Binding to a metal ion. |
7 GO annotations of biological process
| Name | Definition |
|---|---|
| DNA repair | The process of restoring DNA after damage. Genomes are subject to damage by chemical and physical agents in the environment (e.g. UV and ionizing radiations, chemical mutagens, fungal and bacterial toxins, etc.) and by free radicals or alkylating agents endogenously generated in metabolism. DNA is also damaged because of errors during its replication. A variety of different DNA repair pathways have been reported that include direct reversal, base excision repair, nucleotide excision repair, photoreactivation, bypass, double-strand break repair pathway, and mismatch repair pathway. |
| nucleotide-excision repair | A DNA repair process in which a small region of the strand surrounding the damage is removed from the DNA helix as an oligonucleotide. The small gap left in the DNA helix is filled in by the sequential action of DNA polymerase and DNA ligase. Nucleotide excision repair recognizes a wide range of substrates, including damage caused by UV irradiation (pyrimidine dimers and 6-4 photoproducts) and chemicals (intrastrand cross-links and bulky adducts). |
| phosphorylation of RNA polymerase II C-terminal domain | The process of introducing a phosphate group on to an amino acid residue in the C-terminal domain of RNA polymerase II. Typically, this occurs during the transcription cycle and results in production of an RNA polymerase II enzyme where the carboxy-terminal domain (CTD) of the largest subunit is extensively phosphorylated, often referred to as hyperphosphorylated or the II(0) form. Specific types of phosphorylation within the CTD are usually associated with specific regions of genes, though there are exceptions. The phosphorylation state regulates the association of specific complexes such as the capping enzyme or 3'-RNA processing machinery to the elongating RNA polymerase complex. |
| regulation of cyclin-dependent protein serine/threonine kinase activity | Any process that modulates the frequency, rate or extent of cyclin-dependent protein serine/threonine kinase activity. |
| regulation of transcription by RNA polymerase II | Any process that modulates the frequency, rate or extent of transcription mediated by RNA polymerase II. |
| transcription by RNA polymerase II | The synthesis of RNA from a DNA template by RNA polymerase II (RNAP II), originating at an RNA polymerase II promoter. Includes transcription of messenger RNA (mRNA) and certain small nuclear RNAs (snRNAs). |
| transcription initiation at RNA polymerase II promoter | A transcription initiation process that takes place at a RNA polymerase II gene promoter. Messenger RNAs (mRNA) genes, as well as some non-coding RNAs, are transcribed by RNA polymerase II. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MLMDEYEENK | DMCPICKTDR | YLSPDVKFLV | NPECYHRICE | SCVDRIFSLG | PAQCPYKGCD |
| 70 | 80 | 90 | 100 | 110 | 120 |
| KILRKNKFKT | QIFDDVEVEK | EVDIRKRVFN | VFNKTIDDFN | GDLVEYNKYL | EEVEDIIYKL |
| 130 | 140 | 150 | 160 | 170 | 180 |
| DHGIDVAKTE | EKLRTYEELN | KQLIMNNLER | SRTEIESFEQ | RQKFEKEMKL | KKRLLERQIE |
| 190 | 200 | 210 | 220 | 230 | 240 |
| EEERMNKEWT | KKEIVNRLST | TTQDINETIE | GVKNTVKLKK | SSARRKLEEL | NRVLKNNPYF |
| 250 | 260 | 270 | 280 | 290 | 300 |
| NSNVNVQNSR | LKDAVPFTPF | NGDREAHPRF | TLKGSVYNDP | FIKDLEHRKE | FIASGFNTNY |
| 310 | 320 | ||||
| AYERVLTEAF | MGLGCVISEE | L |