Q02725
Gene name |
VTC3 (PHM2, YPL019C) |
Protein name |
Vacuolar transporter chaperone 3 |
Names |
Phosphate metabolism protein 2 |
Species |
Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) |
KEGG Pathway |
sce:YPL019C |
EC number |
|
Protein Class |
|
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
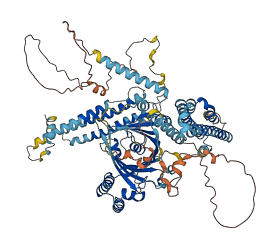
3 structures for Q02725
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| 7YTJ | EM | 300 A | E | 1-835 | PDB |
| 8I6V | EM | 306 A | D | 1-835 | PDB |
| AF-Q02725-F1 | Predicted | AlphaFoldDB |
22 variants for Q02725
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| s16-516980 | 13 | P>S | No | SGRP | |
| s16-516901 | 39 | S>N | No | SGRP | |
| s16-516887 | 44 | W>G | No | SGRP | |
| s16-516778 | 80 | D>G | No | SGRP | |
| s16-516677 | 114 | D>N | No | SGRP | |
| s16-516310 | 236 | V>A | No | SGRP | |
| s16-516281 | 246 | N>Y | No | SGRP | |
| s16-516275 | 248 | E>K | No | SGRP | |
| s16-516256 | 254 | Q>L | No | SGRP | |
| s16-516189 | 276 | Q>H | No | SGRP | |
| s16-516170 | 283 | S>T | No | SGRP | |
| s16-515835 | 394 | E>D | No | SGRP | |
| s16-515714 | 435 | I>V | No | SGRP | |
| s16-515533 | 495 | K>R | No | SGRP | |
| s16-515509 | 503 | Q>R | No | SGRP | |
| s16-515493 | 508 | E>D | No | SGRP | |
| s16-515219 | 600 | E>K | No | SGRP | |
| s16-515194 | 608 | N>S | No | SGRP | |
| s16-515183 | 612 | V>I | No | SGRP | |
| s16-514988 | 677 | P>S | No | SGRP | |
| s16-514728 | 763 | L>F | No | SGRP | |
| s16-514726 | 764 | T>I | No | SGRP |
No associated diseases with Q02725
Functions
6 GO annotations of cellular component
| Name | Definition |
|---|---|
| autophagosome membrane | The lipid bilayer surrounding an autophagosome, a double-membrane-bounded vesicle in which endogenous cellular material is sequestered. |
| endoplasmic reticulum | The irregular network of unit membranes, visible only by electron microscopy, that occurs in the cytoplasm of many eukaryotic cells. The membranes form a complex meshwork of tubular channels, which are often expanded into slitlike cavities called cisternae. The ER takes two forms, rough (or granular), with ribosomes adhering to the outer surface, and smooth (with no ribosomes attached). |
| fungal-type vacuole membrane | The lipid bilayer surrounding a vacuole, the shape of which correlates with cell cycle phase. The membrane separates its contents from the cytoplasm of the cell. An example of this structure is found in Saccharomyces cerevisiae. |
| integral component of membrane | The component of a membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
| membrane | A lipid bilayer along with all the proteins and protein complexes embedded in it an attached to it. |
| vacuolar transporter chaperone complex | A protein complex that contains four related proteins that have been implicated in several membrane-related processes, such as sorting of H+-translocating ATPases, endocytosis, ER-Golgi trafficking, vacuole fusion, vacuolar polyphosphate homeostasis and the microautophagic scission of vesicles into the vacuolar lumen. The complex is enriched at the vacuolar membrane, but also found in other cellular compartments, including the ER and the cell periphery. In Saccharomyces, the subunits are Vtc1p, Vtc2p, Vtc3p and Vtc4p. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| calmodulin binding | Binding to calmodulin, a calcium-binding protein with many roles, both in the calcium-bound and calcium-free states. |
| inositol hexakisphosphate binding | Binding to inositol hexakisphosphate. |
7 GO annotations of biological process
| Name | Definition |
|---|---|
| engulfment of target by autophagosome | The membrane invagination process by which an autophagosomal membrane surrounds an object that will be degraded by macroautophagy. |
| inositol phosphate-mediated signaling | A intracellular signal transduction in which the signal is transmitted within the cell via an inositol phosphate. Includes production of the inositol phosphate, and downstream effectors that further transmit the signal within the cell. Inositol phosphates are a group of mono- to poly-phosphorylated inositols, and include inositol monophosphate (IP), inositol trisphosphate (IP3), inositol pentakisphosphate (IP5) and inositol hexaphosphate (IP6). |
| lysosomal microautophagy | The transfer of cytosolic components into the lysosomal compartment by direct invagination of the lysosomal membrane without prior sequestration into an autophagosome. The engulfing membranes fuse, resulting in the lysosomal delivery of the cargo wrapped in a single membrane derived from the invaginated lysosomal membrane. In S. cerevisiae, the vacuole is the lysosomal compartment. |
| polyphosphate biosynthetic process | The chemical reactions and pathways resulting in the formation of a polyphosphate, the anion or salt of polyphosphoric acid. |
| polyphosphate metabolic process | The chemical reactions and pathways involving a polyphosphate, the anion or salt of polyphosphoric acid. |
| vacuolar transport | The directed movement of substances into, out of or within a vacuole. |
| vacuole fusion, non-autophagic | The fusion of two vacuole membranes to form a single vacuole. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MLFGIKLAND | VYPPWKDSYI | DYERLKKLLK | ESVIHDGRSS | VDSWSERNES | DFVEALDKEL |
| 70 | 80 | 90 | 100 | 110 | 120 |
| EKVYTFQISK | YNAVLRKLDD | LEENTKSAEK | IQKINSEQFK | NTLEECLDEA | QRLDNFDRLN |
| 130 | 140 | 150 | 160 | 170 | 180 |
| FTGFIKIVKK | HDKLHPNYPS | VKSLLQVRLK | ELPFNNSEEY | SPLLYRISYL | YEFLRSNYDH |
| 190 | 200 | 210 | 220 | 230 | 240 |
| PNTVSKSLAS | TSKLSHFSNL | EDASFKSYKF | WVHDDNIMEV | KARILRHLPA | LVYASVPNEN |
| 250 | 260 | 270 | 280 | 290 | 300 |
| DDFVDNLESD | VRVQPEARLN | IGSKSNSLSS | DGNSNQDVEI | GKSKSVIFPQ | SYDPTITTLY |
| 310 | 320 | 330 | 340 | 350 | 360 |
| FDNDFFDLYN | NRLLKISGAP | TLRLRWIGKL | LDKPDIFLEK | RTFTENTETG | NSSFEEIRLQ |
| 370 | 380 | 390 | 400 | 410 | 420 |
| MKAKFINNFI | FKNDPSYKNY | LINQLRERGT | QKEELEKLSR | DFDNIQNFIV | EEKLQPVLRA |
| 430 | 440 | 450 | 460 | 470 | 480 |
| TYNRTAFQIP | GDQSIRVTID | SNIMYIREDS | LDKNRPIRNP | ENWHRDDIDS | NIPNPLRFLR |
| 490 | 500 | 510 | 520 | 530 | 540 |
| AGEYSKFPYS | VMEIKVINQD | NSQMPNYEWI | KDLTNSHLVN | EVPKFSLYLQ | GVASLFGEDD |
| 550 | 560 | 570 | 580 | 590 | 600 |
| KYVNILPFWL | PDLETDIRKN | PQEAYEEEKK | TLQKQKSIHD | KLDNMRRLSK | ISVPDGKTTE |
| 610 | 620 | 630 | 640 | 650 | 660 |
| RQGQKDQNTR | HVIADLEDHE | SSDEEGTALP | KKSAVKKGKK | FKTNAAFLKI | LAGKNISENG |
| 670 | 680 | 690 | 700 | 710 | 720 |
| NDPYSDDTDS | ASSFQLPPGV | KKPVHLLKNA | GPVKVEAKVW | LANERTFNRW | LSVTTLLSVL |
| 730 | 740 | 750 | 760 | 770 | 780 |
| TFSIYNSVQK | AEFPQLADLL | AYVYFFLTLF | CGVWAYRTYL | KRLTLIKGRS | GKHLDAPVGP |
| 790 | 800 | 810 | 820 | 830 | |
| ILVAVVLIVT | LVVNFSVAFK | EAARRERGLV | NVSSQPSLPR | TLKPIQDFIF | NLVGE |