Q02158
Gene name |
plc (pipA, DDB_G0292736) |
Protein name |
1-phosphatidylinositol 4,5-bisphosphate phosphodiesterase |
Names |
Phosphoinositide phospholipase C, PLC |
Species |
Dictyostelium discoideum (Slime mold) |
KEGG Pathway |
ddi:DDB_G0292736 |
EC number |
3.1.4.11: Phosphoric diester hydrolases |
Protein Class |
|
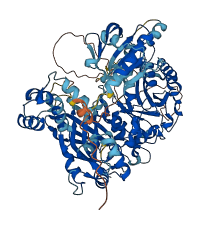
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for Q02158
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-Q02158-F1 | Predicted | AlphaFoldDB |
No variants for Q02158
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for Q02158 | |||||
No associated diseases with Q02158
Functions
| Description | ||
|---|---|---|
| EC Number | 3.1.4.11 | Phosphoric diester hydrolases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| membrane | A lipid bilayer along with all the proteins and protein complexes embedded in it an attached to it. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| calcium ion binding | Binding to a calcium ion (Ca2+). |
| phosphatidylinositol phospholipase C activity | Catalysis of the reaction: 1-phosphatidyl-1D-myo-inositol 4,5-bisphosphate + H(2)O = 1,2-diacylglycerol + 1D-myo-inositol 1,4,5-trisphosphate + H(+). |
8 GO annotations of biological process
| Name | Definition |
|---|---|
| establishment of protein localization | The directed movement of a protein to a specific location. |
| inositol trisphosphate biosynthetic process | The chemical reactions and pathways resulting in the formation of inositol trisphosphate, 1,2,3,4,5,6-cyclohexanehexol, with three phosphate groups attached. |
| lipid catabolic process | The chemical reactions and pathways resulting in the breakdown of lipids, compounds soluble in an organic solvent but not, or sparingly, in an aqueous solvent. |
| negative regulation of asexual reproduction | Any process that stops, prevents or reduces the frequency, rate or extent of asexual reproduction. |
| negative regulation of chemotaxis | Any process that stops, prevents, or reduces the frequency, rate or extent of the directed movement of a motile cell or organism in response to a specific chemical concentration gradient. |
| phosphatidylinositol-mediated signaling | The series of molecular signals in which a cell uses a phosphatidylinositol-mediated signaling to convert a signal into a response. Phosphatidylinositols include phosphatidylinositol (PtdIns) and its phosphorylated derivatives. |
| regulation of phagocytosis | Any process that modulates the frequency, rate or extent of phagocytosis, the process in which phagocytes engulf external particulate material. |
| sorocarp sorus development | The process whose specific outcome is the progression of the sorocarp sorus over time, from its formation to the mature structure. A sorocarp sorus is the spore containing structure of a sorocarp. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MDTLTNSQDY | SNVDLSLESL | AEELYNIQSF | NKDVILDSFD | IDDYDHTQLD | TTIDFNKFKI |
| 70 | 80 | 90 | 100 | 110 | 120 |
| GLTILKISSK | GKPQKKKLIF | DLARNQIVCG | KKKKVNFSEI | DEIRVGHKTN | IFNQFKSSKN |
| 130 | 140 | 150 | 160 | 170 | 180 |
| LKEDIESIQQ | SFSILFSGNL | RKTMDFVCSD | IPERRQIVSA | LYHVVQESKS | VNNEYNFVKR |
| 190 | 200 | 210 | 220 | 230 | 240 |
| EWDRVGKDSI | DFSTLKKILA | RLNFTTSDAV | LHNLMKFSDS | NSDYHLDFSE | FSNLLKLLRS |
| 250 | 260 | 270 | 280 | 290 | 300 |
| HPEMKPVFYK | YNGGNGEWVP | IQGMIDFFRI | EQSEVWTVEQ | CRDLIKKYHH | ERLDCISFEN |
| 310 | 320 | 330 | 340 | 350 | 360 |
| FEEFICGEAN | LAQYPHTSTV | YQDTSKPLSY | YFINSSHNTY | LSGHQLKGLS | TSEMYTNTLR |
| 370 | 380 | 390 | 400 | 410 | 420 |
| QGCKCVELDV | WDGNDGDPII | FHGNTLTSQI | KFSHVCETIK | ARGFETSPYP | VILSLEVHCS |
| 430 | 440 | 450 | 460 | 470 | 480 |
| VPQQIMMANH | MKEIFGEMLP | TPLPEGTKEL | PTLDSLKYKI | LLKGHTSHTH | VSAVGNSSAS |
| 490 | 500 | 510 | 520 | 530 | 540 |
| SSQSNIQTDD | NDDDGAVDLT | EYDEVDDRSA | SSSSSSFSLS | FGSSGKKKKI | TKIKIAPEFE |
| 550 | 560 | 570 | 580 | 590 | 600 |
| ELIYLVSHGF | KSGNTTKEIP | SYKIHSLVEE | KVKQLVQSEP | REVVEASQNH | LLRVYPRGTR |
| 610 | 620 | 630 | 640 | 650 | 660 |
| FDSSNFDPMP | GWSIGCQLAA | LNQQTSSEPM | WINDGMFSDN | GGCGYVLKPP | CLLPGECETY |
| 670 | 680 | 690 | 700 | 710 | 720 |
| DPTSPERIKS | SKYSRLIVNV | ISARQLPKYT | KSTKGEVIDP | YVTLSIVGTH | FDQKVEKTKV |
| 730 | 740 | 750 | 760 | 770 | 780 |
| IDNNGFNPHW | GEEFEFPLYN | SQLSMLLIRV | DDKDKVGHNR | IGHHCIRVEN | IRPGYRILKL |
| 790 | 800 | ||||
| KNNFNRTIPL | ANLLCKFTFV | E |