P50273
Gene name |
ATP22 (TCM10, YDR350C, D9476.9) |
Protein name |
Mitochondrial translation factor ATP22 |
Names |
|
Species |
Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) |
KEGG Pathway |
sce:YDR350C |
EC number |
|
Protein Class |
|
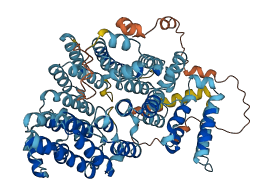
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for P50273
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-P50273-F1 | Predicted | AlphaFoldDB |
17 variants for P50273
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| s04-1178109 | 20 | P>R | No | SGRP | |
| s04-1178082 | 29 | G>E | No | SGRP | |
| s04-1178073 | 32 | T>K | No | SGRP | |
| s04-1178064 | 35 | P>H | No | SGRP | |
| s04-1178016 | 51 | I>S | No | SGRP | |
| s04-1177713 | 152 | G>D | No | SGRP | |
| s04-1177686 | 161 | H>R | No | SGRP | |
| s04-1177602 | 189 | R>K | No | SGRP | |
| s04-1177583 | 195 | I>M | No | SGRP | |
| s04-1177231 | 313 | G>R | No | SGRP | |
| s04-1176913 | 419 | T>A | No | SGRP | |
| s04-1176898 | 424 | A>S | No | SGRP | |
| s04-1176847 | 441 | G>R | No | SGRP | |
| s04-1176826 | 448 | I>V | No | SGRP | |
| s04-1176516 | 551 | H>R | No | SGRP | |
| s04-1176460 | 570 | V>L | No | SGRP | |
| s04-1176143 | 676 | I>V | No | SGRP |
No associated diseases with P50273
No regional properties for P50273
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| No domain, repeats, and functional sites for P50273 | |||
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| mitochondrial inner membrane | The inner, i.e. lumen-facing, lipid bilayer of the mitochondrial envelope. It is highly folded to form cristae. |
1 GO annotations of molecular function
| Name | Definition |
|---|---|
| translation regulator activity | Any molecular function involved in the initiation, activation, perpetuation, repression or termination of polypeptide synthesis at the ribosome. |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| positive regulation of mitochondrial translation | Any process that activates or increases the frequency, rate or extent of the chemical reactions and pathways resulting in the formation of proteins by the translation of mRNA in a mitochondrion. |
| proton-transporting two-sector ATPase complex assembly | The aggregation, arrangement and bonding together of a proton-transporting two-sector ATPase complex, a large protein complex that catalyzes the synthesis or hydrolysis of ATP by a rotational mechanism, coupled to the transport of protons across a membrane. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MLKCICRVYS | QPLAQMVTSP | LFKHMGSAGT | YTILPITNLR | HLSTKNCPLK | IKSNRSEPLQ |
| 70 | 80 | 90 | 100 | 110 | 120 |
| FGDFERQVPC | SRKSGSSKNV | QKRLYELRQL | KTVLSETFGV | TEYASFFESL | RNALHINNCS |
| 130 | 140 | 150 | 160 | 170 | 180 |
| ENEKKKLLYD | IILHQHELYP | EVARKIGFYL | PGEVHRWFWY | HIPKSESFNH | YLFLLKSDVL |
| 190 | 200 | 210 | 220 | 230 | 240 |
| LFTSNYCTRF | TNRLIKGTEM | ERQLATFQIF | LHDETNIKFI | MEKVLKLHTF | DSLIALVNGL |
| 250 | 260 | 270 | 280 | 290 | 300 |
| VKAKNFRFIK | VFIQALLQKL | EQHCYSGKDG | AKQKNLRYVK | FNNTLLYYLL | KSGNVELFIK |
| 310 | 320 | 330 | 340 | 350 | 360 |
| TFQEELKFIV | SSGLLNHIDG | NEHILNFPIH | HYLNLLRISN | RQEELFNVIS | CLQSSPLMKY |
| 370 | 380 | 390 | 400 | 410 | 420 |
| KLFKEFLMGE | LIASFQAFRD | PKLVCKYLLS | SYSSKASANI | LNALGIWGWL | YHSKSTTLTA |
| 430 | 440 | 450 | 460 | 470 | 480 |
| PTLARELKNK | NNILPNTMRI | GSPVTVPILT | ELYRSLLSSS | SVSLESGQFK | NCLLDLYYKY |
| 490 | 500 | 510 | 520 | 530 | 540 |
| KSFLSEEAHK | YRYWRNDTGI | LNVFLNYIRF | QAREPRLAYN | VLLDFYSQPF | AKKVVLTTTL |
| 550 | 560 | 570 | 580 | 590 | 600 |
| CPFSIVAYKN | HTLTQAELSE | LLQVMHKNGV | PLTFKFCSAM | VMHYVKMRDE | KGARSWYNKI |
| 610 | 620 | 630 | 640 | 650 | 660 |
| LFGGFEIRHM | ALIQIIKDQG | WPFPKNFDET | LLTELVENNN | IKEPTDSTLF | TDEDMFEEDG |
| 670 | 680 | ||||
| KPRFNDDDVN | KCTNIIRETL | KSLN |